Introduction
For decades, conventional agricultural management has led to a gradual impoverishment and simplification of agricultural landscapes, compromising the overall health of the most productive areas1. Since the 1950s, agricultural landscapes have been progressively stripped of the ecological infrastructure that for centuries had supported their ecological, productive, and cultural functions2. This has led to the disruption of the multiple relationships and self-regulation mechanisms within the agroecosystem, which has become a vulnerable and unstable system, highly dependent on external inputs to sustain its productive function3, unable to support other ecosystem functions across different scales – from soil domain, to the individual field, to the farming system, to the local landscape context and, more broadly, to the landscape unit4.
When considering the subset of peri-urban agricultural systems, these processes are further exacerbated. While urban systems confer numerous benefits to their inhabitants, they are also responsible for the profound alteration of the functioning of local and global ecosystems. This is achieved by the fragmentation and degradation of agricultural and natural habitats, leading to a reduction in biodiversity. Furthermore, urban systems disrupt hydrological systems, and modify energy flows and nutrient cycles. These dynamics, together with unsustainable land-use practices, affect agroecosystem functions and the provision of key ecosystem services (ES) on which the very livelihood of urban populations depends, e.g. supply of clean water, maintenance of soil fertility and health, food production, climate regulation and climate change mitigation, improvement of air quality5. Nonetheless, peri-urban fringe areas - ecotonal zones where the thinning of the urban fabric gradually gives way to natural, forestry, and pastoral land uses - hold considerable potential for providing buffering and resilience functions for cities6–11.
Soil health is increasingly recognized as a cornerstone of the broader concept of Global Health, as it underpins agricultural productivity, ecosystem services, human nutrition, and climate resilience. This complexity requires the development of composite indicators that are rapid, sensitive, and reliable in capturing the multifunctionality of soils. Many recent papers explicitly call for harmonized methodologies able to link soil health assessment with food security, biodiversity, and climate policies12–15. In this perspective, soil health indicators should not only measure physical and chemical properties, but also integrate biological and functional dimensions, thereby providing a comprehensive and policy-relevant assessment tool.
To address these challenges, it is therefore necessary to rethink the territorial development of peri-urban fringes in order to maximize their delivering capacity of ES, enhancing their capacity to mitigate the negative externalities of urban systems. Recent advances in the literature highlight the potential of silvoarable agroforestry systems (SAFs) as a strategy to counteract soil degradation and biodiversity loss in Western Europe. According to 16, SAFs contribute to soil biological health by fostering richer and more diverse soil communities and improving soil organic matter, litter-feeding macrofauna, and arbuscular mycorrhizal fungi, while also reducing soil bulk density. These effects are most pronounced in older stands and in proximity to tree rows, underscoring the role of temporal and spatial factors in shaping belowground processes. Despite these benefits, important research gaps remain—particularly concerning mesofauna, microbial activity, young stands, and deeper soil layers—indicating the need for more integrative indices that combine multiple biological parameters. Incorporating such findings into the broader context of sustainable land management underscores SAFs as a promising practice to enhance ecosystem services and soil resilience under climate and agricultural pressures.
In this contest, in the present study we investigated soil health using different indicators and performing a deep data analysis of different land uses representative of typical northern Italy peri-urban agricultural landscapes, i.e field annual crops, agroforestry, wooded areas, set-aside fields.
Results
Community composition and diversity patterns
To characterise differences in soil communities across land-use types, we analysed the taxonomic composition, richness, and diversity of fungal and bacterial communities, and quantified the overlap in species occurrence among land uses. Heatmap visualisation of the 25 most abundant fungal and bacterial genera revealed clear differences in taxonomic profiles among the four land-use types (Figure 1). Fungal communities showed stronger variation in dominant genera across land uses than bacterial communities, with certain genera significantly more abundant in specific samples and in specific land-use types. In contrast, the relative abundance in bacterial profiles displayed a higher homogeneity among samples, although clustering within the same land-use type is still visible to a certain degree. In general, fungal samples were dominated by genera such as Mortierella, Fusarium, and Trebouxia, while bacterial communities showed high relative abundances of members of the Acidobacteria group, Gemmatimonas and Gaiella. It is worth noting that in both fungal and bacterial datasets, some of the most abundant features were not fully resolved to genus level, suggesting the presence of a substantial fraction of community members that remain taxonomically undercharacterised. These results underline the stronger sensitivity of fungal communities to land-use and land-use change, probably due to their symbiotic associations with plants and strong linkage with organic matter, namely lignin and complex organic molecules and undisturbed conditions17. From an agroecological point of view, this results clearly demonstrate the role of agronomical management that enhance soil organic inputs (e.g., manure, green mulch, compost application, agroforestry litterfall) in sustaining fungal diversity.
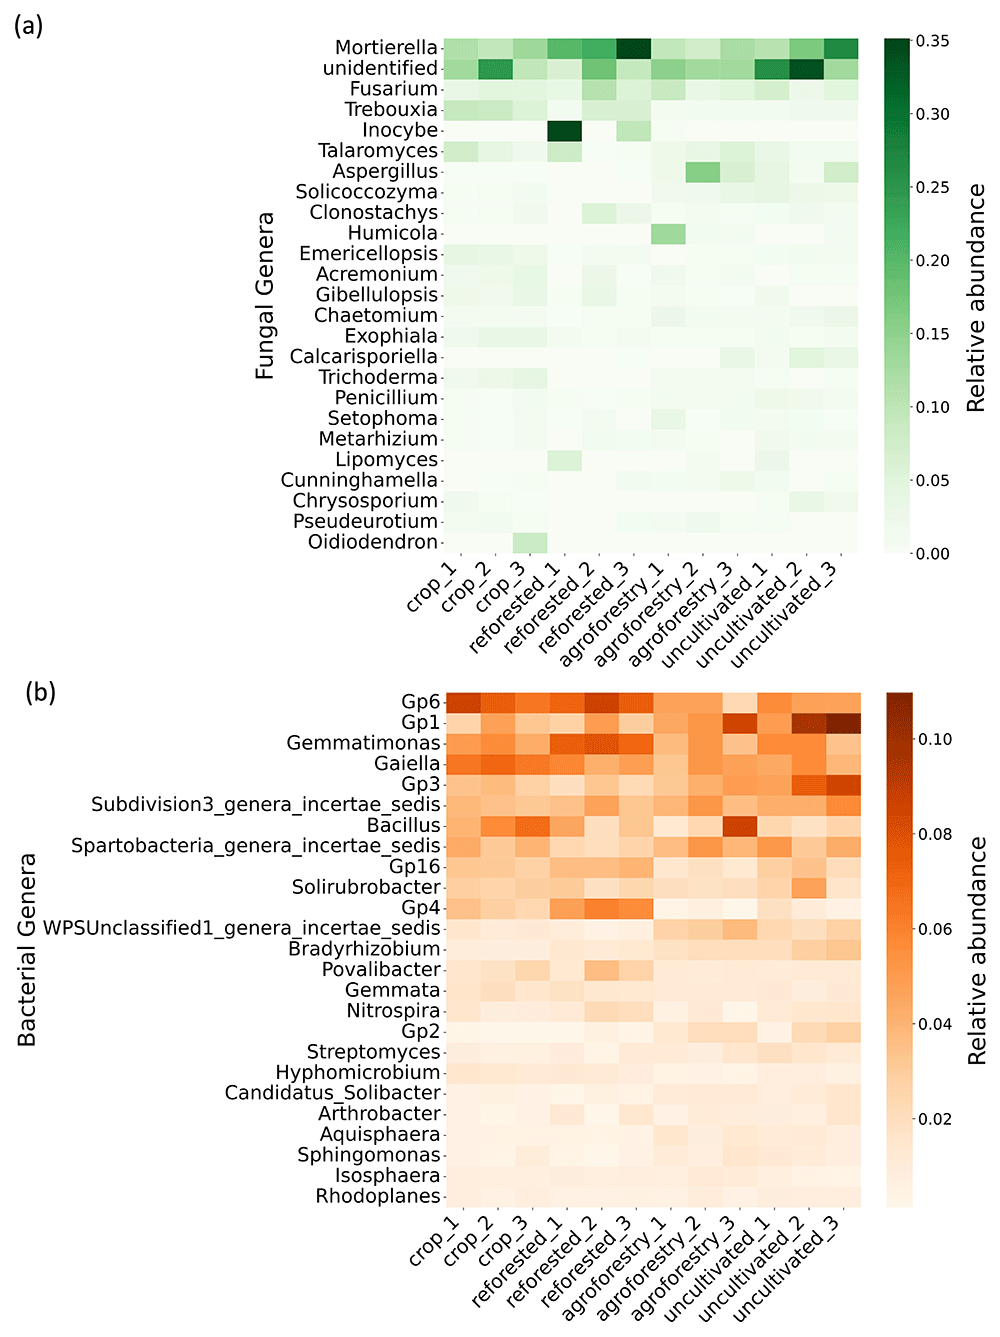
Figure 1.
Heatmaps of (a) the 25 most abundant fungal genera, and of (b) the 25 most abundant bacterial genera across 12 soil samples representing four land-use types (crop, reforested, agroforestry, and uncultivated). Genera are ordered by overall abundance. Color intensity reflects relative abundance within each sample.
Comparisons of diversity metrics at the species level showed that both fungal and bacterial richness and Shannon diversity varied noticeably across land-use types (Figure 2a). Uncultivated and reforested soils consistently exhibited lower richness than crop and agroforestry. However, due to the limited number of replicates for each land-use type (n=3), significant statistical differences were found only for richness: in bacteria, between crop and reforested soils; and in fungi, between crop and reforested soils as well as between reforested and agroforestry soils. Barplots showing patterns of richness and Shannon diversity across replicates are displayed in Figure 3, which confirms that the trends observed in the boxplots are consistent at the sample level.
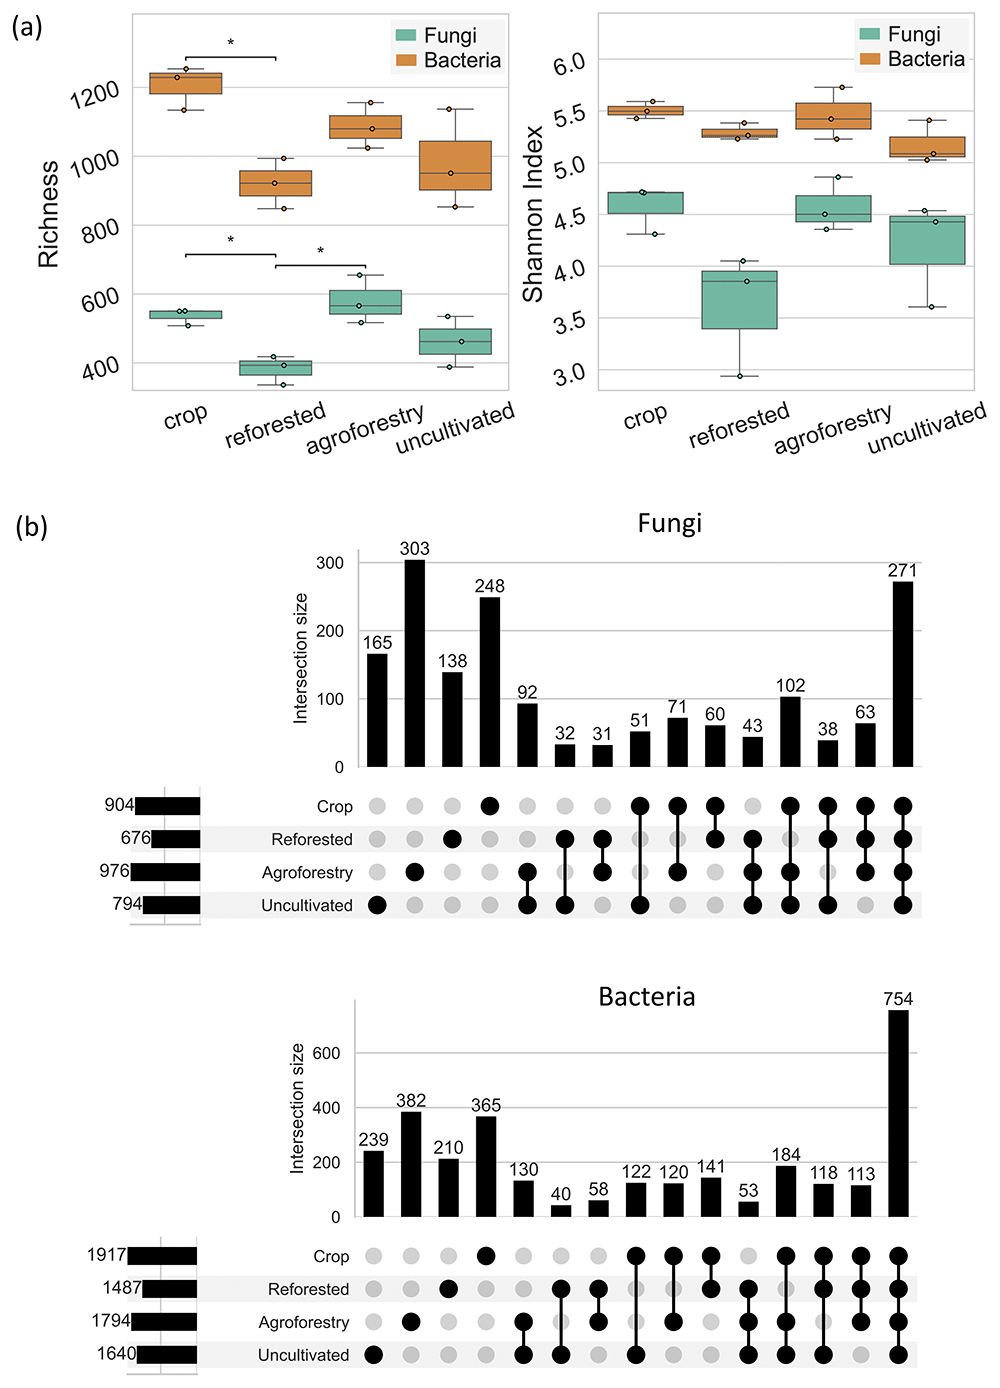
Figure 2.
(a) Boxplots of fungal and bacterial richness and Shannon’s diversity index at species level across different land uses. Significant differences between land-uses, assessed with a Tukey HSD test on the mean values of each ecological index, are indicated with a bar over the couple of boxplots and a number of stars. Differences are considered statistically significant at p-value < 0.05 and are reported with the following legend: 10−2 < p < 5 · 10−2 (*), 10−3 < p < 10−2 (**), 10−4 < p < 10−3 (***), p < 10−4 (****). (b) UpSet plots showing the intersection of bacterial and fungal species across four land use types. Each plot illustrates the number of species unique to or shared between different land uses. Horizontal bars represent the total number of species observed per land use, while the vertical bars show the size of species sets defined by each intersection.
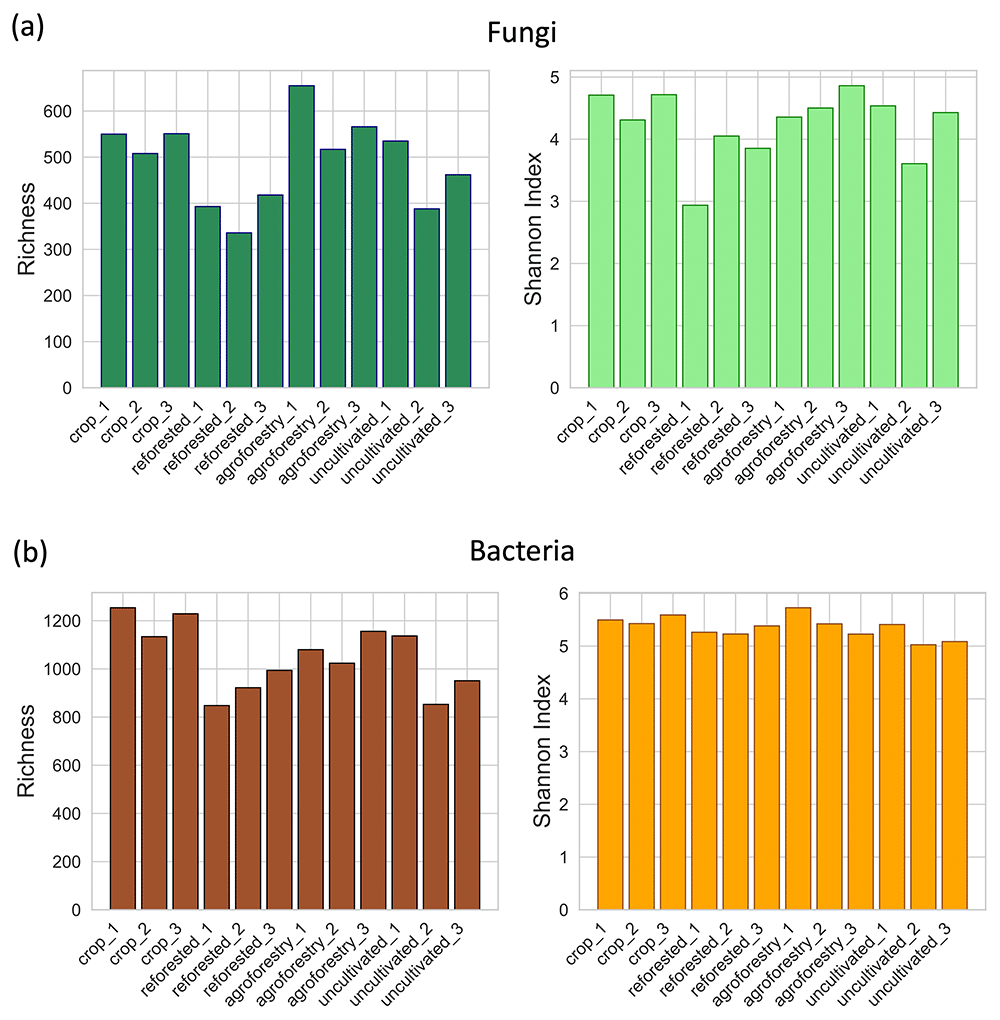
Figure 3. Ecological indices of fungal and bacterial communities across land-uses.
(a) Richness (left) and Shannon diversity index (right) for fungal communities in 12 soil samples. (b) Richness (left) and Shannon diversity index (right) for bacterial communities in the same samples. Each bar represents a replicate within one of four land-use categories: crop, reforested, agroforestry, and uncultivated.
UpSet plots of species presence–absence (Figure 2b) showed that a substantial proportion of fungal and bacterial taxa were unique to particular land-use types. Agroforestry soils feature the highest number of exclusive taxa for both fungi and bacteria, while reforested soils displayed the lowest number of unique species for both domains. These results indicate the agroecological function of agroforestry systems in terms of reservoirs of unique microbial taxa. Such diversification contributes to ecosystem resilience and multifunctionality, which are essential for effective biological pest control. Significant overlap in community composition was observed, especially in bacteria, with over 700 species common to all the land-use types. In addition to species-level differences, significant shifts were also observed at higher taxonomic ranks. Figure 4 and Figure 5 show fungal and bacterial phyla whose relative abundances varied significantly across land-use types, indicating that land-use effects are strong also at broader taxonomic groups. Notably, a larger number of bacterial phyla showed significant differences compared to fungi, likely reflecting the higher overall richness and taxonomic diversity of bacterial communities.
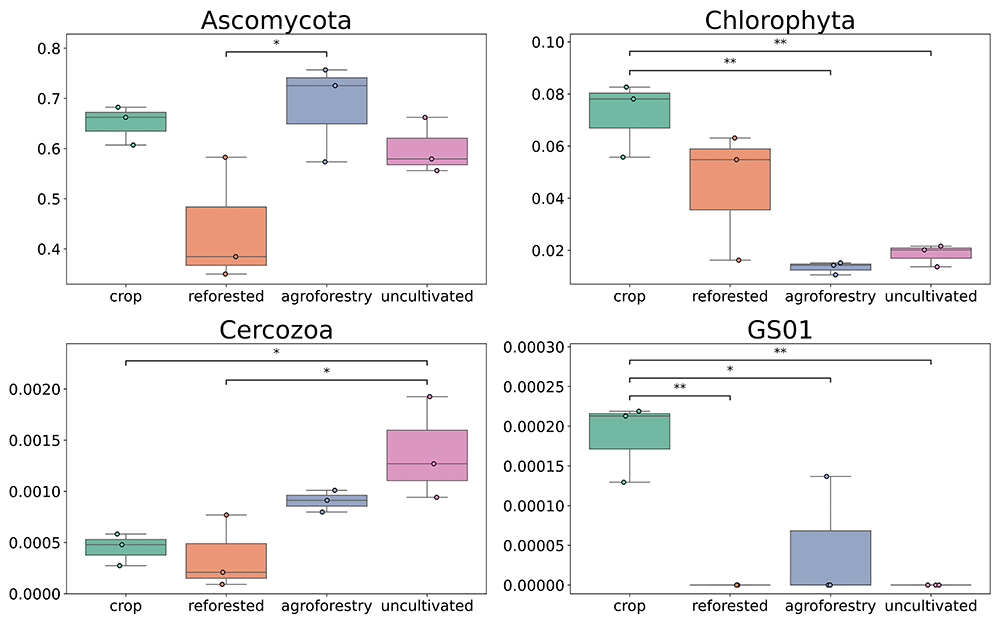
Figure 4. Boxplots of relative abundance of selected fungal genera across land-use types.
Only taxa with statistically significant differences (assessed with Tukey HSD test) are shown. Differences are considered statistically significant at p-value < 0.05 and are reported with the following legend: 10−2
< p < 5 · 10−2 (*), 10−3
< p < 10−2 (**), 10−4
< p < 10−3 (***), p < 10−4 (****).
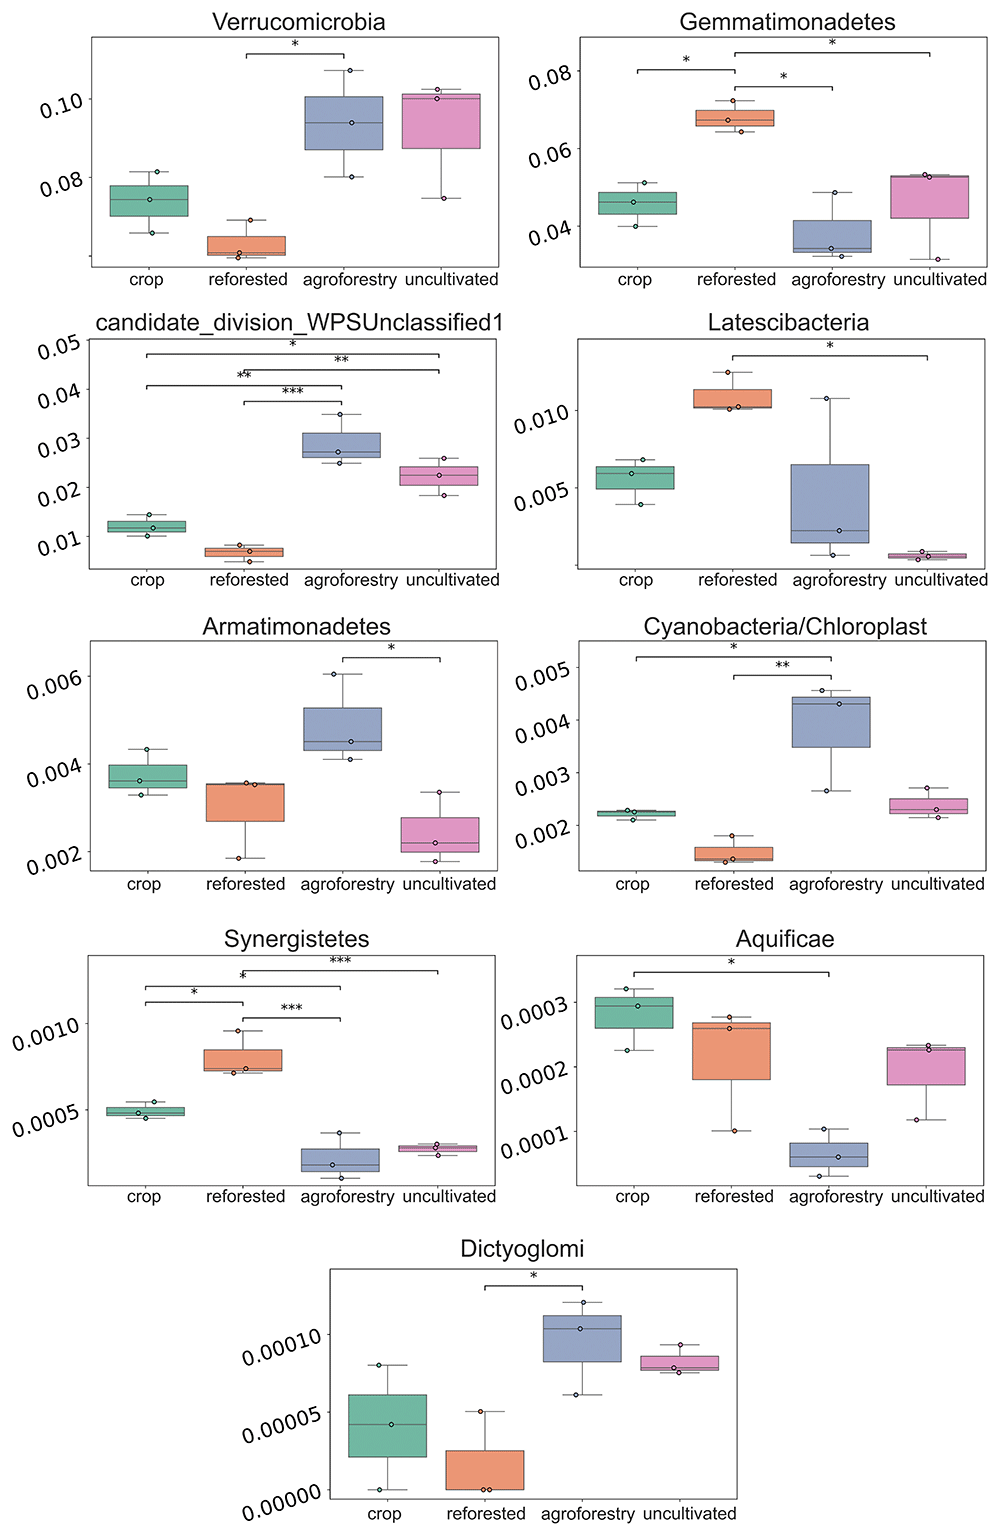
Figure 5. Boxplots of relative abundance of selected bacterial genera across land-use types.
Only taxa with statistically significant differences (assessed with Tukey HSD test) are shown. Differences are considered statistically significant at p-value < 0.05 and are reported with the following legend: 10−2 < p < 5 · 10−2 (*), 10−3 < p < 10−2 (**), 10−4 < p < 10−3 (***), p < 10−4 (****).
Correlation patterns among samples and abiotic parameters
To explore similarities among samples, we computed Pearson correlation matrices based on the bacterial, fungal and abiotic profiles of each sample; correlation matrices were represented as clustered heatmaps (Figure 6). In all three cases, samples sharing the same land-use tend to cluster; bacterial communities were more strongly clustered by land use than fungal communities, with two clear clusters formed by crop-reforested and uncultivated-agroforestry samples.
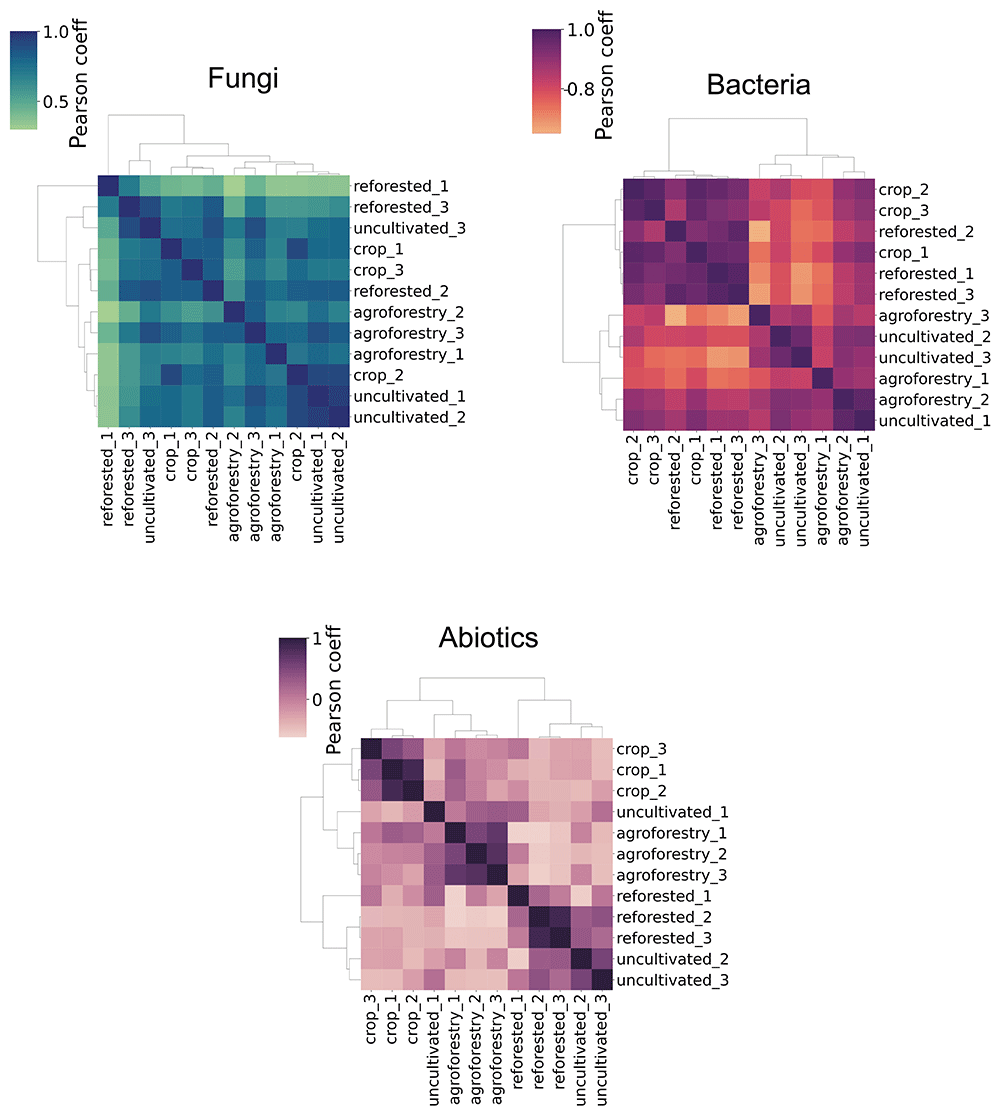
Figure 6. Heatmaps of pairwise Pearson correlations among samples based on fungal, bacterial, and abiotic profiles.
Each panel displays hierarchical clustering of the 12 soil samples based on their correlations. Darker colors indicate stronger positive correlations.
Moreover, we computed the Pearson correlation matrices of the abiotic parameters to investigate relationships among chemical and physical soil properties. Analysis of the top 20 strongest pairwise correlations among abiotic variables (Figure 7) revealed different patterns across land-use types. While crop and reforested soils displayed compact and large clusters dominated by strong correlations among fertility-related variables (e.g., organic matter, total nitrogen, organic carbon), agroforestry and uncultivated soils exhibited more complex and heterogeneous clustering patterns. This structural complexity suggests that agronomic practices enhancing agroecosystem diversity (e.g., intercropping, crop rotations, integrating annuals and perennials, and minimising soil disturbance) may lead to increased soil stability compared to simplified cropping and farming systems. In these two land uses, several subgroups of variables emerged, leading to a higher structural complexity. The complete correlation matrices (showing all the correlations, not only the strongest ones) for the different land-use types are shown in Figure 9–Figure 12. These plots display patterns broadly consistent with those observed in the reduced correlation matrices.
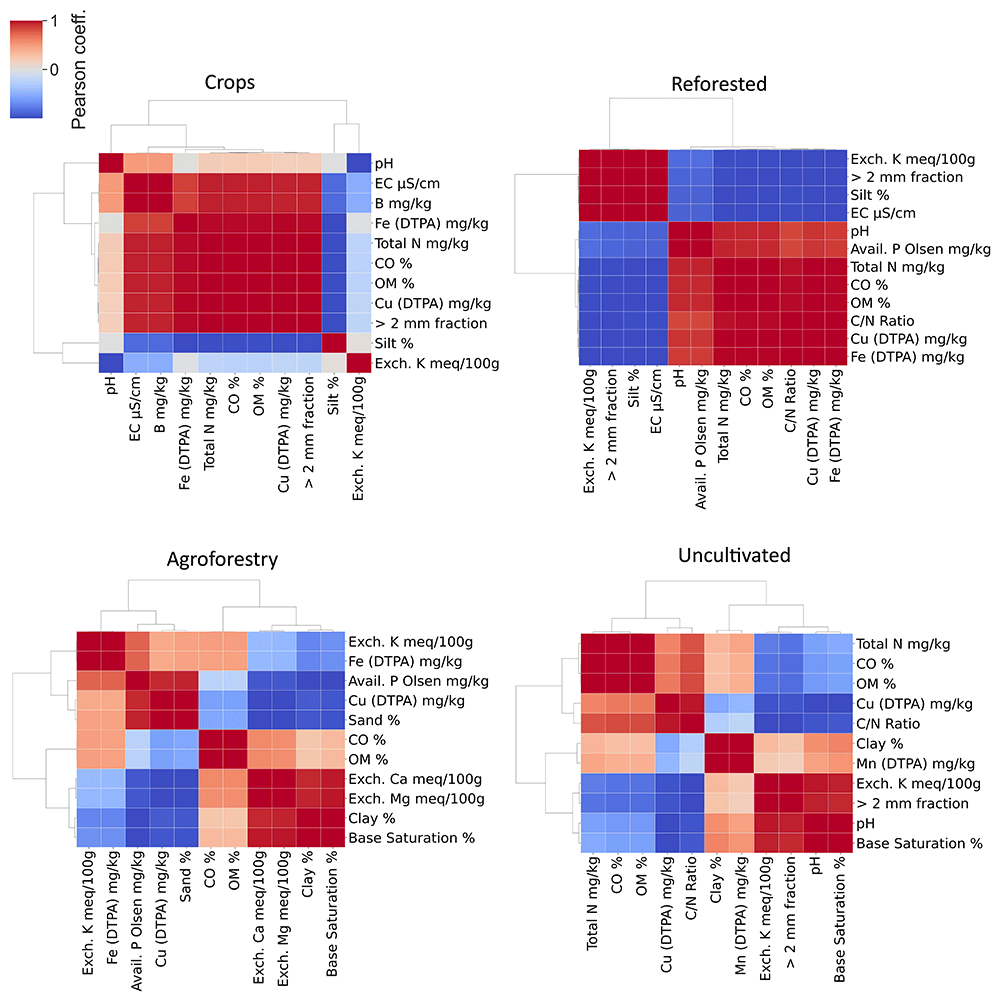
Figure 7. The figure displays a clustered heatmap of the top 20 strongest pairwise Pearson correlations (by absolute value) among abiotic variables.
Only variables involved in at least one of these top correlations were retained in the plot. The color scale represents the Pearson correlation coefficient.
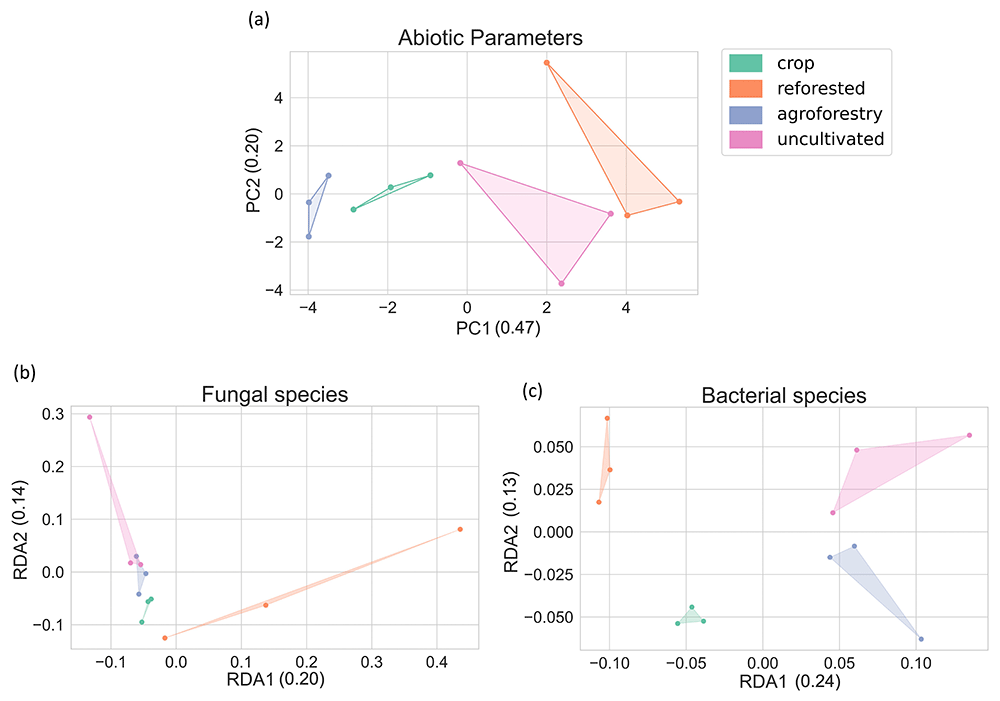
Figure 8. Ordination plots of abiotic and species data.
(a) Principal Component Analysis (PCA) of abiotic parameters across samples. (b) Redundancy Analysis (RDA) of fungal species constrained by selected abiotic variables. (c) Redundancy Analysis (RDA) of bacterial species constrained by selected abiotic variables. Convex hulls connect replicates within each land use group to visually highlight the clusters. The values between parentheses report the variance explained by each component.
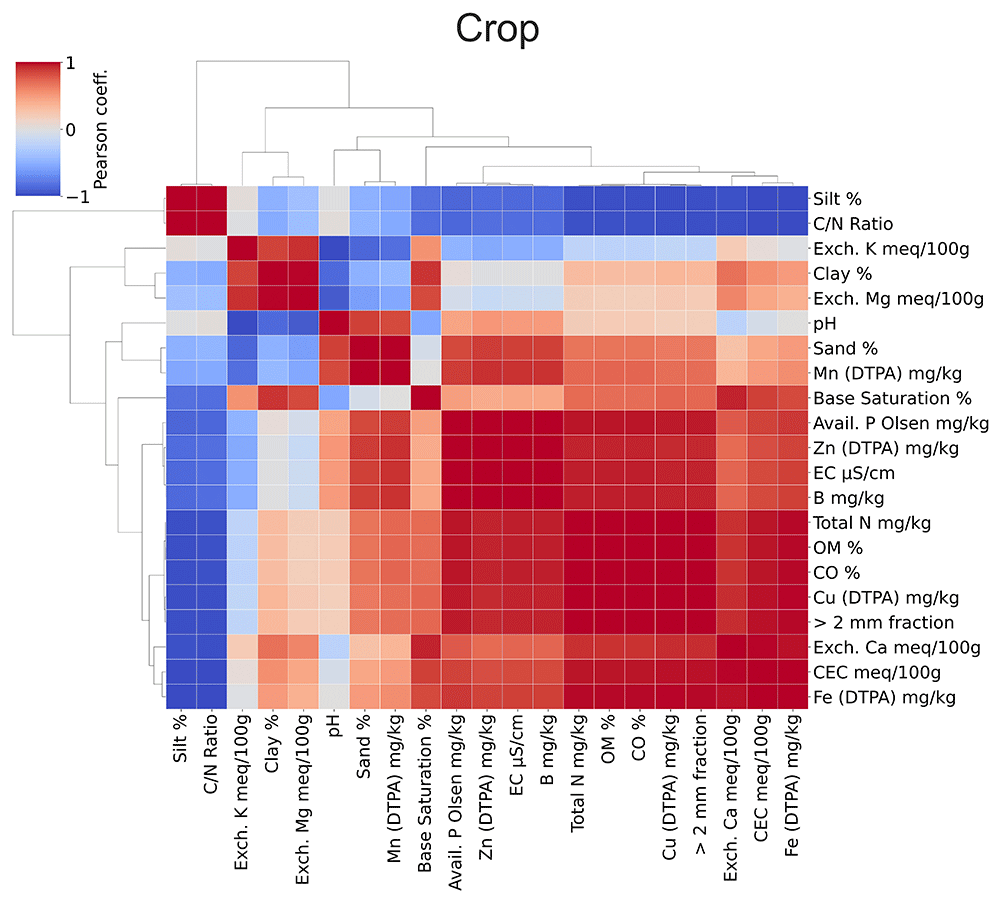
Figure 9. Heatmaps of pairwise Pearson correlations among abiotic parameters in Crop land-use.
Each panel displays hierarchical clustering of the abiotic parameters based on their correlations (for abbreviation key see Table 2). Darker colors indicate stronger positive correlations.
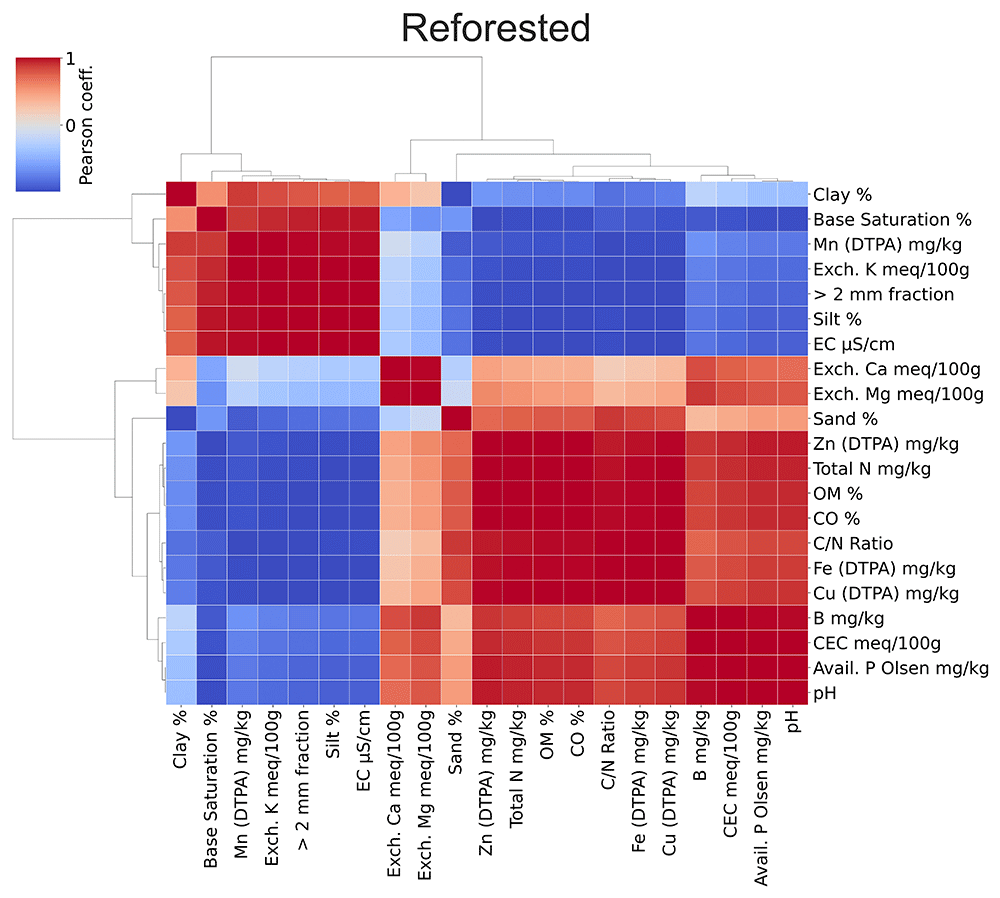
Figure 10. Heatmaps of pairwise Pearson correlations among abiotic parameters in Reforested land-use.
Each panel displays hierarchical clustering of the abiotic parameters based on their correlations (for abbreviation key see Table 2). Darker colors indicate stronger positive correlations.
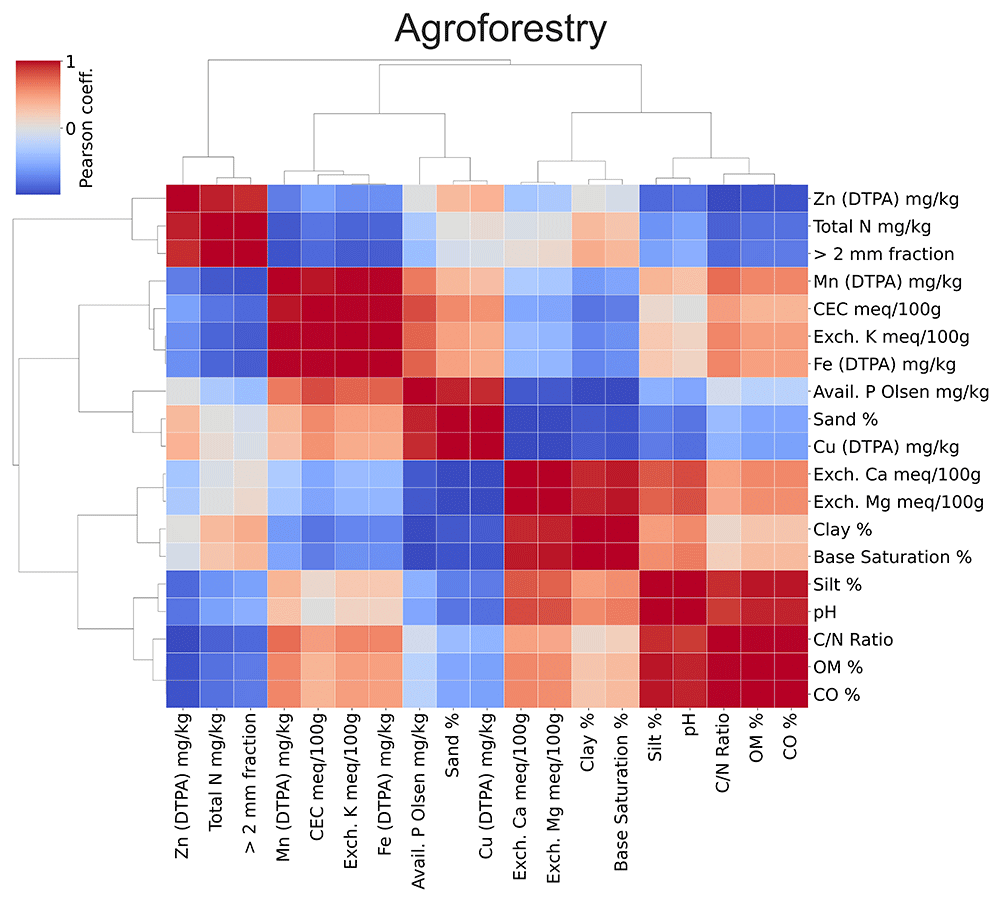
Figure 11. Heatmaps of pairwise Pearson correlations among abiotic parameters in Agroforestry land-use.
Each panel displays hierarchical clustering of the abiotic parameters based on their correlations (for abbreviation key see Table 2). Darker colors indicate stronger positive correlations.
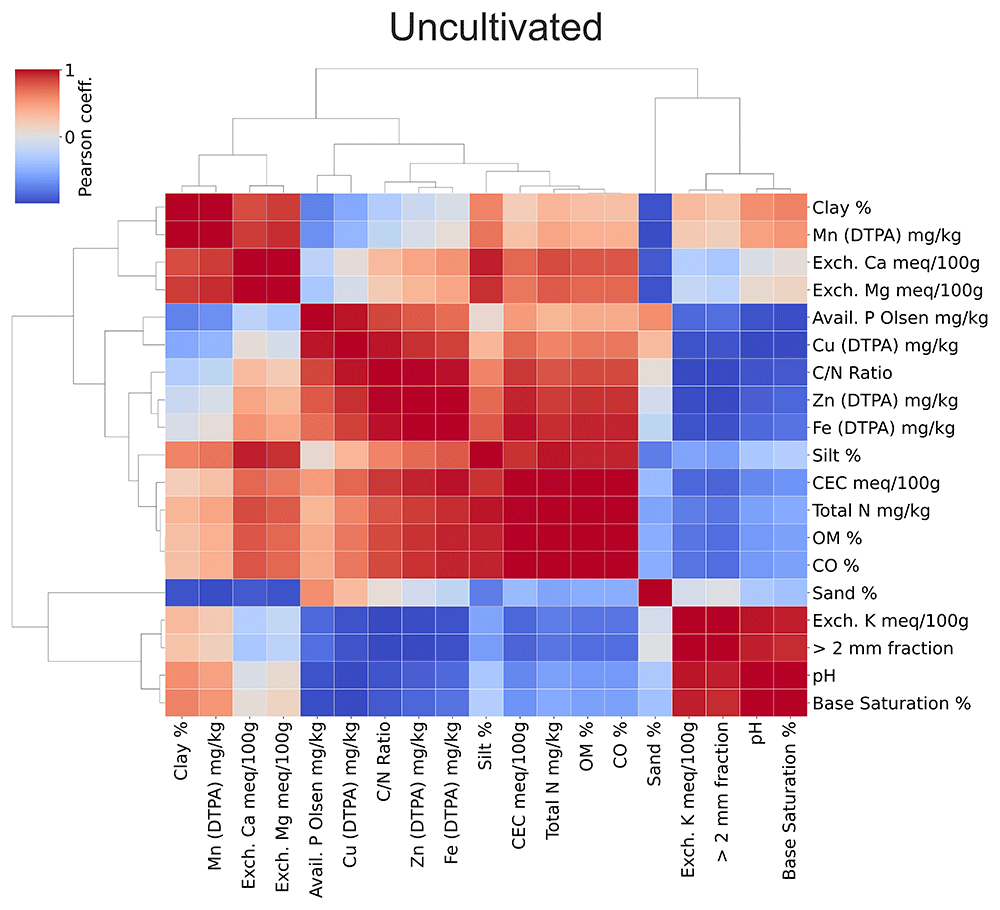
Figure 12. Heatmaps of pairwise Pearson correlations among abiotic parameters in Uncultivated land-use.
Each panel displays hierarchical clustering of the abiotic parameters based on their correlations (for abbreviation key see Table 2). Darker colors indicate stronger positive correlations.
We also assessed significant differences for each abiotic parameter across land-use types; the parameters showing the strongest effects are reported in Figure 13.
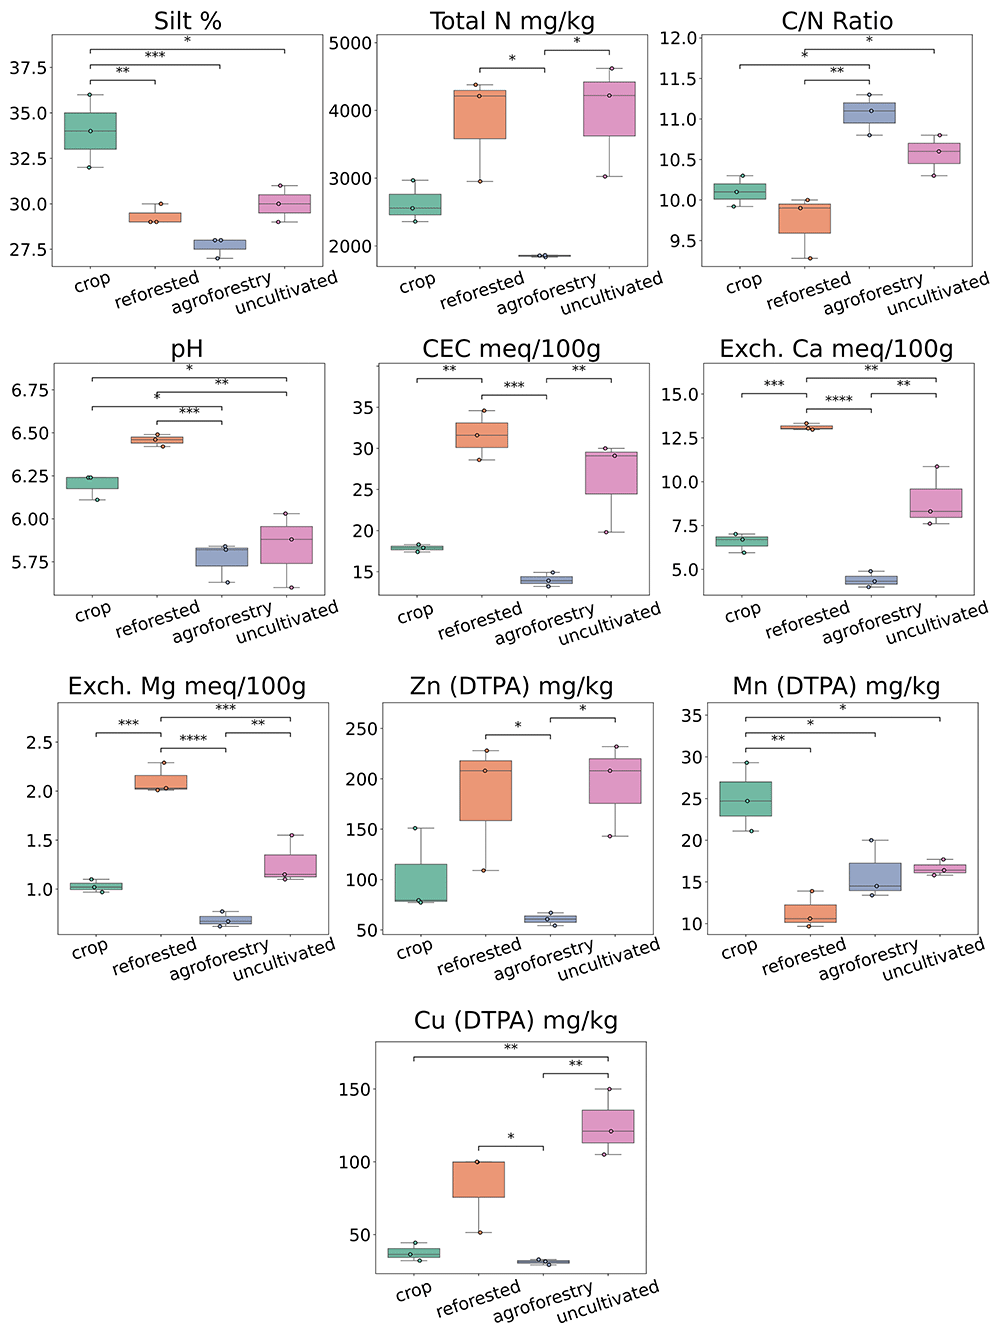
Figure 13. Boxplots of abiotic parameters across land-use types.
Only parameters with statistically significant differences (assessed with Tukey HSD test) are shown. Differences are considered statistically significant at p-value < 0.05 and are reported with the following legend: 10−2
< p < 5 · 10−2 (*), 10−3
< p < 10−2 (**), 10−4
< p < 10−3 (***), p < 10−4 (****). Abbreviation keys are reported in Table 2).
Multivariate analysis of soil communities and abiotic parameters
In order to assess how abiotic parameters shape microbial community structure, we performed ordination analyses. Principal Component Analysis (PCA) of abiotic variables (Figure 8a) explained a substantial fraction of variance in the first two components (> 60%) and showed clear separation of samples according to land use. Top abiotic contributors to the first principal component were Cation-Exchange Capacity, Total Nitrogen and Boron. These soil features are closely linked to the management of organic matter and organic carbon. Agronomic practices aimed at increasing organic inputs and enhancing specific nutrient cycles are crucial for positively shaping soil microbiomes.
Redundancy Analysis (RDA) of fungal and bacterial taxonomical profiles, where abiotic parameters were used as explanatory variables, confirmed significant associations between abiotic factors and soil community structure. The first 2 components of the RDA explained more than 30% of the variance, and both fungal and bacterial species were found to cluster in this 2-dimensional space, although this result is much more evident for bacteria.
Functional analysis of bacterial communities
To investigate whether land-use type influences microbial functional potential, we used PICRUSt2 to predict bacterial functional profiles; in particular, we computed Kyoto Encyclopedia of Genes and Genomes (KEGG) Orthology (KO) terms, Enzyme Commission (EC) numbers, and MetaCyc metabolic pathways for each land-use. Principal component analysis of these profiles consistently separated the different land-uses (Figure 14a–c), although uncultivated and agroforestry EC profiles partially overlap in the 2-dimensional space defined by the first 2 components of the PCA. We also created stacked bar plots of the 15 most abundant functions (Figure 14d–f) for each functional profile across the different land-uses. These stacked plots represent less or about 10% of the total predicted functional profile, indicating that the vast majority of detected functions occur at lower relative abundances. Moreover, the most prevalent functions displayed broadly similar relative abundances across land-use types, suggesting that a common set of core metabolic capacities dominates bacterial communities regardless of management regime.
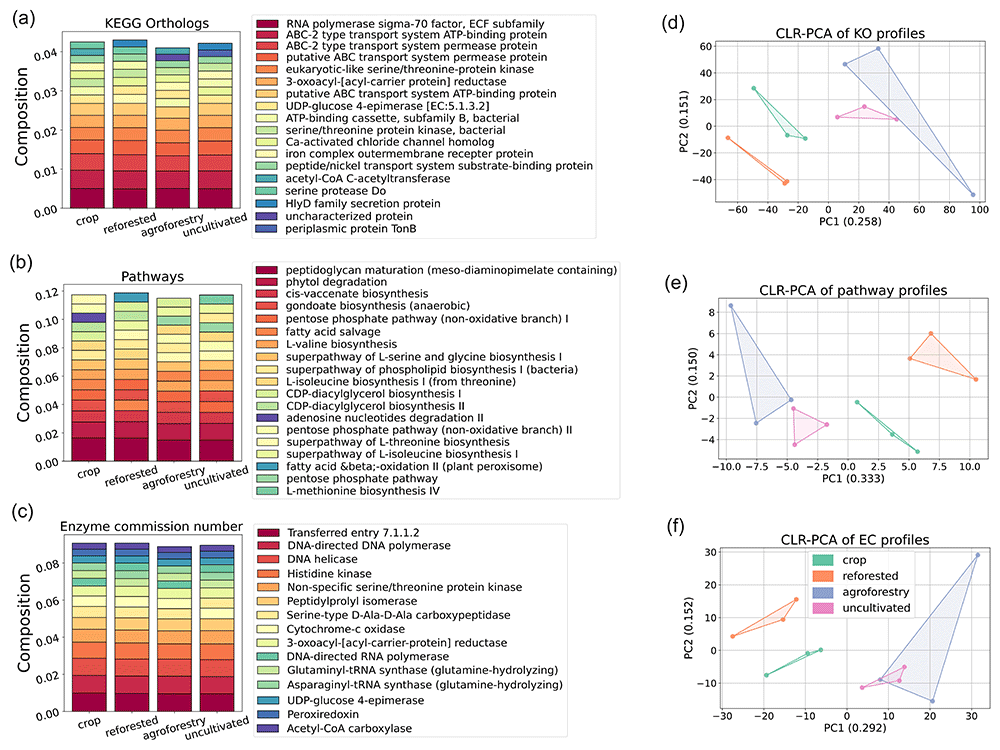
Figure 14.
(a)(b)(c) Stacked plots of the 15 most represented functions as expressed by KEGG, EC and MetaCyc metabolic pathways across land-use type. (d)(e)(f) Principal Component Analysis (PCA) of bacterial KEGG, EC and MetaCyc metabolic pathways functional profiles across land-use type, as obtained from PICRUSt2 analysis. Convex hulls connect replicates within each land use group to visually highlight the clusters. The values between parentheses report the variance explained by each component.
Methods
Study area
The study is applied to an agricultural area on the southeastern edge of the city of Milan (Figure 1), which has been the focus of recent strategic transformation plans aimed at establishing an agroecological experimentation laboratory18, integrated into the Living Lab Milano Porta Verde system19: an open-air laboratory dedicated to the socio-environmental regeneration of the area. The study area covers approximately 100 ha, part of the South Milan Agricultural Park - Vettabbia Valley system, an ancient strategic axis linking city and countryside20. The area is predominantly composed of agricultural lands (arable crops, horticulture, permanent and fallow grasslands) and semi-natural areas (young reforestation). Since 2019, the implementation of 2 ha under productive agroforestry management - a multilayered agro-silvo-pastoral system inspired by regenerative practices - has begun (Figure 1). The study area belongs to an alluvial context (Po Plain) dominated by Cambisols (WRB Classification System21), and Gleysols strips along water courses. A loamy-sandy texture predominates: loose and relatively permeable soils, easily workable, typical of alluvial contexts. Four land use types are investigated as treatments: crop field (crop), uncultivated area (uncultivated), wooded area (reforested), agroforestry system (agroforestry) (Table 1). Their selection was based on:
Table 1. Sampling sites main features.
| Land use type | Abbr. | Current
management | Current
management start date | Previous
land use | Products |
|---|
| Annual crop field | Crop | Conservation
agriculture | About 25 years
ago | Conventional
crop field | Corn (2–3 yrs)
in rotation with winter wheat (1 yr)
and soyabean (1 yr) |
| Wooded area | Reforested | Semi-natural | 2018 (planting) | Uncultivated
area | No products |
Agroforestry
system | Agroforestry | Regenerative
agriculture | 2019 (planting) | Conventional
crop field | Fruits, berries,
eggs |
Uncultivated
area | Uncultivated | Mowings | Stable for
decades | Crop field | Hay |
Table 2. Abiotic parameters: complete names and abbreviations used in figures.
| Abiotic parameter | Abbreviation |
|---|
| Sand % | Sand % |
| Clay % | Clay % |
| Silt % | Silt % |
| Total Nitrogen mg/kg | Total N mg/kg |
| C/N Ratio | C/N Ratio |
| Organic Matter % | OM % |
| OC % | OC % |
| Available Phosphorus Olsen mg/kg | Avail. P Olsen mk/kg |
| pH | pH |
| Electrical Conductivity (µS cm−1, 20°C) | EC µS/cm |
| Cation-Exchange Capacity meq 100g−1
| CEC meq 100g−1
|
| Base Saturation % | Base Saturation % |
| Exchangeable Calcium meq/100g | Exch. Ca meq/100g |
| Exchangeable Potassium meq/100g | Exch. K meq/100g |
| Exchangeable Magnesium meq/100g | Exch. Mg meq/100g |
| Zinc (DTPA) mg/kg | Zn (DTPA) mg/kg |
| Manganese (DPTA) mg/kg | Mn (DTPA) mg/kg |
| Iron (DTPA) mg/kg | Fe (DTPA) mg/kg |
| Boron (mg/kg) | B mg/kg |
| Copper (DTPA) mg/kg | Cu (DTPA) mg/kg |
| > 2 mm fraction | > 2 mm fraction |
• the intention to compare the agroforestry system with different local land uses, yet still of agro-silvo-pastoral or semi-natural type;
• the opportunity to compare sites characterized by the same pedological substrate (same cartographic Unit22).
In each site, sampling was conducted at selected nodes of an 8 × 8 grid with a 20 m mesh (Figure 15): four quadrants were set in the grid; in each of them one sampling point was identified, for a total of 3 soil sampling points for each site. Sampling points were selected to ensure an even distribution within the grid, avoiding marginal points, which often coincided with the edges of the site (roads, ditches, tree rows) and were more likely to be subject to disturbances that could influence the analytical results. Points that coincided with specific sources of heterogeneity within the site were also excluded, such as those located very close (< 2 m) to tree rows crossing the uncultivated area. The sampling was carried out by removing litter and picking soil slices through a spade at a depth of 0-30 cm with fixed thickness. Table 2 reports the soil parameters investigated.
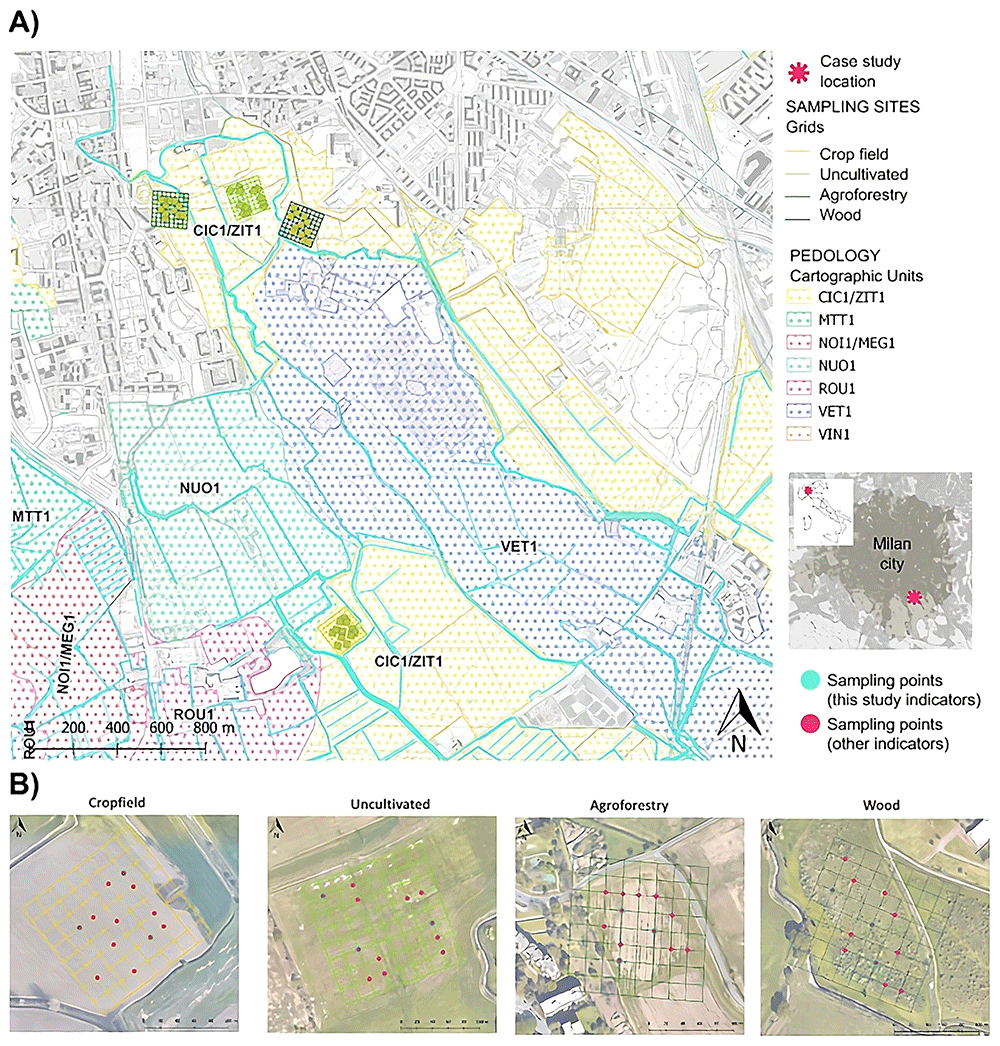
Figure 15.
a) The study area location in Milan metropolitan area and sampling sites location in CIC1/ZIT1 Soil Cartographic Unit - Cambisols; b) sampling sites location and sampling protocol.
Metagenomic sequencing library preparation, sequencing and analysis
The next generation sequencing experiments, which included quality control and the initial bioinformatics analysis, were executed by Genomix4life S.R.L. (Baronissi, Salerno, Italy). DNA quality control checks utilized the NanoDropOne spectrophotometer (Thermo Scientific, Waltham, MA, USA) and the Qubit Fluorometer 4.0 (Invitrogen Co., Carlsbad, CA, USA). 16S amplification was performed using primers targeting the hypervariable V3 and V4 region of the 16S rRNA gene (Forward: 5’-CCTACGGGNGGCWGCAG-3’; and Reverse: 5’-GACTACHVGGGTATCTAATCC-3’)23, while ITS amplification used the ITS3 – ITS4 primers (ITS3f 5’- GCATCGATGAAGAACGCAGC -3’ ITS4r: 5’-TCCTCCGCTTATTGATATGC -3’). Each Polymerase Chain Reaction (PCR) followed the protocol detailed in the Metagenomic Sequencing Library Preparation (Illumina, San Diego, CA, USA). A negative control, comprising all reagents used in 16S amplification and library preparation but excluding the sample, was incorporated into the workflow to ensure the absence of contamination. Libraries were quantified using a Qubit fluorometer (Invitrogen Co., Carlsbad, CA, USA) and then pooled to achieve an equimolar concentration of 4 nM for each index-tagged sample, with the inclusion of the Phix Control Library. The pooled samples underwent cluster generation and subsequent sequencing on the MiSeq platform (Illumina, San Diego, CA, USA) in a 2×250 paired-end format. Data analysis was carried out using the 16S Metagenomics pipeline (Illumina, San Diego, CA, USA). The RefSeq RDP 16S v3 database was sourced from: https://benjjneb.github.io/dada2/training.html. The UNITE Fungal ITS Database v7.2, which includes singletons set as RefS, was based on the FASTA release from December 1, 2017 https://doi.org/10.15156/BIO/587475.
Community diversity and taxonomical composition
Raw taxa abundances were first processed by normalizing the values for each sample to relative abundances (ranging from 0 to 1). To visualise the composition of the most common taxa at genus-level, we generated heatmaps showing the relative abundance of the 25 most abundant fungal and bacterial genera across the 12 soil samples.
To quantitatively assess the composition of soil communities, we calculated two metrics: observed richness (number of unique species) and Shannon diversity index.
These metrics were computed separately for fungal and bacterial taxa, based on species-level metagenomic assignments from each of the 12 soil samples.
Richness was defined as the count of distinct taxa detected per sample. The Shannon diversity index was calculated as:
where N is the number of observed taxa in a sample and pi is the relative abundance of the ith taxon. To visualise the ecological indices, we created barplots of richness and Shannon’s index across all 12 samples and boxplots across the different land-uses (crop, reforested, agroforestry, uncultivated), for both fungal and bacterial species. The ecological indices were computed using custom Python (v3.12.4) code, while the plots were created using the seaborn (v0.13.2) and matplotlib (v3.8.4) libraries.
To complement diversity and abundance-based metrics, we also assessed the overlap of microbial taxa across land-use types using UpSet plots24. These plots visualize the intersections of species sets and were created using the UpSetPlot (v0.9.0) package in Python.
Statistical analysis
To assess how soil communities and environmental parameters vary across different land-use types, we performed comparative analyses focusing on diversity metrics, taxonomic composition, and abiotic factors. The 12 soil samples were grouped according to their land-use classification: crop, reforested, agroforestry, and uncultivated (3 replicates per group).
Richness and Shannon diversity values and relative abundances of fungal and bacterial species were compared across land-use types using boxplots. Statistical differences were assessed via one-way ANOVA followed by Tukey’s Honest Significant Difference (HSD) post hoc test25. Significance was defined at p < 0.05. Given the large number of genera detected, only those exhibiting statistically significant differences between land-use types were visualized.
Abiotic soil parameters were compared across land-use types using the same procedure. Electrical conductivity (EC) and boron (B) included left-censored observations (reported as < 0.7µS/cm and < 0.5 mg/kg, respectively). These values were set at one-half the respective detection limit for the analysis. Again, we represented only the parameters where significant differences were found. All visualizations and tests were implemented using custom Python scripts with seaborn (v0.13.2), scipy (1.12.0), and statannotations (v0.7.1).
Correlation analysis
First, we assessed samples similarity computing pairwise Pearson correlation matrices among the 12 soil samples using three different variable sets: bacterial species abundances, fungal species abundances, and abiotic parameters. These correlation matrices were visualized as heatmaps paired with hierarchical clustering.
Moreover, to identify and visualize the strongest associations among abiotic soil parameters, we computed pairwise Pearson correlation coefficients using the full set of measured variables for each one of the four land-uses types. To reduce visual clutter, we implemented a filtering strategy to retain only the most strongly correlated variable pairs.
Specifically, we first computed the Pearson correlation matrix across all abiotic parameters, using the absolute values of the coefficients. We then ranked all unique variable pairs by the magnitude of their correlation coefficients and selected the top 20 strongest associations (excluding self-correlations). The set of variables involved in these top correlations was extracted, and a reduced correlation matrix was constructed using only this subset. This filtered matrix was visualized as a heatmap with hierarchical clustering.
This analysis was carried out using custom Python (v3.12.4) scripts, while the heatmaps were created using seaborn (v0.13.2) package.
Multivariate analysis
Before performing Multivariate Analysis, all variables were scaled to zero mean and unit variance using the StandardScaler function from the sklearn (v1.4.2) package. To reduce the dimensionality of the abiotic dataset and identify environmental gradients, we applied Principal Component Analysis (PCA) to the standardized abiotic parameters using the PCA function from sklearn (v1.4.2). The first two principal components were used to visualize the samples in reduced space, with samples colored by land-use type. Convex hulls were drawn around groups to highlight clustering by land use using the ConvexHulls function from scipy (v1.12.0).
To investigate the relationships between soil community composition and abiotic variables, we performed Redundancy Analysis (RDA) using species-level abundance data for fungi and bacteria as response matrices and a selected subset of abiotic parameters as explanatory variables. Because the number of abiotic variables exceeded the number of samples, we retained as explanatory variables only a selection of abiotic parameters. These were chosen as the top-contributing abiotic variables to the first principal component (PC1). In particular, we retained all the parameters whose linear coefficient describing PC1 were above 0.25: Cation Exchange Capacity (CEC) meq/100g, Total Nitrogen mg/kg, Boron mg/kg, Exchangeable Calcium, Zinc (DTPA) mg/kg, CO (%), Organic Matter and Exchangeable Magnesium meq/100g.
RDA was performed using the rda function from the scikit-bio (v0.6.3) package. We visualised the results with a scatter plot in the 2-dimensional space defined by the main components of the RDA using matplotlib (v3.8.4).
Functional analysis
Raw paired-end FASTQ files were processed in QIIME 226 (qiime2-amplicon-2025.7 version). Denoising, was performed with q2-dada2 (v2024.10.0) using denoise-paired. The produced amplicon sequence variant (ASV) feature table and representative sequences were used to predict functional profiles with PICRUSt227 (v2.4.1). In particular, we predicted Kyoto Encyclopedia of Genes and Genomes (KEGG)
Orthology (KO) terms, Enzyme Commission (EC) numbers, and MetaCyc metabolic pathways for each sample. These functional profiles were aggregated by land-use type; for each functional profile, we generated stacked bar plots showing the relative abundance of the 15 most prevalent functions across land uses. In addition, centered log-ratio (CLR) transformation was applied to each table (after compositional normalization), and principal component analysis (PCA) was performed to visualise patterns of functional differentiation among the four land-use categories. These exploratory analyses were conducted separately for KO, EC, and pathway profiles to compare the degree and structure of functional variation associated with land use.
Discussion
In the present study we investigated, in typical northern Italy peri-urban agricultural landscapes, how land use is able to influence soil microbial communities, abiotic soil parameters, and functional potentials. This kind of study is important to identify the best agroecological practice in peri-urban area able to preserve an healthy soil. In fact, it is known that the expanding urbanization affects biodiversity and agrobiodiversity, for example in a recent paper was discussed the complex relationship between these aspects also focusing to urban and peri-urban land for the best use in terms of biodiversity28.
Agroecological practices, included within the framework of Nature-Based Farming Solutions (e.g., landscape features, agroforestry), have the potential to activate and implement processes of diversification, ecological regeneration and multifunctional re-functionalization of rural areas29. In particular, agroforestry management, understood broadly as the management of productive and non-productive tree and shrub components, both within fields and along boundaries, such as hedgerows, tree lines, buffer strips, and small wooded patches30, is distinctive in its ability to interact with different levels of agroecosystem organization31.
Our results collectively suggest that agroforestry systems in spite of uncultivated, reforested and crop land use, can play a pivotal role in restoring soil health and enhancing EC, reinforcing their importance as nature-based solutions for sustainable land management. In fact, the observed differences in fungal and bacterial community composition across land-use types confirm that land management has a measurable impact on soil microbiota. Agroforestry soils were characterized by the highest number of unique taxa, whereas reforested soils showed the lowest richness and diversity, aligning with previous studies that highlight the early successional stage of reforestation systems32–34.
In a recent meta-analysis where was investigated the effects of agroforestry on ES provision in Europe35, was reported that, compared to conventional land uses such as pastures, arable crops, or forests, agroforestry supports higher levels of biodiversity and ecosystem goods and services. In this connection, the study by Beillouin et al.36 confirmed the capacity of agroforestry to significantly influence multiple ES, including biodiversity, production, water regulation and quality, pest and disease control, and soil quality.
Furthermore, we found that fungal communities had a stronger variation in dominant genera across land uses in comparison to bacterial communities. The predominance of Mortierella, Fusarium, and Trebouxia in fungal communities, as well as the dominance of Acidobacteria and Gemmatimonadetes in bacterial communities, underscores the potential of these taxa as bioindicators of soil health and management intensity. In fact, Mortierella is often found in the plant rhizosphere, where apparently that prevails in less disturbed soils with organic matter. Some studies have also indicated that Mortierella is associated with disease-suppressive soils. which goes with the accentuated complexity of undisturbed and diversified systems such as Silvoarable Agroforestry Systems (SAF)37–39. These symbioses are crucial for the nutrient cycle in forests and can play an important role in ecological succession processes. Considering the richness, that is the number of species present in each community, we found the highest level in land use for crops and agroforestry for both bacteria and fungi, while the Shannon index which considers the richness and evenness due to the limited number of replicates for each land use type confirm a great variety across land-use types but not significant. All together these analysis pointed out the deep impact of land use on the soil microbiome.
We then investigated how abiotic parameters such as for example cation-exchange capacity (CEC), total nitrogen, and boron, affect microbial communities. Multivariate analyses (PCA and RDA) revealed that abiotic parameters were key determinants of microbial community structure. This finding supports the hypothesis that soil fertility parameters not only reflect the chemical status of soils but also shape microbial niches and resource availability. Interestingly, agroforestry and uncultivated soils exhibited more heterogeneous clustering patterns of abiotic variables, suggesting a higher degree of spatial complexity and potentially greater resilience to disturbances. Functional predictions using PICRUSt2 indicated that while a core set of metabolic functions was shared across all land uses, agroforestry soils exhibited a broader functional repertoire. This functional diversification is consistent with the idea that agroforestry systems enhance ecological functions beyond productivity by providing microhabitats and diversified root exudates, as well as creating microhabitats that support a wider range of microbial guilds, thereby improving nutrient cycling and soil multifunctionality40,41. Our results provide evidence that management practices can influence not only who is present in the soil microbiome but also what functions they are capable of performing. This is aligned with the growing body of literature advocating agroforestry as a key tool in the ecological refunctionalization of rural and peri-urban landscapes42,43. By promoting biodiversity, improving soil structure, and enhancing carbon sequestration, agroforestry systems directly contribute to several Sustainable Development Goals (SDGs), including Zero Hunger (SDG 2), Climate Action (SDG 13), and Life on Land (SDG 15). The ES provided by agroforestry-managed soils include: soil conservation; soil health; carbon sequestration; nutrient cycling and enrichment; and the sequestration, transformation, and detoxification of chemicals into non-toxic forms. These benefits are difficult to measure independently, as they are interconnected. For example, increased carbon sequestration enhances soil nutrient status by improving cation exchange capacity, soil stability, and soil quality, while also reducing soil erosion44.
Overall, our study highlights the need for composite soil health indicators that integrate microbial, chemical, and physical parameters, as recommended by international frameworks such as the FAO’s Global Soil Partnership and the EU Soil Strategy for 2030. Despite the robustness of our findings, the limited number of replicates (n=3 per land-use type) constrains the statistical power of some comparisons, particularly for fungal communities where natural variability can be high. Future research should include temporal sampling to capture seasonal dynamics and longitudinal changes following management interventions.
Conclusion
Our findings show that land-use type has a significant impact on soil microbial communities, with agroforestry emerging as a promising agroecological practice. By increasing microbial diversity, supporting unique taxa, and broadening functional profiles, agroforestry can enhance ecosystem services, including nutrient cycling, carbon sequestration, and resilience to environmental stress. These findings support the incorporation of agroforestry into peri-urban agricultural landscapes as a strategy to balance food production with biodiversity conservation and climate regulation.
From a policy standpoint, this study emphasizes the importance of soil health indicators that incorporate biological aspects, as recommended by the FAO and the EU Soil Strategy 2030. Agroecological methods should be prioritized in land management frameworks to enhance soil ecosystem services and global health.
Ethics and consent
Ethical approval and consent were not required.
Data availability
UNIMI Dataverse. Replication Data for: Soil Health and Microbial Diversity Across Land-Use Types: Evidence for Agroecological Management in Peri-Urban Areas. https://dataverse.unimi.it/dataset.xhtml?persistentId=doi:10.13130/RD_UNIMI/ZGZY4Q45
This project contains the following underlying data:
16s Genus Level Aggregate Counts 2.csv: ITS OTU table at genus level ITS Species Level Aggregate Counts.csv: ITS OTU table at species level 16s Species Level Aggregate Counts.csv: 16s OTU table at species level ITS Genus Level Aggregate Counts.csv: 16s OTU table at genus level Samples.xlsx: metadata specifying the type of soil for each sample
Data is available under the terms of the CC BY 4.0 licence
Faculty Opinions recommendedReferences
- 1.
Millennium Ecosystem Assessment: Ecosystems and human well-being: wetlands and water synthesis. 2005. Reference Source
- 2.
Stoate C, Arau´jo M, Borralho R: Conservation of European farmland birds: abundance and species diversity.
Ornis Hungarica.
2003; 12(13): 33–40. Reference Source
- 3.
Gliessman SR, Rosado-May FJ, Guadarrama-Zugasti C, et al.: Agroecología: promoviendo una transición hacia la sostenibilidad.
Ecosistemas.
2007; 16(1): 13–23. Reference Source
- 4.
Ingegnoli V, et al.: Landscape bionomics biological-integrated landscape ecology. Springer, 2015. Publisher Full Text
- 5.
Borrelli P, Robinson DA, Fleischer LR, et al.: An assessment of the global impact of 21st century land use change on soil erosion.
Nat Commun.
2017; 8(1): 2013. PubMed Abstract
| Publisher Full Text
| Free Full Text
- 6.
Chiaffarelli G, Vagge I: Cities vs countryside: an example of a science-based peri-urban landscape features rehabilitation in Milan (Italy).
Urban For Urban Green.
2023; 86: 128002. Publisher Full Text
- 7.
Norman C, Surjan A, Booth M: Making resilience a reality: the contribution of peri-urban ecosystem services (BGI) to urban resilience. In: Ecosystem-Based disaster and climate resilience: integration of blue-green infrastructure in sustainable development. Springer, 2021; 185–200. Publisher Full Text
- 8.
Colucci A: Peri-urban/peri-rural areas: identities, values and strategies. In: Peri-Urban areas and food-energy-water nexus: sustainability and resilience strategies in the age of climate change. Springer, 2016; 99–104. Publisher Full Text
- 9.
Butt A: Sustainable, resilient, regenerative? The potential of melbourne’s peri-urban region.
Front Sustain Cities.
2024; 6: 1391712. Publisher Full Text
- 10.
Dal Borgo AG, Bocchi S, Capocefalo V, et al.: Agroforestry for the city: farmscaping the urban fringe through transformative and participatory action research in Milan.
Agroforest Syst.
2025; 99(5): 125. Publisher Full Text
- 11.
Dal Borgo AG, Chiaffarelli G, Capocefalo V, et al.:
Agroforestry as a driver for the provisioning of peri-urban socio-ecological functions: a trans-disciplinary approach.
Sustainability.
2023; 15(14): 11020. Publisher Full Text
- 12.
Erdogan HE, Havlicek E, Dazzi C, et al.:
Soil conservation and Sustainable Development Goals (SDGs) achievement in europe and central asia: which role for the European soil partnership?
International Soil and Water Conservation Research.
2021; 9(3): 360–369. Publisher Full Text
- 13.
Heuser I:
Soil governance in current European Union law and in the European green deal.
Soil Secur.
2022; 6: 100053. Publisher Full Text
- 14.
Panagos P, Montanarella L, Barbero M, et al.:
Soil priorities in the European Union.
Geoderma Reg.
2022; 29: e00510. Publisher Full Text
- 15.
Pereira P, Bogunovic I, Muñoz-Rojas M, et al.:
Soil ecosystem services, sustainability, valuation and management.
Curr Opin Environ Sci Health.
2018; 5: 7–13. Publisher Full Text
- 16.
De Clercq P, De Vroe A, Janssens P, et al.:
Effect of a soil water balance controlled irrigation on the cultivation of Acer pseudoplatanus forest Tree liners under non-limiting and limiting soil water conditions.
Horticulturae.
2025; 11(4): 435. Publisher Full Text
- 17.
Khan A, Rao TS:
Molecular evolution of xenobiotic degrading genes and mobile DNA elements in soil bacteria. In: Microbial Diversity in the Genomic Era. Elsevier, 2019; 657–678. Publisher Full Text
- 18.
Longo A:
Openagri – 18 progetti x 30 ettari: un masterplan per un parco della sperimentazione agroecologica. Workshop working document (wp7), Dipartimento DAStU, Politecnico di Milano; Dipartimento ABC Politecnico di Milano; Dipartimento ESP Universit`a degli Studi di Milano, Milano, Italia. Nell’ambito del progetto OpenAgri, bando europeo Urban Innovative Actions (UIA), 2018.
- 19.
LIAISON Consortium: Milano porta verde — European Rural Innovation Ambassador. Horizon 2020 project LIAISON, Grant Agreement No. 773418, 2020. Reference Source
- 20.
Prusicki M, et al.:
Area sud-milano. Uno scenario strategico di riqualificazione paesistica del basso milanese. In: LOTO Landscape Opportunities. La Gestione Paesistica delle Trasformazioni Territoriali. Complessit`a Territoriale e Valorizzazione del Paesaggio. Esperienze a Confronto in Lombardia, Regione Lombardia, 2006; 52–92.
- 21.
Costantini E, Dazzi C:
World Reference Base for Soil Resources. Base di riferimento mondiale per le risorse pedologiche. CRA-ABP, 1999. Reference Source
- 22.
ERSAF: Regional soil database Losan. 2008. Reference Source
- 23.
Klindworth A, Pruesse E, Schweer T, et al.:
Evaluation of general 16s ribosomal RNA gene PCR primers for classical and next-generation sequencing-based diversity studies.
Nucleic Acids Res.
2013; 41(1): e1. PubMed Abstract
| Publisher Full Text
| Free Full Text
- 24.
Lex A, Gehlenborg N, Strobelt H, et al.:
Upset: visualization of intersecting sets.
IEEE Trans Vis Comput Graph.
2014; 20(12): 1983–1992. PubMed Abstract
| Publisher Full Text
| Free Full Text
- 25.
Tukey JW:
Comparing individual means in the analysis of variance.
Biometrics.
1949; 5(2): 99–114. PubMed Abstract
- 26.
Bolyen E, Rideout JR, Dillon MR, et al.:
Reproducible, interactive, scalable and extensible microbiome data science using QIIME 2.
Nat Biotechnol.
2019; 37(8): 852–857. PubMed Abstract
| Publisher Full Text
| Free Full Text
- 27.
Douglas GM, Maffei VJ, Zaneveld JR, et al.:
PICRUSt2 for prediction of metagenome functions.
Nat Biotechnol.
2020; 38(6): 685–688. PubMed Abstract
| Publisher Full Text
| Free Full Text
- 28.
Zimmerer KS, Duvall CS, Jaenicke EC, et al.:
Urbanization and agrobiodiversity: leveraging a key nexus for sustainable development.
One Earth.
2021; 4(11): 1557–1568. Publisher Full Text
- 29.
Wezel A, Goris M, Bruil J, et al.:
Challenges and action points to amplify agroecology in Europe.
Sustainability.
2018; 10(5): 1598. Publisher Full Text
- 30.
Santiago-Freijanes JJ, Mosquera-Losada MR, Rois-Díaz M, et al.:
Global and European policies to foster agricultural sustainability: agroforestry.
Agroforest Syst.
2021; 95(5): 775–790. Publisher Full Text
- 31.
Montagnini F, Fierro S:
Functions of agroforestry systems as biodiversity Islands in productive landscapes. In: Biodiversity Islands: Strategies for Conservation in Human-dominated Environments. Springer, 2022; 89–116. Publisher Full Text
- 32.
Kong W, Wei X, Wu Y, et al.:
Afforestation can lower microbial diversity and functionality in deep soil layers in a semiarid region.
Glob Chang Biol.
2022; 28(20): 6086–6101. PubMed Abstract
| Publisher Full Text
- 33.
Beule L, Vaupel A, Moran-Rodas VE:
Abundance, diversity, and function of soil microorganisms in temperate alley-cropping agroforestry systems: a review.
Microorganisms.
2022; 10(3): 616. PubMed Abstract
| Publisher Full Text
| Free Full Text
- 34.
De Clerck C, Andrianarisoa KS, Lassois L, et al.:
Silvoarable agroforestry systems as promising practices for improving soil biological health: recent advances and future challenges in Western European region.
Soil Use Manag.
2025; 41(3): e70104. Publisher Full Text
- 35.
Torralba M, Fagerholm N, Burgess PJ, et al.:
Do European agroforestry systems enhance biodiversity and ecosystem services? A meta-analysis.
Agriculture, ecosystems & environment.
2016; 230: 150–161. Publisher Full Text
- 36.
Beillouin D, Ben-Ari T, Malézieux E, et al.:
Positive but variable effects of crop diversification on biodiversity and ecosystem services.
Glob Chang Biol.
2021; 27(19): 4697–4710. PubMed Abstract
| Publisher Full Text
- 37.
Siles JA, Vera A, Díaz-López M, et al.:
Land-use-and climate-mediated variations in soil bacterial and fungal biomass across Europe and their driving factors.
Geoderma.
2023; 434: 116474. Publisher Full Text
- 38.
Kim HS, Lee SH, Jo HY, et al.:
Diversity and composition of soil Acidobacteria and Proteobacteria communities as a bacterial indicator of past land-use change from forest to farmland.
Sci Total Environ.
2021; 797: 148944. PubMed Abstract
| Publisher Full Text
- 39.
Gossner MM, Lewinsohn TM, Kahl T, et al.:
Land-use intensification causes multitrophic homogenization of grassland communities.
Nature.
2016; 540(7632): 266–269. PubMed Abstract
| Publisher Full Text
- 40.
Ullah S, Han X, Ali I, et al.:
Ecological impacts of diversified agroforestry on soil nutrients and bacterial communities in pinus massoniana plantations in the southern subtropics.
Industrial Crops and Products.
2024; 222(Part 4): 119933. Publisher Full Text
- 41.
Soliveres S, Van Der Plas F, Manning P, et al.:
Biodiversity at multiple trophic levels is needed for ecosystem multifunctionality.
Nature.
2016; 536(7617): 456–459. PubMed Abstract
| Publisher Full Text
- 42.
Castle SE, Miller DC, Merten N, et al.:
Evidence for the impacts of agroforestry on ecosystem services and human well-being in high-income countries: a systematic map.
Environ Evid.
2022; 11(1): 10. PubMed Abstract
| Publisher Full Text
| Free Full Text
- 43.
Jose S:
Agroforestry for ecosystem services and environmental benefits: an overview.
Agroforest Syst.
2009; 76(1): 1–10. Publisher Full Text
- 44.
Udawatta RP, Rankoth LM, Jose S:
Agroforestry and biodiversity.
Sustainability.
2019; 11(10): 2879. Publisher Full Text
- 45.
Replication Data For: Soil Health and Microbial Diversity Across Land-Use Types: Evidence for Agroecological Management in Peri-Urban Areas. http://www.doi.org/10.13130/RD_UNIMI/ZGZY4Q