1. Introduction
Olive cultivation is a cornerstone of Mediterranean agriculture, providing substantial economic, cultural and environmental benefits while supporting high levels of biodiversity. However, olive production remains severely constrained by the olive fruit fly, B. oleae (Rossi, 1790) (Diptera: Tephritidae), the most economically damaging pest of olives worldwide. Larval feeding inside the fruit causes premature drop, yield losses frequently exceeding 30–50 %, and significant degradation of olive oil quality through increased acidity and microbial contamination.1,2 For decades, chemical control of B. oleae has relied heavily on synthetic insecticides. This intensive use has promoted the selection of pre-existing resistant alleles in natural populations, resulting in the widespread evolution of insecticide resistance3,4 Moreover, such practices have caused significant negative impacts on non-target organisms, including natural enemies, while raising growing concerns for human health and environmental sustainability. In this context, organically managed and low-input olive groves have emerged as valuable model systems for developing more sustainable integrated pest management (IPM) strategies. A recent systematic map of control methods for the olive fruit fly highlights the urgent need for diversified approaches that go beyond conventional chemical reliance.5 Production systems that rely less on synthetic insecticides and promote habitat heterogeneity and plant diversity generate complex ecological conditions, with diverse alternative host plants, microclimatic variation, and increased biodiversity.6 These factors strongly shape B. oleae behaviour and population dynamics. In such environments, alternative food resources, together with cultural practices, pheromone-based mass trapping, and biological control, can influence adult survival and fecundity under organic olive production.7 In heterogeneous environments, adult flies interact with a variety of landscape elements, and the availability of alternative resources can influence their movement and local abundance.8 Some tephritid species also show that, during host-searching, adults can exploit a wide range of alternative food sources, including crop pollen.9 In agro-diversified agroecological systems, Ceratitis capitata, like other tephritid species, is known to exhibit pronounced phenotypic plasticity.10 Such ecological complexity can shape morphological traits and generate substantial intraspecific variation, highlighting the importance of detailed morphological studies in entomology.11 Previous research has addressed the evolution of morphological traits,12,13,14,15 whereas other studies have concentrated on the development and application of geometric morphometric approaches.16,17 In B. oleae specifically, functional morphology in response to fruit composition has been evidenced through sensory analyses.18 A recent study by Pajač Živković et al.19 demonstrated the utility of geometric morphometrics in capturing cultivar-specific morphological adaptations of B. oleae. The authors showed that olive cultivars differ in their susceptibility to the insect, and may influence population variability. Moreover, as reported by Pajač Živković et al.,19 this phenotypic plasticity of B. oleae such as wing shape and sexual dimorphism may enhance dispersal and oviposition efficiency in olive fruits. Accurate identification and monitoring of locally adapted populations therefore represent a significant challenge for organic olive production.
Although fruit characteristics clearly play a major role in determining olive susceptibility to B. oleae attack, the insect’s own morphological responses remain poorly documented. Only a limited number of studies have described intraspecific morphological variation within olive agroecosystems, and very few have quantified how such variation may influence performance traits in B. oleae. This gap is particularly evident across the Mediterranean basin, where diverse production systems and environmental conditions could promote substantial phenotypic differentiation.
Within defined environments such as organically managed systems, investigating morphological variability in B. oleae is especially relevant. Beyond descriptive accounts, determining whether this variability has a detectable genetic basis remains an open question that has not yet been systematically addressed. Establishing such connections would provide a valuable framework for linking morphological diversity with genomic data and strengthening future comparative studies across cultivars, orchards, and geographic regions.
Population genetic studies have revealed substantial polymorphisms and complex colonization histories of B. oleae across the Mediterranean basin and olive groves areas and.20,21 These patterns have been supported by the early development of polymorphic microsatellite markers.22 More recently, genomic technologies have opened new avenues for pest management by providing insights into population structure, gene flow, and potential adaptive mechanisms.23,24 Complete mitochondrial genomes, in particular, offer higher resolution for detecting fine-scale haplotype diversity compared to partial gene fragments.25 Although conventional markers have revealed relatively high genetic diversity combined with limited geographic structure and high gene flow among Mediterranean populations,26,27 mitogenomic data from organically managed olive groves remain scarce.
In the present study, B. oleae adults were collected from a traditional organic olive orchard in Órgiva (Granada, southern Spain). We documented morphological variability within this local population, focusing on traits associated with fecundity and survival potential on two local olive varieties (Picual and Picholine), and assembled a complete mitochondrial genome using Oxford Nanopore long-read sequencing (GenBank accession PZ179621). This work provides both a high-quality reference mitogenome and a detailed morphological baseline from an organic biotope, offering a valuable foundation for future comparative analyses and the development of region-specific molecular tools to support sustainable integrated pest management strategies against B. oleae.
2. Materials and methods
2.1 Description of the sampling site
The study was conducted in a traditional, organically managed olive orchard located near Órgiva, Granada Province, southern Spain (36°53′47.56″N, 3°24′01.46″W; elevation 401 m a.s.l.) (Figure 1). The orchard is situated on mountain slopes and comprises approximately 450 olive trees of the varieties Picual and Picholine, each around 60 years old. It is embedded within a heterogeneous Mediterranean agroecosystem that includes mixed crops such as citrus, carob, and pomegranate, together with forest trees, hedgerows, and patches of natural vegetation. Management follows low-input organic practices, with minimal use of synthetic pesticides and fertilizers, relying mainly on pheromone-based mass trapping and other ecological methods.
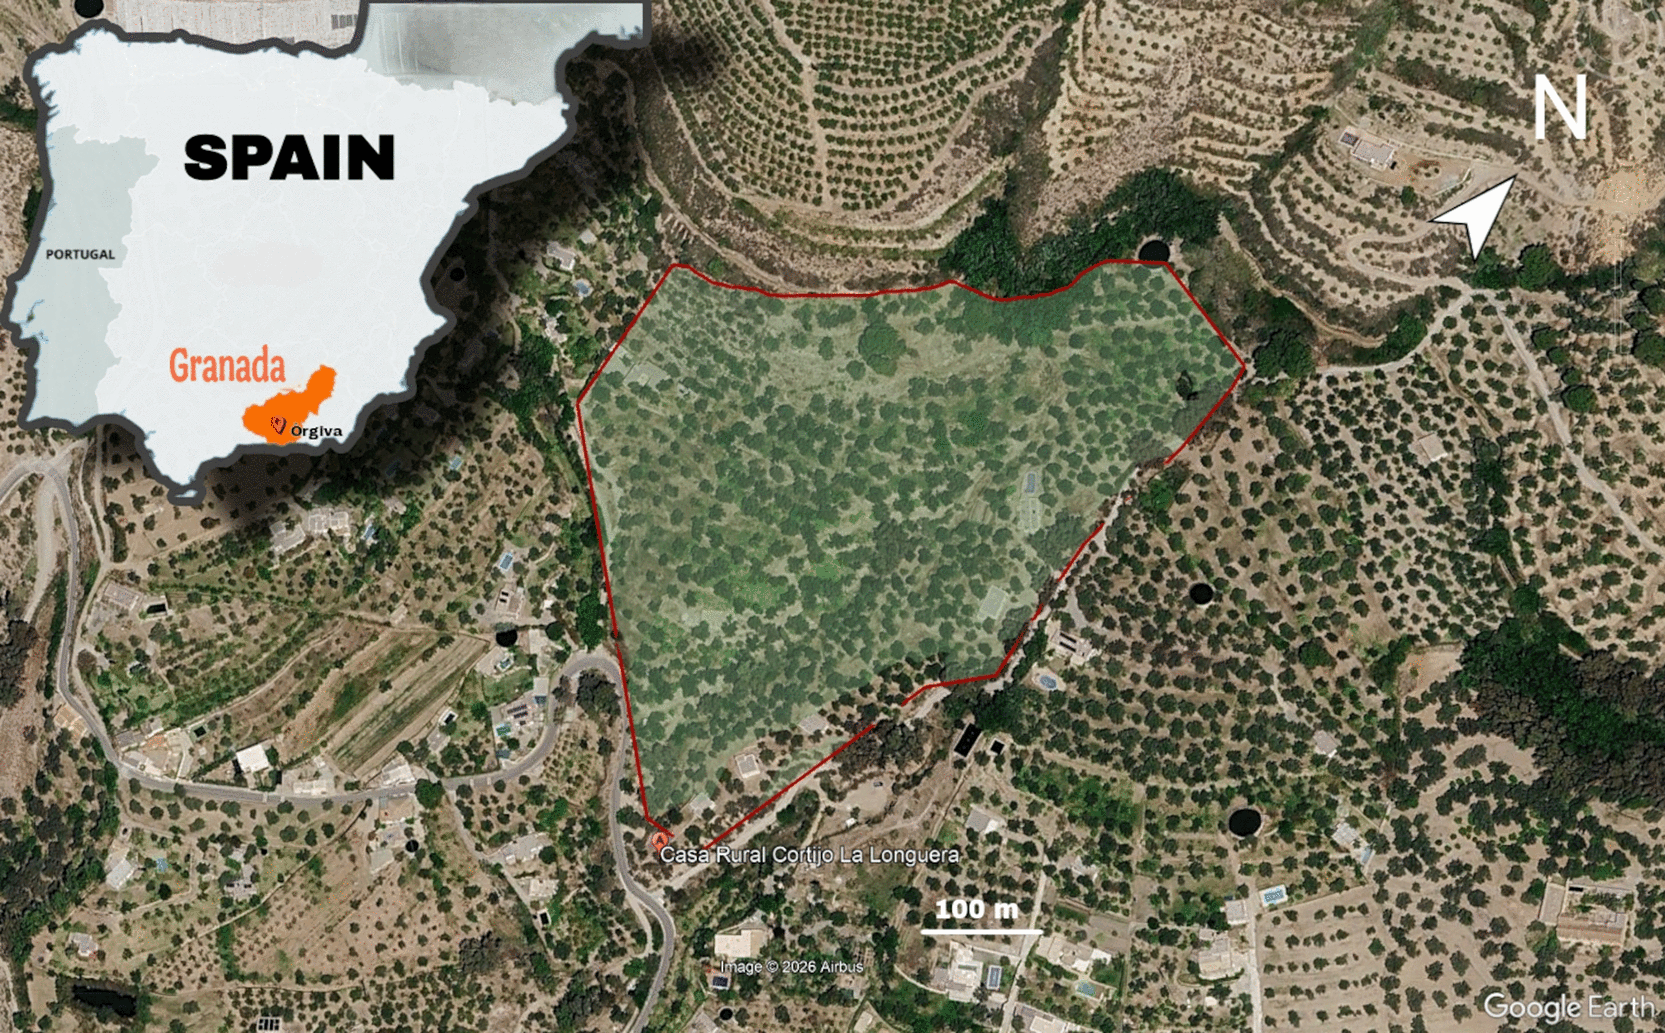
Figure 1. Area of sampling in southern Spain.
The red polygon outlines the olive orchard (~450 olive trees of the varieties Picual and Picholine) in Órgiva (36°53′47.56″N, 3°24′01.46″W, Granada). The inset map (upper left) indicates the position within Spain. Satellite imagery from Google Earth (2026). Mapping and annotations performed with GIMP 3.0.8-2.
2.2 Sample collection and rearing protocol
B. oleae adults were obtained from naturally infested olive fruits collected from about 180 trees of the traditional Lechín and Picual varieties in the study orchard. Sampling was conducted between September and December 2024, a period characterized by moderate infestation levels of approximately 30–40%. Infested fruits were collected and placed in transparent plastic containers covered with aerated fabric to ensure ventilation and prevent mould development. They were then transferred to larger containers fitted with a fine-mesh zippered lid and maintained in controlled-environment chambers at 25 °C and 70 % relative humidity (reduced to ~65 % during pupation) under a 16:8 h (L:D) photoperiod until adult emergence. Emerging adults were examined to document morphological caraterisctics and subsequently preserved at −20 °C in 70% ethanol prior to DNA extraction.
2.3 Imaging procedure and morphological characterization
A total of 140 B. oleae adults were examined using an Olympus SZX61 stereomicroscope at 50× magnification, equipped with an integrated digital camera. All images were captured under standardized lighting conditions and processed with GIMP (v2.10) to standardize background, brightness, and contrast while preserving natural morphological features. A calibrated 2 mm scale bar was included in each photograph to enable accurate morphometric measurements.
The following morphological traits were quantified for each individual: thoracic pigmentation, abdominal banding intensity, abdomen shape (length-to-width ratio), ovipositor morphology (females only), and body length measured from the anterior margin of the head to the tip of the abdomen. Thoracic pigmentation was scored on a scale of 1–5, where 1 represented light yellowish-brown uniform coloration and 5 indicated dark reddish-brown with strongly contrasting pigmented zones. Abdominal banding intensity was scored on a similar 1–5 scale, ranging from absent or very faint (1) to wide, strongly marked black transverse bands (5). Abdomen shape was quantified as the length-to-width ratio. Ovipositor morphology was assessed qualitatively on a scale of 1–4 (1 = slender and straight; 4 = short, robust, curved or pointed). Six morphological groups were initially defined based primarily on thoracic pigmentation and abdominal banding scores. All measurements and scorings were performed by the same observer to ensure consistency. Statistical analyses were subsequently conducted to verify and refine this preliminary classification, assessing whether the observed morphological groupings were supported by quantitative data.
2.4 Statistical and multivariate analyses
Data normality was evaluated using the Shapiro–Wilk test and non-parametric tests were applied. Differences in body length and abdomen L/W ratio among the six morphological groups were analyzed using the Kruskal–Wallis test, followed by Dunn’s post-hoc test for multiple comparisons (p < 0.05). To explore overall morphological variation and validate the group structure, a Principal Component Analysis (PCA) was performed on standardized variables to identify the main axes of variation. Hierarchical clustering using Ward’s method and Euclidean distance was then applied to the PCA scores to classify individuals into clusters. All analyses and visualizations were performed in R v4.5.228 using the packages FactoMineR, factoextra, and ggplot2. Significance was set at p < 0.05.
2.5 Adult longevity and fecundity assays
To assess potential differences in fitness-related traits among the six morphological groups, longevity and oviposition performance were evaluated under controlled laboratory conditions. For each morphological group, three replicates were prepared, each consisting of three females selected from the 140 emerged adults plus two males from the same rearing batch (to ensure mating). Thus, a total of 9 females and 6 males per morphological group were tested. Replicates were maintained in aerated containers constructed from fine muslin fabric, each fitted with an access door and provisioned with 30 healthy, fresh olives (15 Picual and 15 Picholine). Olives were replaced every 5 days. Adults were provided with a continuous source of food consisting of diluted honey on cotton wool and water. The experiment was conducted under under the laboratory’s ambient temperature and humidity conditions.
Longevity was recorded daily until the death of all individuals. Oviposition was evaluated by counting the total number of punctures (stings) on the olives and distinguishing between fertile punctures (those containing an egg) and sterile punctures.
The percentage of fertile punctures was calculated as:
This was calculated separately for Picual and Picholine cultivars. Statistical analyses were performed using one-way ANOVA to test for differences among morphological groups, followed by Tukey’s HSD post-hoc tests to identify pairwise differences in longevity and fecundity.
2.6 DNA extraction, sequencing and basecalling
High-molecular-weight genomic DNA was extracted from a pool of 40 adult B. oleae individuals, selected from the 140 morphologically characterized specimens and preserved in 96% ethanol. This pooling approach ensured sufficient high-quality DNA for Oxford Nanopore long-read sequencing while providing a representative consensus mitogenome of the Órgiva population.
Specimens were first rinsed thoroughly three times with nuclease-free water to remove residual ethanol, gently air-dried on sterile filter paper at room temperature, snap-frozen in liquid nitrogen, and stored at −80°C until extraction. Approximately 25 mg of pooled tissue was mechanically pulverized in a pre-chilled mortar and pestle. DNA extraction was performed using the MagAttract HMW DNA Mini Kit (Qiagen, Hilden, Germany) following the manufacturer’s instructions for insect tissue, with minor modifications only in the initial tissue homogenization step to optimize yield from pooled samples.
DNA quality and quantity were assessed using a NanoDrop 2000 spectrophotometer (Thermo Fisher Scientific) for purity ratios (A260/A280 ≈ 1.8–2.0 and A260/A230 > 1.8) and a Qubit 4.0 fluorometer (Invitrogen) for accurate double-stranded DNA concentration. Only extracts meeting high-quality thresholds were used for library preparation.
Sequencing libraries were prepared using the Native Barcoding Expansion 1–24 (EXP-NBD114) and the Ligation Sequencing Kit (SQK-LSK114) (Oxford Nanopore Technologies). Sequencing was performed on a PromethION P2 Solo instrument equipped with a FLO-PRO114M flow cell. Basecalling was conducted with Guppy v6.5.7 using the “super-accurate” (SUP) model. This generated 3.11 Gb of raw data from 2,391,348 reads (mean read length 1,301 bp). A total of 37,405 reads (53 Mb) mapped to the B. oleae reference mitochondrial genome, providing an average coverage depth of approximately 3,600×. Sequencing and library preparation were carried out by Secugen S.L. (Madrid, Spain).
2.7 Mitochondrial genome mapping, assembly, annotation
Nanopore long reads were mapped to the B. oleae reference mitochondrial genome (GenBank CM090314.1) using minimap2 v2.28 with the “map-ont” preset. Mapped reads were extracted and assembled de novo with Flye v2.9.5 in high-accuracy mode (--nano-hq). The consensus sequence was polished with Medaka using the r1041_e82_400bps_sup model. Functional annotation was performed with MITOS2 v2.1.9 using the NCBI invertebrate mitochondrial genetic code (translation table 5). Nucleotide composition and codon usage were calculated in MEGA v11.29 Statistical analyses were performed in R v4.5.2,28 including a one-way ANOVA to assess variability among genes, with standard deviations computed from raw gene-level values.
2.8 Comparative and phylogenetic analyses
2.8.1 COI Distance analysis
The cytochrome c oxidase subunit I (COI) gene was extracted from the assembled mitogenome and aligned with COI sequences from closely related Bactrocera and Dacus species retrieved from GenBank. Pairwise genetic distances were calculated under the Tamura–Nei 93 (TN93) substitution model30 using MEGA v1129 to evaluate species-level divergence and the diagnostic utility of COI for B. oleae identification. Pairwise mitochondrial genome distances from full alignments were visualized as a heatmap with hierarchical clustering. Distance matrices were generated in R v4.5.228 using the pheatmap package v1.0.1231 with Euclidean distance metrics and complete linkage, and refined with ggplot2 v3.5.32
2.8.2 Phylogenetic reconstruction
To position the Órgiva B. oleae mitogenome within Tephritidae, complete mitochondrial genomes of 19 representative species were used. The dataset included 14 Bactrocera species (B. dorsalis, B. cucurbitae, B. zonata, B. carambolae, B. tryoni, B. correcta, B. scutellata, B. limbifera, B. melastomatos, B. umbrosa, B. tuberculata, B. caudata, B. biguttula, B. ritsemae), three Dacus species (D. bivittatus, D. longicornis, D. trimacula), Ceratitis capitata as a related outgroup, and Drosophila melanogaster as a distant outgroup. All accessions and references are listed in Table S1. Sequences were aligned using MAFFT v7 with the L-INS-i algorithm. The best-fit nucleotide substitution model was identified using ModelTest in MEGA X. A Maximum Likelihood phylogenetic tree was reconstructed in MEGA X with 1,000 bootstrap replicates and rooted with D. melanogaster. Tree visualization was performed using MEGA X. Finally, the newly assembled B. oleae mitogenome was aligned with the Italian reference sequence (NC_005333.1) using MAFFT v7. Pairwise nucleotide differences were identified and classified as synonymous or non-synonymous using MEGA v11 under the invertebrate mitochondrial genetic code.
3. Results and analyses
3.1 Morphological analyses and adult performances
3.1.1 Definition of morphological groups
From the rearing protocol, 140 adult B. oleae successfully emerged from naturally infested olives collected from the organic orchard in Órgiva. All specimens exhibited the diagnostic traits of the species, with body length ranging from 4.2 to 5.1 mm (mean ± SD: 4.68 ± 0.23 mm). Compared to the typical Spanish phenotype described by Ruiz Castro (1948)33 (Figure 2), characterized by a yellowish-brown thorax, pale scutellum, and elongated abdomen with subtle lateral markings, the emerged adults displayed notable intraspecific variation in thoracic pigmentation, abdominal banding, abdomen shape, and ovipositor morphology. Quantitative assessment allowed the classification of all 140 individuals into six distinct morphological groups based primarily on thoracic pigmentation and abdominal banding intensity (
Table 1). Representative specimens of each morphological group were photographed to illustrate this variation (Figure 3A–L). Group 1 (Typical light form) was the most abundant (27.9%), whereas Group 3 (Compact orange form) was the rarest (6.4%). Thoracic pigmentation scores ranged from 1 (light yellowish-brown, uniform) to 5 (dark reddish-brown with strongly contrasting zones; overall mean 3.1 ± 1.3). Abdominal banding intensity ranged from 1 (faint or absent) to 5 (pronounced transverse black bands; overall mean 2.9 ± 1.4). Abdomen length-to-width ratios varied between 1.50 (compact) and 2.00 (elongated). Among females, ovipositor morphology ranged from slender and straight to short and blunt. Body length differed significantly among groups (Kruskal–Wallis test, H = 28.4, p < 0.001), with individuals in Groups 3 and 6 being significantly smaller than those in Groups 1, 4, and 5 (Dunn’s post-hoc test, p < 0.05). The abdomen L/W ratio also varied significantly among groups (H = 45.7, p < 0.001), with Group 6 showing the most compact shape.
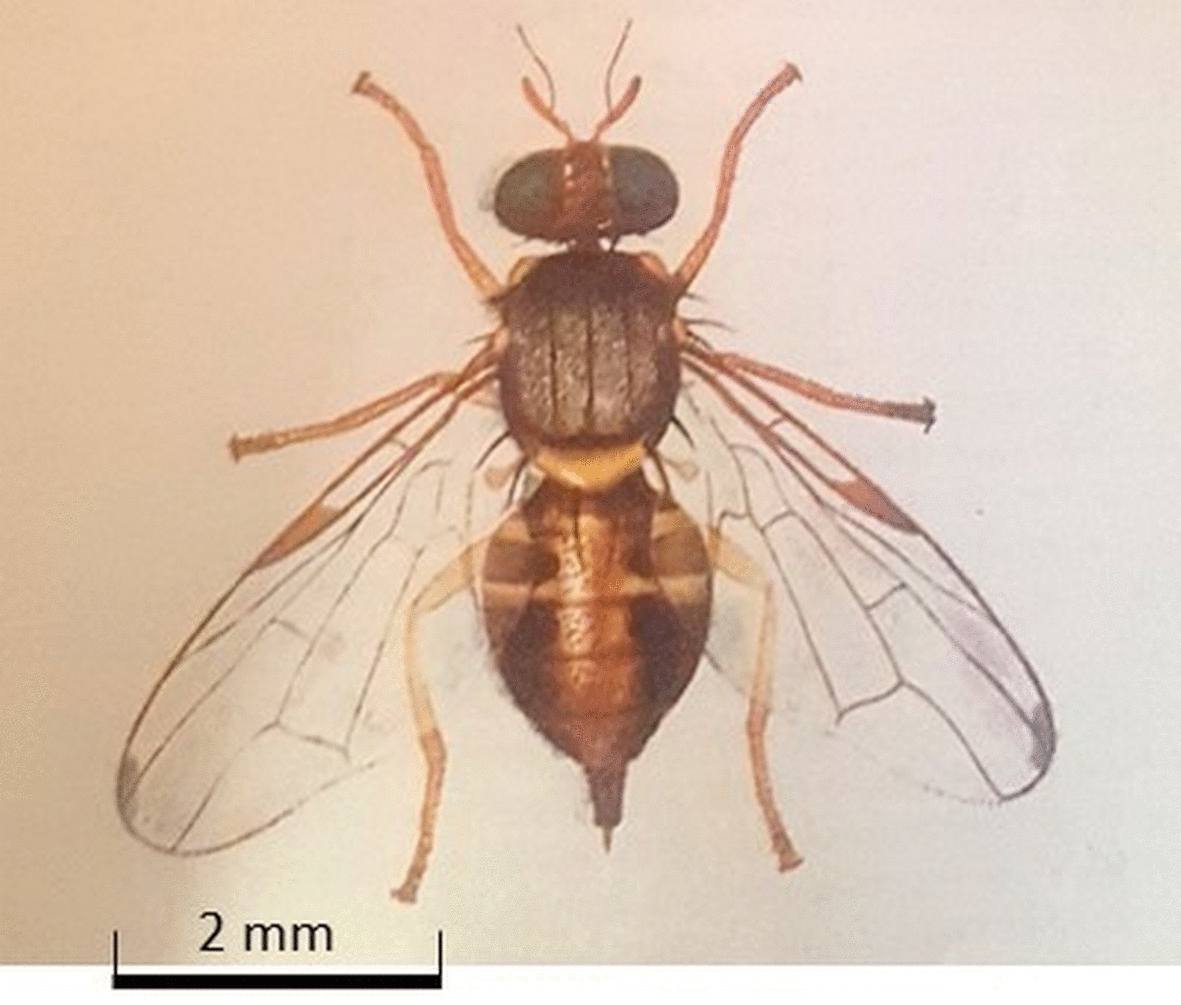
Figure 2. Reference specimen of the olive fruit fly Dacus oleae, as described by Ruiz Castro (1948) in Fauna entomológica del olivo en España.
Table 1. Morphological variation among 140 B. oleae adults collected from the organic olive orchard at Orgiva, southern Spain.
Values are presented as mean ± SD or range. Groups were defined primarily by thoracic pigmentation and abdominal banding intensity scores.
| Morphological Group* |
Description | Thoracic pigmentation (1–5) | Abdominal banding (1–5) | Abdomen L/W ratio | Ovipositor morphology (♀) | Body length (mm)** | n (%) | Representative specimens (Figure 3) |
|---|
| 1) Typical light form
| Brown thorax with faint markings, slender body and pale abdomen | 4–5 | 3–5 | 1.80–1.95 | Slender, straight | 4.75 ± 0.22a | 39 (27,9) | B, I |
| 2) Dark thoracic form
| Dark reddish-brown thorax, contrasting pigmentation | 4–5 | 2–3 | 1.65–1.80 | Robust, slightly short | 4.65 ± 0.18ab | 23 (16.4) | E, K |
| 3) Compact orange form
| nearly square thorax, compact and rounded abdomen, characteristic bright orange | 1–2 | 1–2 | 1.50–1.65 | Short and blunt | 4.50 ± 0.25b | 9 (6.4) | G |
| 4) Brown elongated thorax
| Elongated brown thorax, dark transverse bands on the abdomen | 2–4 | 2–4 | 1.70–1.85 | characteristically long | 4.80 ± 0.20a | 26 (18.5) | H |
| 5) Pronounced
abdominal banding
| Brown thorax, strong transverse black bands, compact abdomen | 3–4 | 4–5 | 1.85–2.00 | Long, straight | 4.85 ± 0.15a | 24 (17.1) | F, L |
| 6) Dark compact form
| Blackish robust thorax, white scutellum, rounded compact abdomen | 1–3 | 1–2 | 1.55–1.70 | Short to medium,
robust | 4.59 ± 0.27b | 19 (13.6) | C, J |
| Overall
| - | 3.1 ± 1.3
| 2.9 ± 1.4
| 1.74 ± 0.16
| - | 4.68 ± 0.23
| 140 (100)
| A–L |
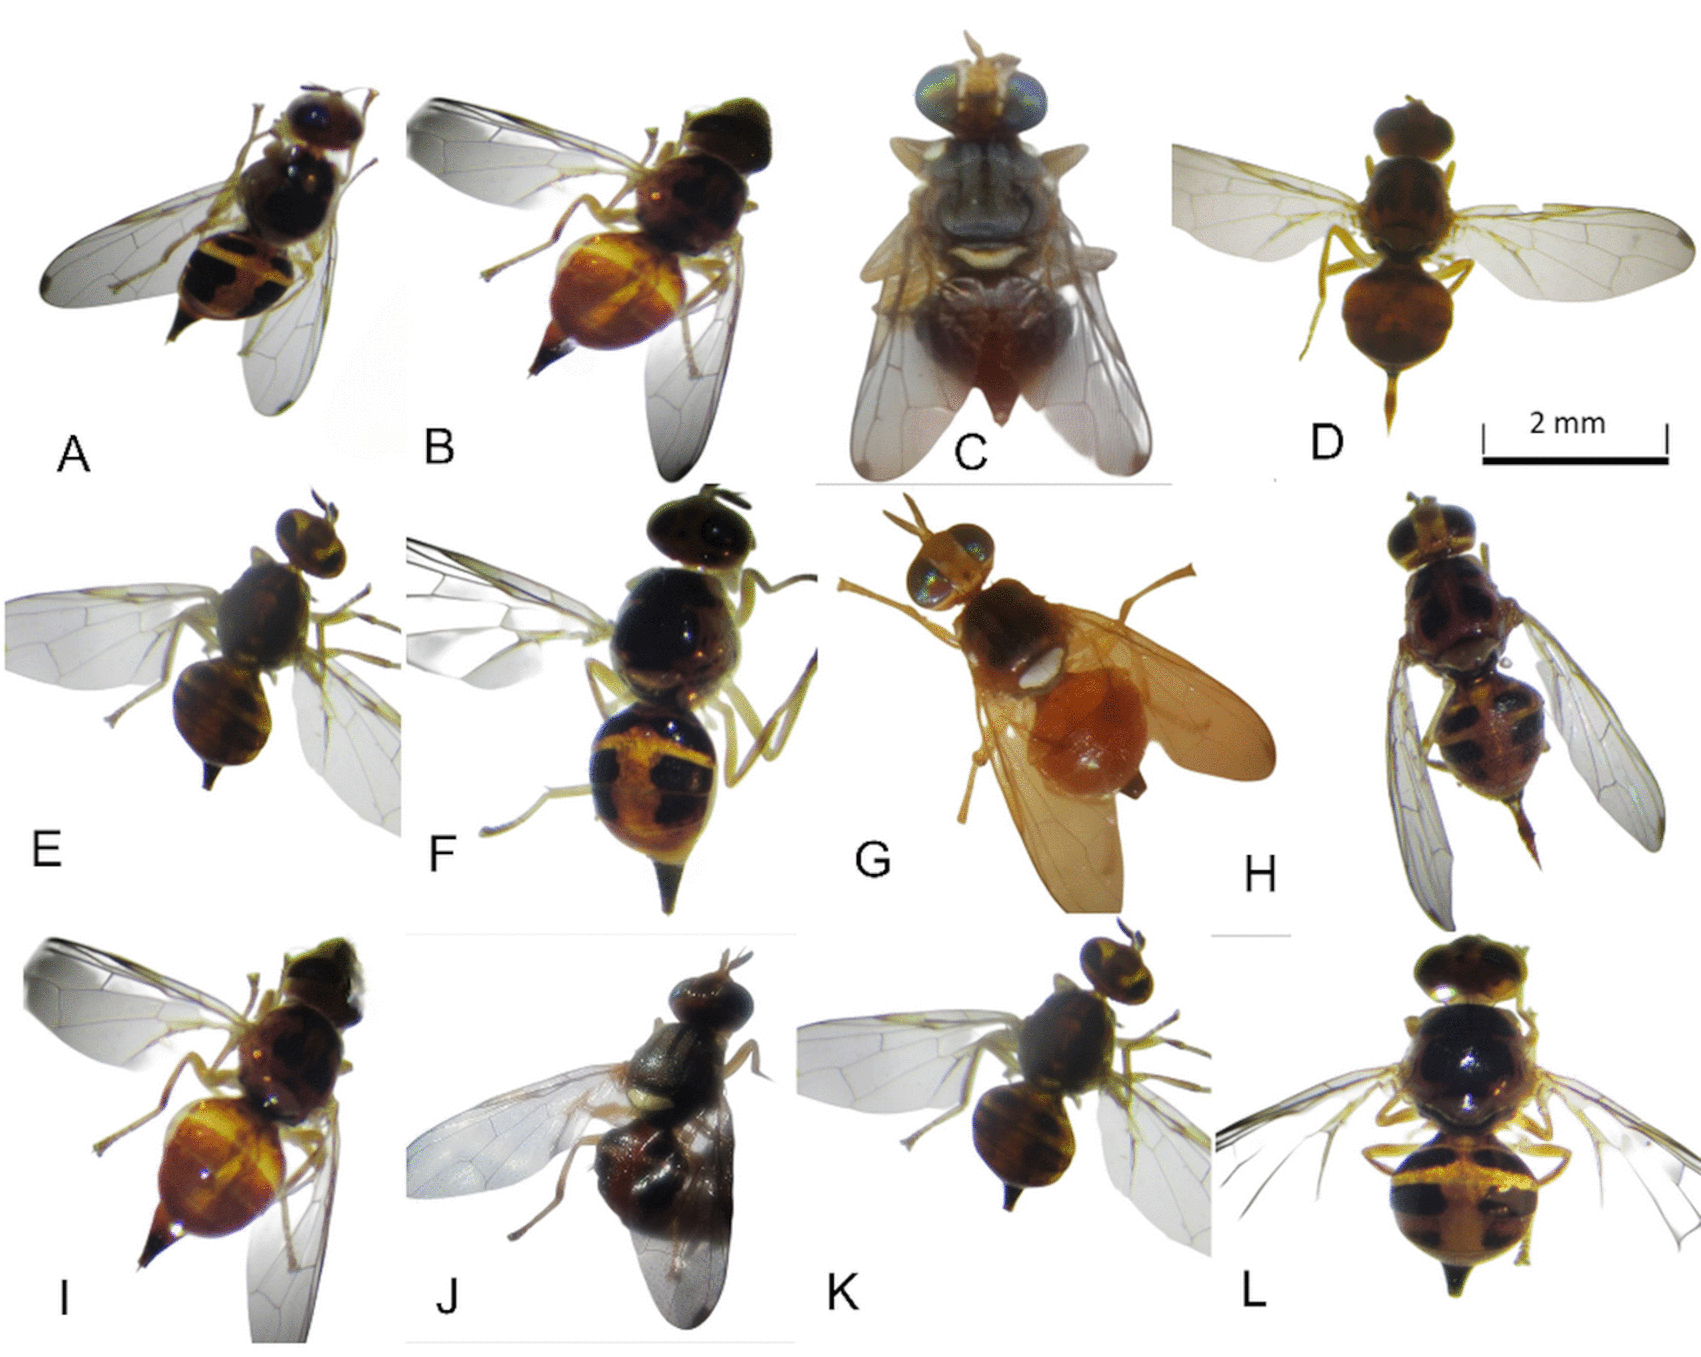
Figure 3. Representative specimens of the six morphological groups of B. oleae adults emerged from the organic olive orchard in Órgiva, southern Spain.
Panels A–L show representative specimens of the six morphological groups defined in
Table 1. Scale bar = 2 mm. Olympus SZX61 stereomicroscope and processed with GIMP (v2.10).
Principal Component Analysis (PCA) revealed that the first two dimensions accounted for 95.4% of the total variance (Dim1 = 87.5%, Dim2 = 7.9%), with Dim1 driven by thorax length, thorax width, and ovipositor length, reflecting overall body size, while Dim2 was associated with abdomen proportions (Figure 4). Building on these results, hierarchical clustering using Ward’s method identified six well-defined clusters (Figure 5), which corresponded closely to the morphological groups defined by pigmentation and banding scores. The clusters were primarily separated along Dim1, confirming body size as the dominant axis of differentiation. The different analyses reveal that Groups 3 and 6 were characterized by smaller body size and compact abdominal morphology, whereas Groups 1, 4, and 5 were distinguished by larger thoracic dimensions and elongated ovipositors.”
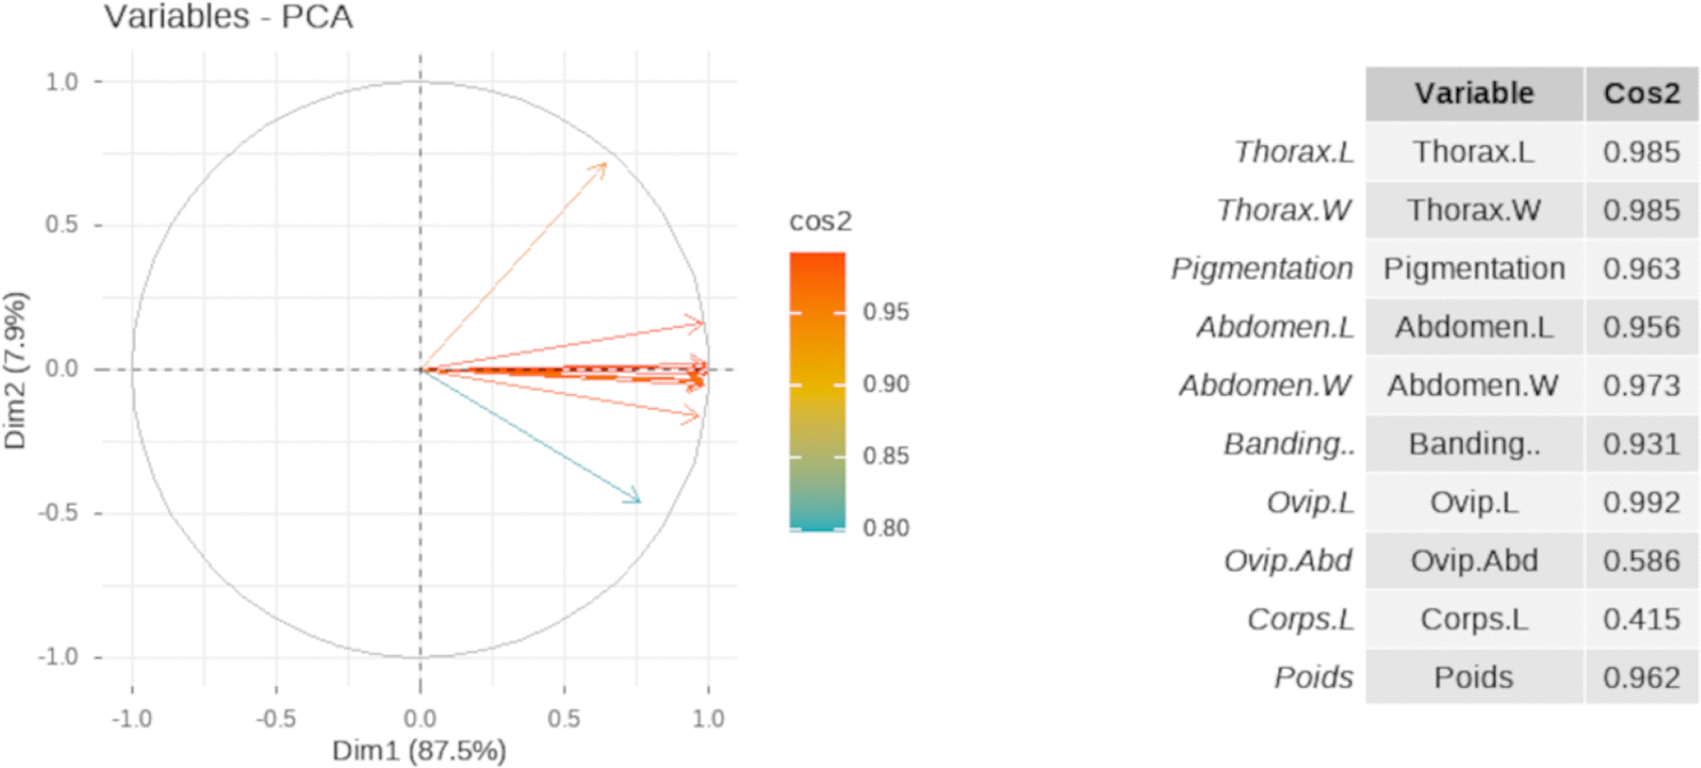
Figure 4. Principal Component Analysis (PCA) of morphological traits in B. oleae performed on 140 adults collected from the organic olive orchard at Orgiva.
Generated in R v4.5.2 using ggplot2.
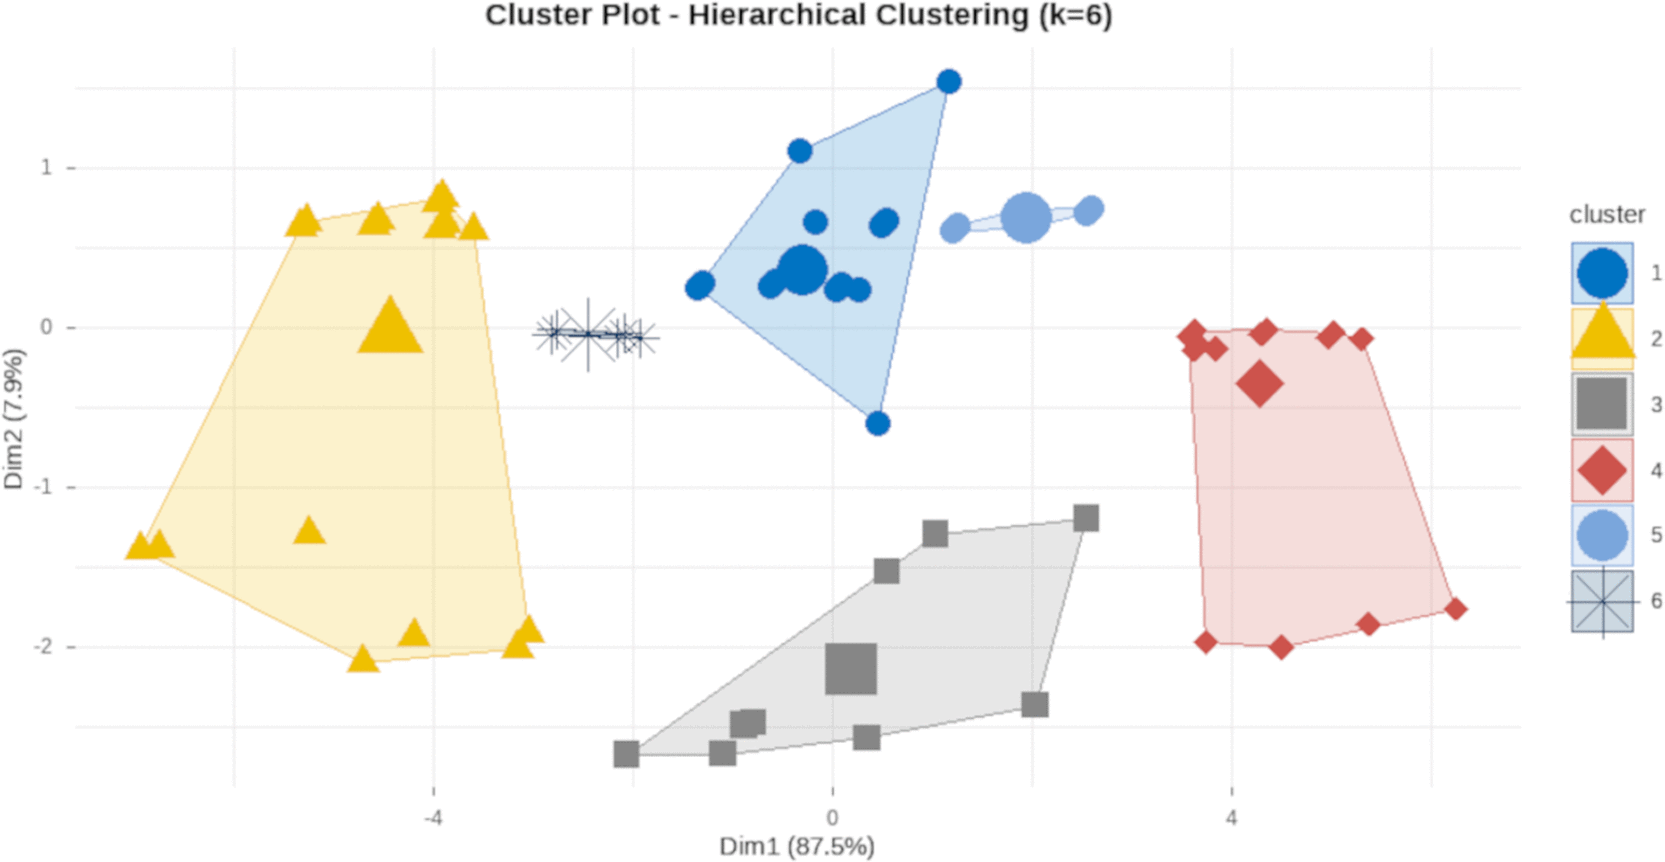
Figure 5. Hierarchical clustering of morphological traits in B. oleae performed on 140 adults collected from the organic olive orchard at Orgiva using Ward’s method, generated in R v4.5.2 with ggplot2.
3.1.2 Longevity and fecundity performance
Significant morphological variation was observed among the 140 emerged B. oleae adults, which were clustered into six distinct groups based on thoracic pigmentation, abdominal banding, body shape, and ovipositor morphology (see
Table 1 and
Figure 3 for representative specimens). Adult longevity and fecundity potential differed significantly among the six morphological groups (
Table 2). Mean longevity ranged from 24.9 ± 2.1 days (Compact orange form) to 31.7 ± 1.8 days (Dark thoracic form). One-way ANOVA revealed significant differences in longevity among groups (F = 4.87, df = 5, p = 0.003).
Table 2. Longevity and fecundity performance of six morphological groups of B, oleae females under laboratory conditions.
| % Fertile punctures on Picholine Mean ± SE | % Fertile punctures on Picual Mean ± SE | Longevity (days) Mean ± SE | Morphological Group |
|---|
| 38.7 ± 2.9b | 42.1 ± 3.2b | 28.3 ± 1.4ab | 1) Typical light form |
| 41.2 ± 3.1ab | 45.3 ± 2.8ab | 31.7 ± 1.8a | 2) Dark thoracic form |
| 32.4 ± 3.7c | 35.6 ± 4.1c | 24.9 ± 2.1b | 3) Compact orange form |
| 48.5 ± 3.4a | 51.7 ± 2.9a | 29.8 ± 1.5ab | 4) Brown elongated thorax |
| 46.9 ± 2.8a | 49.8 ± 3.0a | 30.4 ± 1.6a | 5) Pronounced abdominal banding |
| 36.8 ± 3.3bc | 39.4 ± 3.5bc | 27.1 ± 1.9ab | 6) Dark compact form |
| 40.8 ± 1.7 | 44.0 ± 1.8 | 28.7 ± 0.8 | Overall
|
Fecundity, expressed as the percentage of fertile punctures, also varied significantly among morphological groups on both olive cultivars. On cv. Picual, the percentage of fertile punctures ranged from 35.6 ± 4.1% (Compact orange form) to 51.7 ± 2.9% (Brown elongated thorax) (F = 8.24, df = 5, p < 0.001). A similar pattern was observed on cv. Picholine, with fertile puncture rates ranging from 32.4 ± 3.7% to 48.5 ± 3.4% (F = 7.65, df = 5, p < 0.001). Post-hoc Tukey’s HSD tests showed that groups 4 (Brown elongated thorax) and 5 (Pronounced abdominal banding), which possessed characteristically long ovipositors, exhibited significantly higher percentages of fertile punctures compared to groups with shorter or blunter ovipositors (groups 3 and 6).
3.2 Mitochondrial genome assembly and gene length variation across tephritidae
Oxford Nanopore sequencing of the pooled sample of 40 adults generated 3.11 Gb of long-read data, yielding a high-quality circular mitochondrial genome of 15,810 bp with an average coverage depth of ~3,600×. (GenBank accession PZ179621) (Figure 6). The assembly contained the complete set of 37 mitochondrial genes (13 protein-coding genes, 22 tRNAs, 2 rRNAs, and one A+T-rich control region) in the typical Tephritidae gene order. Nucleotide composition was strongly AT-biased (72.6%), consistent with other Bactrocera species.
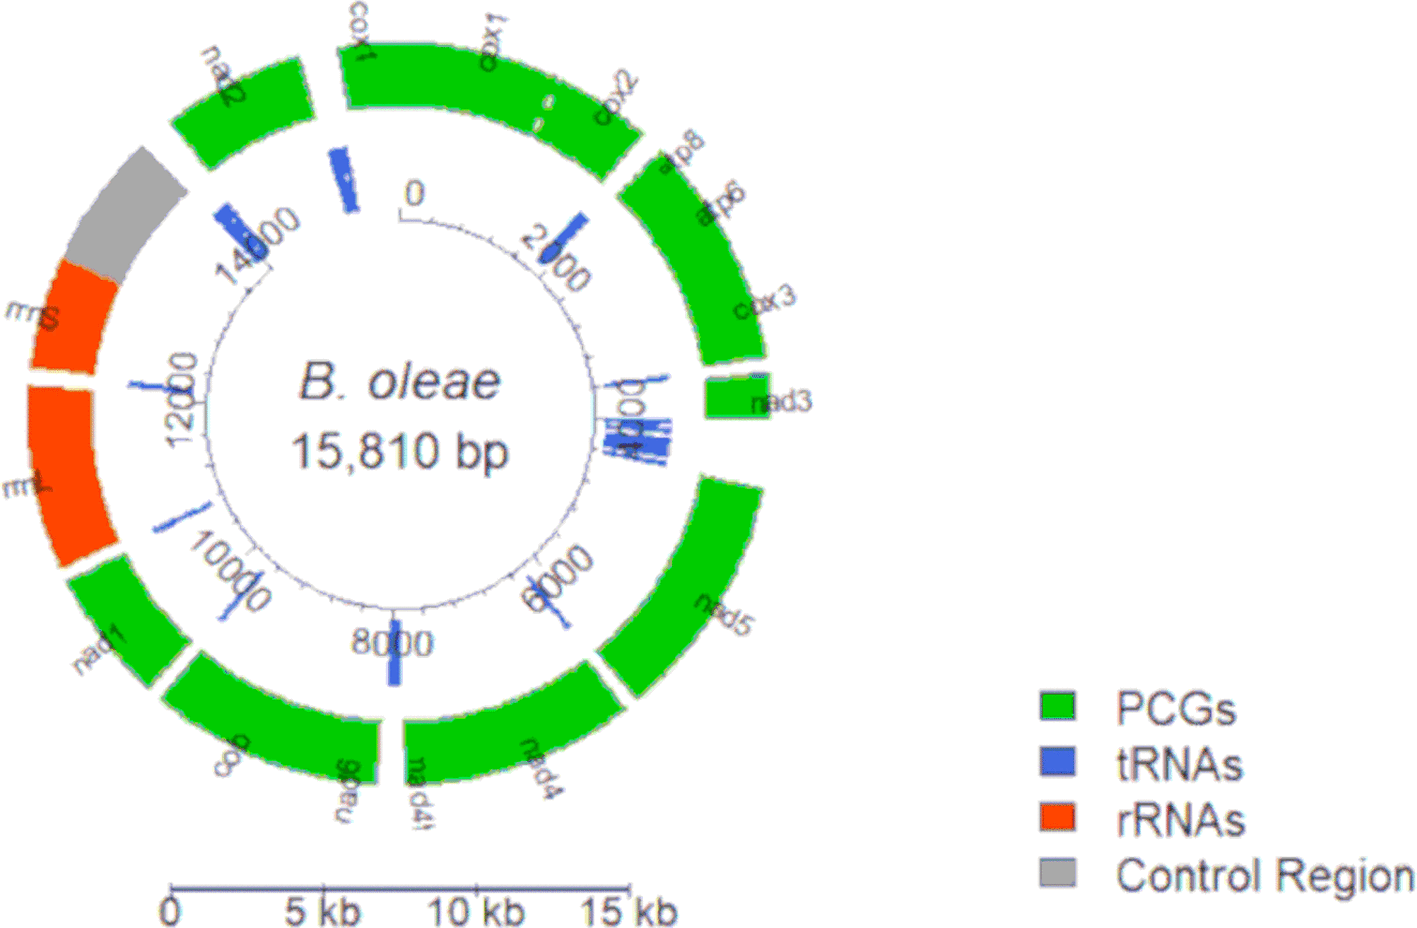
Figure 6. Circular map of the complete mitochondrial genome of Bactrocera oleae (isolate 25OT00063; 15,810 bp).
Protein-coding genes (green), tRNAs (blue), rRNAs (orange), and the A+T-rich control region (grey) are shown. Genes on the majority (J) strand are transcribed clockwise, while those on the minority (N) strand are transcribed counterclockwise. Map generated in R v4.5.2 using the circlize package.
Comparison of the 13 protein-coding genes (PCGs) across Tephritidae mitogenomes revealed strong structural conservation. Most genes showed identical or nearly identical lengths, with modest variation mainly restricted to ND1, ND3, ND5, COX1, and ND6. The Órgiva mitogenome (PZ179621) matched the length patterns of previously published B. oleae sequences. ND3, ND4L, and ND6 were the most conserved (median lengths ≈350 bp, ≈290 bp, and ≈520 bp), whereas ND1 and ND5 showed broader interspecific variation (≈940 bp and ≈1720 bp, with deviations up to ~100 bp). Mean values closely matched medians, indicating minimal skew in the distributions (Figure 7).
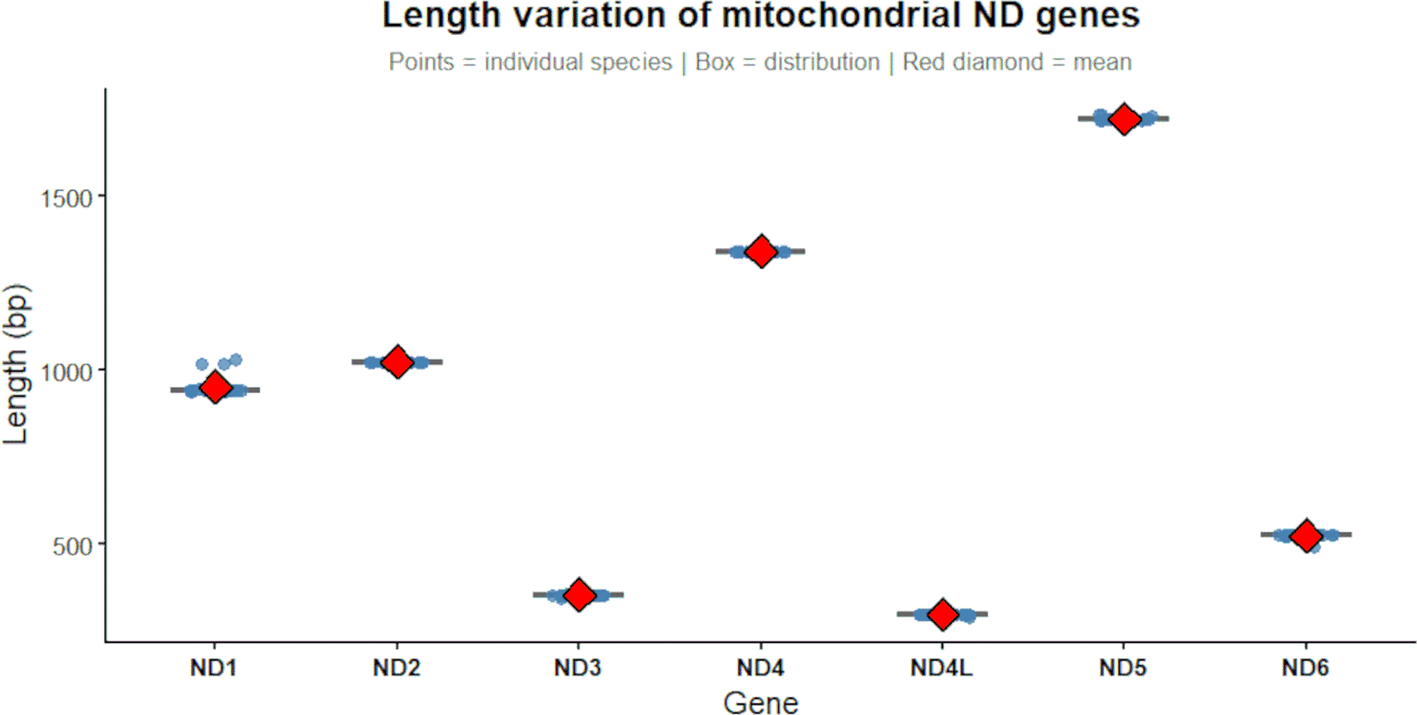
Figure 7. Length variation of mitochondrial NADH dehydrogenase (ND) genes across the Tephritidae species.
Red diamonds indicate mean lengths. Generated in R v4.5.2 using ggplot2.
The Órgiva consensus mitogenome was aligned with three publicly available B. oleae mitogenomes (NC_005333.1, AY210702, AY210703). Pairwise nucleotide divergence ranged from 0.000% to 0.202% (Figure 8). Compared to the Italian reference NC_005333.1, the Órgiva haplotype differed by 21 nucleotide substitutions (0.133% divergence), including 11 non-synonymous changes located mainly in ND (ND1, ND5, ND6) and COX (COX1, COX2) genes. Comparative analysis with the additional mitogenomes confirmed low but detectable intraspecific variation, with no insertions, deletions, or genomic rearrangements observed.
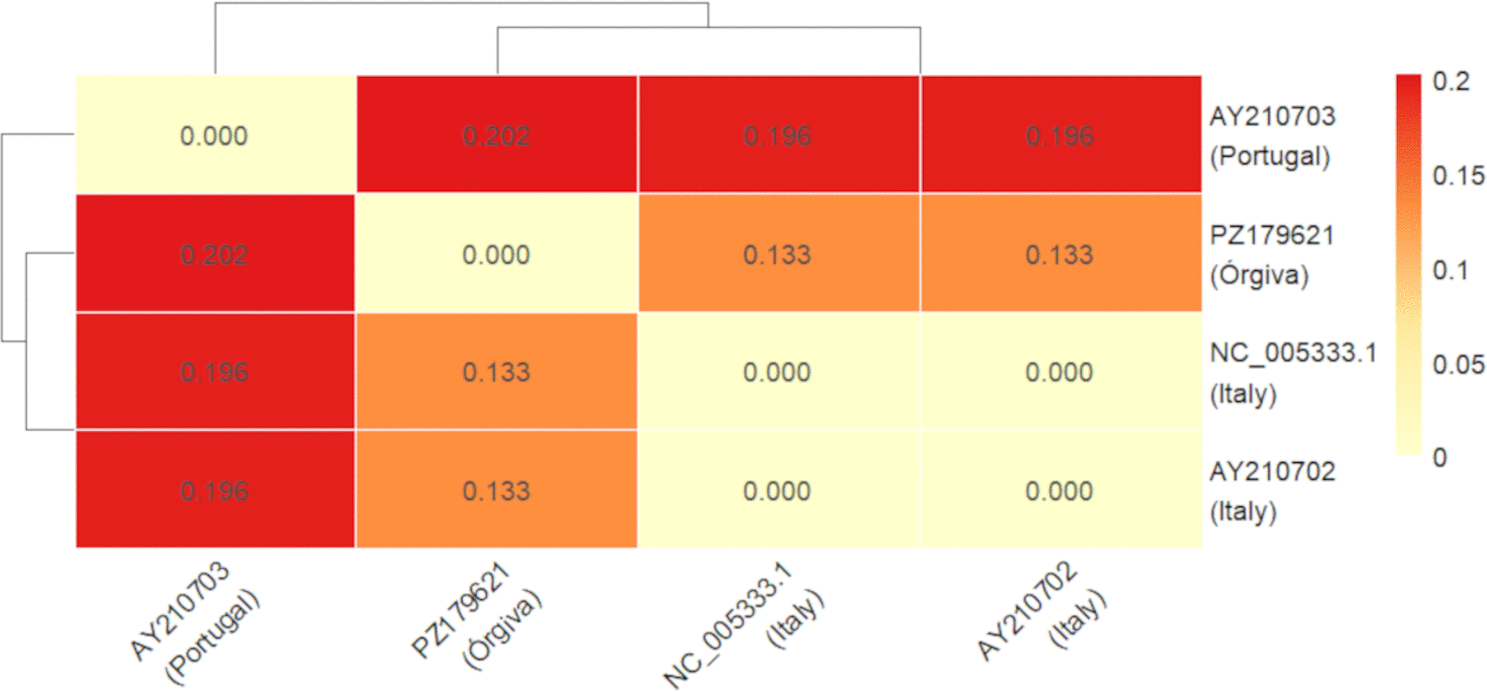
Figure 8. Pairwise nucleotide divergence heatmap of the Órgiva consensus mitogenome of B. oleae (PZ179621) compared with three reference mitogenomes (NC_005333.1, AY210702 and AY210703).
Generated in R v4.5.2 using the ggplot2 package
3.3 Phylogenetic placement and comparative analysis
The multiple sequence alignment of 21 Tephritidae mitogenomes, with Drosophila melanogaster as outgroup, revealed the expected combination of conserved and variable regions typical of insect mitochondrial DNA. The ~15.8 kb alignment contained ~65% conserved sites and ~20% parsimony-informative positions, providing strong phylogenetic signal. Clear genus-level patterns were detected: Bactrocera sequences were highly homogeneous across PCGs, Dacus showed lineage-specific motifs, and Ceratitis displayed distinct substitutions toward the 3′ ends of several genes. As expected, Drosophila was strongly divergent, confirming its suitability as an outgroup.
Maximum Likelihood analyses based on the complete mitogenome alignment produced a well-resolved topology (Figure 9). Bactrocera formed a strongly supported monophyletic clade, clearly separated from Dacus and from the outgroup taxa Ceratitis capitata and Drosophila melanogaster. The Órgiva mitogenome (PZ179621) clustered with full support (bootstrap = 100%) within the Mediterranean B. oleae lineage, showing closest affinity to the reference sequence NC_005333.1. This Mediterranean subclade was clearly distinct from the Asian/African Bactrocera group. Bootstrap values (1,000 replicates) confirmed the robustness of the topology, with ≥98–100% support for most major nodes. Lower support at a few deep nodes did not affect the placement of the Órgiva sequence or the separation between Bactrocera and Dacus.
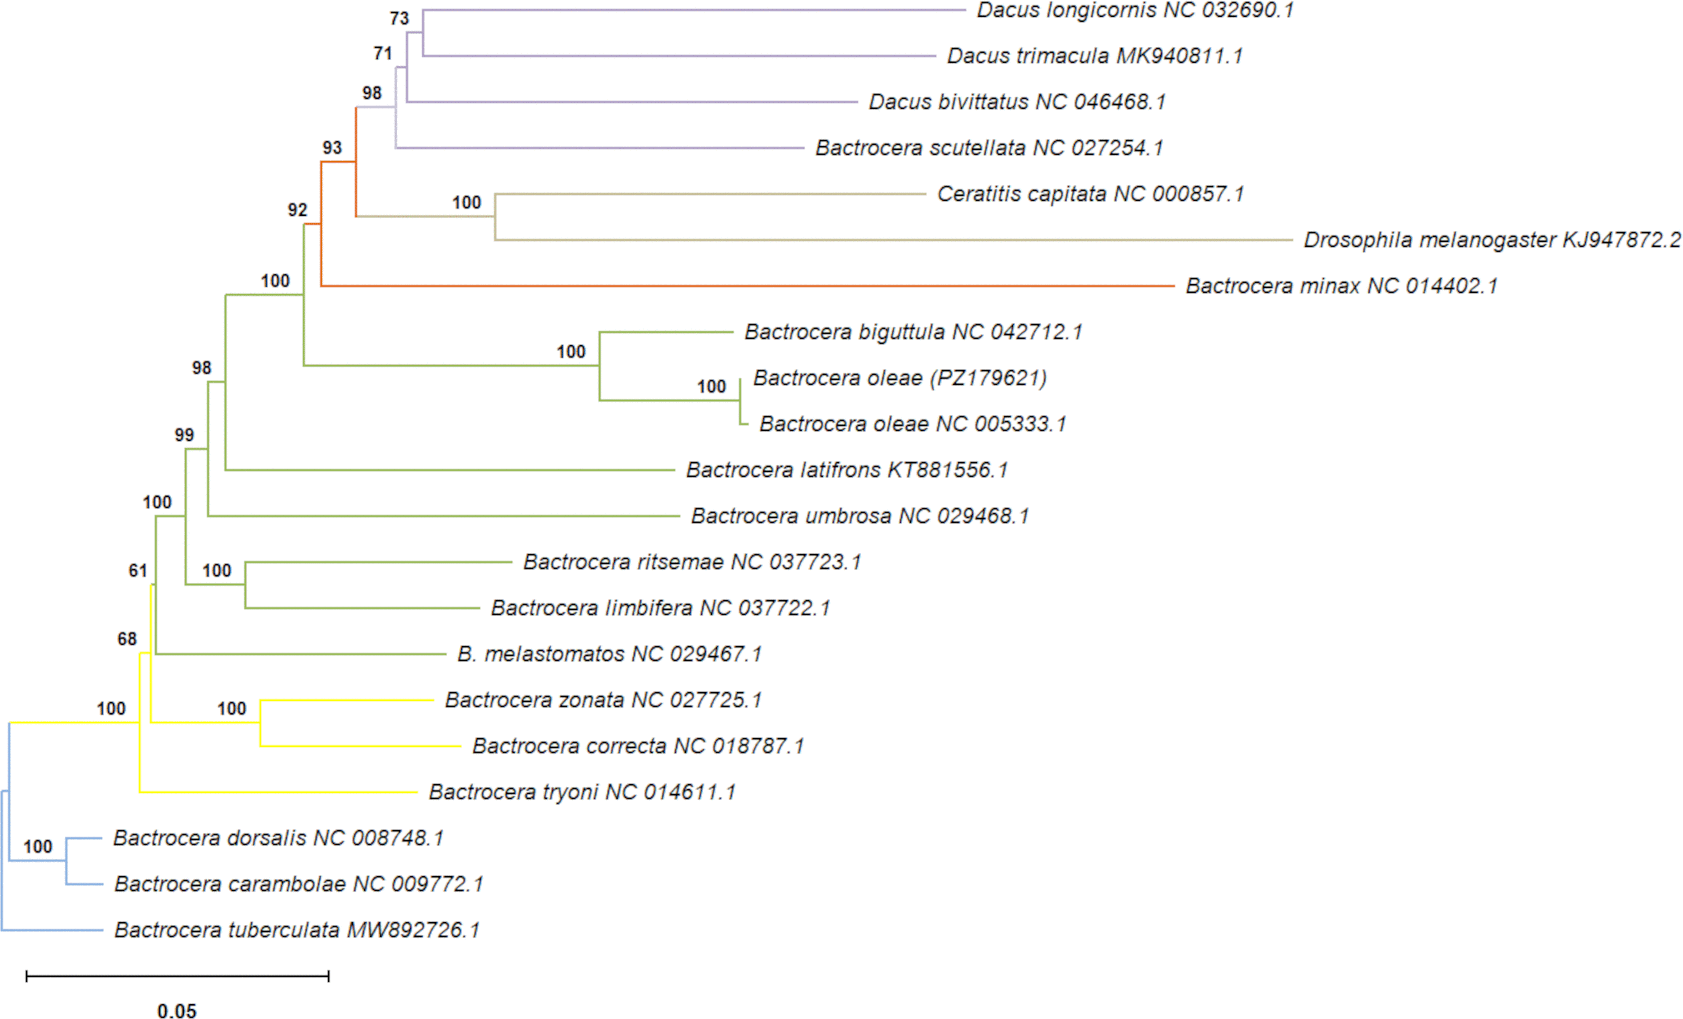
Figure 9. Maximum Likelihood phylogenetic tree of Tephritidae based on complete mitogenomes (21 taxa), with Drosophila melanogaster as outgroup.
The Órgiva haplotype (PZ179621) is highlighted in green. Bootstrap values (≥ 70 %) are shown at nodes. The scale bar indicates substitutions per site.
4. Discussion
This study was carried out in a structurally complex, organically managed olive orchard in southern Spain, characterized by mixed crops, forest patches, and low chemical inputs, representing a typical Mediterranean agroecosystem. This traditional landscape supports high local biodiversity and provides an excellent setting for documenting morphological variation and generating genomic ressources, including the reference mitogenome. These datasets provide a valuable baseline for future comparative research on B. oleae species in Mediterranean olive systems. Field sampling of the autumnal generation, conducted from September to December 2024, revealed moderate to high infestation levels (30–40% of fruits affected) in the Lechín and Picual cultivars. Such infestation rates are typical of organically managed olive orchards with limited pesticide inputs. The observed differences in cultivar susceptibility to B. oleae infestation are consistent with fruit traits such as morphology, maturation timing, and pericarp hardness, which are known to influence oviposition preference and larval performance.34,35,36 This influence may also be combined with factors such as cuticle size and volatile compounds in the fruits.37
In this study, adults of B. oleae reared from naturally infested olives collected in a traditional organic orchard provided a representative sample for documenting intra-specific morphological diversity. All individuals exhibited the diagnostic traits of the species; however, clear intraspecific variation was observed in thoracic pigmentation, abdominal banding, abdomen proportions, and especially ovipositor morphology. The integration of qualitative and quantitative descriptors allowed the classification of adults into distinct morphological groups. Multivariate analyses strongly supported this structure: Principal Component Analysis (PCA) identified body size and ovipositor traits as the primary axes of variation and hierarchical clustering revealed six well-defined morphological groups confirmed the robustness of the classification, with thorax and ovipositor characters emerging as the strongest discriminating variables.
This descriptive framework is consistent with the broader use of morphometric methods in entomology. Multivariate approaches, particularly geometric morphometrics, have proven effective in characterizing functional morphology, sexual dimorphism, and host-associated phenotypic plasticity in various insect groups. In Tephritidae, such techniques have been successfully applied to reveal phenotypic variation and host-induced morphological changes in species such as B. dorsalis and C. capitata.10,38,39
The marked phenotypic diversity, observed among flies emerging from olive cultivars (primarily Lechín and Picual) during the same sampling period and within the same biotope, appears to reflect a certain degree of phenotypic plasticity in response to heterogeneous microhabitats and reduced chemical pressure—conditions typically associated with organic farming. Such variation contrasts with the more uniform morphology historically reported for Spanish populations,33 who described a typical light form (yellowish-brown thorax and pale abdomen) that remains the most frequent phenotype in vast monoculture olive plains and conventional production systems. More recently, studies have demonstrated cultivar-specific morphological adaptations in B. oleae in olive orchards, with cultivar-specific susceptibility.19 Importantly, the occurrence of morphological diversity within the same microhabitat may be attributed to additional factors, including the organic system and habitat heterogeneity. Organic compounds and environmental conditions have been shown to strongly influence oviposition preference and offspring performance in container-breeding insects, providing insights into host selection mechanisms that may also apply to B. oleae.40
The six morphological groups identified showed differences in body size and ovipositor traits, which were associated with variations in longevity and reproductive potential. Adults belonging to groups with elongated ovipositors exhibited both higher longevity and greater reproductive success across Picual and Picholine cultivars, whereas compact forms tended to live shorter and produced fewer fertile punctures. These results suggest a functional link between morphological variation and fitness-related traits, highlighting the adaptive significance of phenotypic plasticity in this organic biotope. Similar associations between ovipositor morphology and reproductive success have been reported in B. oleae populations under controlled laboratory conditions41 and more broadly in tephritid flies where oviposition depth influences host exploitation and fecundity.42
Taken together, these findings emphasize that morphological diversity in B. oleae is not merely a descriptive trait but carries direct implications for fitness and population dynamics. By linking ovipositor morphology to reproductive success, this study highlights how phenotypic plasticity may enhance adaptability in heterogeneous organic olive systems, thereby shaping both pest pressure and management strategies.
The observed variability in thoracic pigmentation, abdominal banding, and ovipositor morphology, combined with the high-quality mitogenome assembly, underscores the potential of integrating morphological and genomic datasets. Such integration provides a basis for developing molecular markers and comparative tools, but this remains a hypothesis that requires verification through longer-term sampling and cultivar-specific analyses. Fruit traits such as cuticle thickness and volatile composition are known to influence olive fly tolerance37 and documenting these factors alongside morphological descriptors will be essential for future work. Establishing robust baselines of morphological diversity and genomic data will ultimately facilitate monitoring of population structure, haplotype distribution, and gene flow between orchards managed under different production systems.
Oxford Nanopore long-read sequencing of a pooled sample of 40 adults, selected to represent the observed morphological diversity, yielded a high-quality circular mitochondrial genome of 15,810 bp (PZ179621), assembled de novo with an average coverage of ~3,600×. This consensus haplotype represents the predominant mitochondrial lineage present in the Órgiva organic population. The mitogenome displays the typical insect quadripartite architecture, including the full complement of 37 genes (13 protein-coding genes, 22 tRNAs, 2 rRNAs, and one A+T-rich control region) and a strongly AT-biased nucleotide composition (72.6 %), consistent with other Bactrocera species.
Comparative analysis with publicly available B. oleae mitogenomes indicates that the Órgiva haplotype exhibits only modest intraspecific variation. The Órgiva haplotype differs from the Italian reference (NC_005333.1) by only 21 nucleotide substitutions including 11 non-synonymous changes, mainly in ND and COX genes. This limited divergence is consistent with the generally low mitochondrial variability reported across Mediterranean populations. Similar patterns of high sequence similarity with other regional haplotypes further support the genetic homogeneity of B. oleae in this area. Phylogenetic reconstruction based on complete mitogenomes placed the Órgiva haplotype with maximum bootstrap support (100 %) within the Mediterranean clade of B. oleae, confirming its genetic coherence with the broader Mediterranean group.25,26 Genomic studies of this pest can further strengthen this approach; for instance, physical mapping of the B. oleae genome has enabled the localization of key genes on polytene chromosomes, offering a valuable foundation for genomic and cytogenetic investigations.43
Based on the proposed grouping classification, the combination of morphological polymorphism (six groups among 140 individuals) with low mitochondrial genetic divergence strongly suggests that the observed variation is primarily driven by phenotypic plasticity rather than deep genetic differentiation. Although 11 non-synonymous substitutions were identified in ND and COX genes, these may hint at local adaptation to organic conditions—characterized by minimal use of pesticides—and microhabitat heterogeneity. Notably, B. oleae shows possible susceptibility to cultivar diversity,19 is influenced by microclimatic and soil heterogeneity44 and may interact with the endosymbiont Candidatus Erwinia dacicola.45,46 However, the present dataset does not allow firm conclusions regarding the functional or adaptive significance of these substitutions. Nevertheless, the findings provide valuable support for the development of morphological and genetic study protocols.
This study was conducted in a traditional organic orchard during the autumnal generation and relied on pooled sequencing, yielding a consensus haplotype. While this approach provides a robust baseline, it also highlights the need for future individual-level analyses to capture intra-population mitochondrial diversity and haplotype frequencies. The present work delivers a morpho-genomic case study from a well-characterized agroecosystem, integrating field observations, quantitative morphological assessment, and mitogenomic data. The newly assembled mitogenome represents a high-quality dataset that expands the limited genomic resources currently available for Bactrocera oleae. Beyond its descriptive value, the reference sequence establishes a baseline for the development of molecular markers, haplotype tracking, and comparative analyses across Mediterranean olive systems.
While the results do not allow firm conclusions regarding local genetic adaptation, they underscore the value of integrating detailed morphological characterization with high-quality genomic data. The Órgiva population, although genetically consistent with the broader Mediterranean B. oleae lineage, exhibits clear local morphological variation. This integrated morpho-genomic approach provides a robust baseline for future comparative studies across cultivars, orchards, and management systems (organic versus conventional).
Ultimately, this work contributes a high-quality reference mitogenome and a reproducible framework for morphological analysis. These resources are particularly relevant for organic and low-input olive systems, where sustainable pest management is essential, and will facilitate the development of region-specific molecular tools to support effective, biodiversity-friendly strategies across the Mediterranean basin.
5. Conclusions
This study provides a high-quality reference mitogenome for B. oleae (15,810 bp, GenBank PZ179621) together with a detailed morphometric characterization of 140 adults collected from a traditional organic olive orchard in southern Spain. Multivariate analyses (PCA, hierarchical clustering, and LDA) supported the identification of six distinct morphological groups showing notable variation in thoracic pigmentation, abdominal banding, abdomen shape, and ovipositor morphology.
Adult longevity and fecundity assays revealed significant differences among these morphological groups. Flies with elongated ovipositors consistently exhibited higher longevity and greater reproductive success across Picual and Picholine cultivars, whereas compact forms tended to live shorter and produced fewer fertile punctures. These findings establish a functional link between morphological variation and fitness-related traits, underscoring the adaptive significance of phenotypic plasticity in this organic biotope.
Although the pooled nature of the mitogenome limits direct genotype–phenotype linkages, the very low genetic divergence (0.133 %) from Mediterranean references suggests that the observed phenotypic diversity is primarily driven by plasticity rather than strong genetic differentiation. These resources offer a valuable foundation for future comparative analyses, haplotype tracking, population monitoring, and investigations into phenotypic plasticity versus genetic adaptation in Mediterranean organic olive systems
Ethics and consent
Ethical approval and consent were not required









