Introduction
The pine processionary moth Thaumetopoea pityocampa (Lepidoptera, Notodontidae), is one of the major forest pests across the circum-Mediterranean countries that attacks all the Pinus and Cedrus species, both native and introduced, and occasionally other conifer species, namely those of the genus Pseudotsuga (Battisti et al., 2015; Carus, 2009; Sbay et Zas, 2018). Beyond its negative environmental impact resulting from tree defoliation, this species is a major public health concern due to the urticating setae that the larvae develop from the third instar (Battisti, Larsson, et Roques, 2017; Moneo et al., 2015). The geographic range of this pest extends from northern Africa to southern Europe, from the Atlantic coast to the western part of Turkey (EPPO, 2004; Kerdelhué et al., 2009; Roques et al., 2015). This species has a single generation per year, with adult emergence and oviposition occurring in summer, larval development during autumn and winter, and pupal diapause extending from late winter to summer. Huchon and Démolin (1970) showed that the distribution of this insect is strictly associated with climatic constraints, specifically winter and summer temperatures as well as annual sunshine duration, historically confining the species’ distribution to Mediterranean climates with warmer winter temperatures.
The pine processionary moth is one of the few species for which a causal relationship between climate warming and range expansion has been firmly demonstrated (Battisti et al., 2005; Rosenzweig et al., 2007). The northern edge of the species distribution was almost steady until the 1990s but records showed a significant expansion towards higher latitudes and elevations in southern Europe due to winter warming that has facilitated feeding in this winter-developing species and thus indirectly ascribed to improving survival and growth rates in newly colonized regions (Battisti et al., 2005; Robinet et al., 2007). Contrary to the beneficial effects of climate warming observed near the northern edge of the distribution, adverse effects have been reported at the southern edge in north Africa where local climate warming during summer and fall has contributed to increasing mortality rates of early life stages, leading to range retraction (Bourougaaoui et al., 2021). Monitoring the flight activity of this species is therefore crucial for assessing infestations risks in both forested and urban environments as well as early detection in new areas, given the species’ ongoing northward/uphill expansion in Europe, which, along with its southern retraction, serve as both an indicator of global warming and human-mediated transportation.
The accurate and timely detection of insect pests is crucial for effective forest health, biodiversity conservation, and crop protection (Ray et al., 2026). Traditional monitoring approaches, including visual scouting, sticky traps, pheromone traps, and light traps, have long been the cornerstone of pest surveillance (Elkinton & Cardé, 1981; Kammar et al., 2020; Roberts et al., 2025). In forestry, standard surveillance systems rely heavily on baited traps with lures and visual cues, that collect insects in buckets or collectors. These collectors require regular inspection and emptying by trained personnel to ensure regular functionality and to supply data for decision-making by forest managers. However, such systems present two major challenges: first, captured insects may disappear between the checks; second, these traps often capture non-target organisms, including natural enemies of the pests or other key elements of the forest food web (Battisti, 1989). Overall, these conventional techniques are labour-intensive because of frequent visits and time for checking, often yield delayed results that compromise timely pest management decisions, and are inadequate for detecting early-stage infestations.
The emergence of smart monitoring technologies represents a paradigm shift in how we detect and manage insect pest populations. The development of automated traps has seen a huge increase over the last decade, with widespread implementation in agriculture (Albanese et al., 2021; Brunelli et al., 2020; Sütő, 2021) but limited adoption in forest ecosystems. This disparity highlights a critical gap in forestry management tools, although the proven efficacy of automated systems in providing more accurate data for pest management, as demonstrated in agricultural context with species such as the codling moth (Cydia pomonella) in orchards in Italy (Preti et al., 2021).
Among the most prominent smart traps are camera-based traps integrated with deep learning models. These systems leverage on-board computing, edge AI, and low-cost hardware to achieve real-time detection and species-level classification. For instance, Bjerge et al. (2021) developed a light-table system powered by Raspberry Pi and convolutional neural networks (CNNs), achieving an F1 score of 0.93 in identifying moth species. Similarly, Sittinger et al. (2024) introduced a DIY solar-powered camera trap using YOLOv5 and EfficientNet-B0 models, reporting >90% accuracy for common hoverfly species. Other studies such as Novak et al. (2024) and Brunelli et al. (2020) deployed ultra-low-power CNNs on embedded microcontrollers (ESP32, GAP8) for robust insect detection, demonstrating strong performance (up to 88.8% F1 score) under favourable conditions. Yet, for most studies limitations such as image occlusion, environmental interference, and reduced accuracy in visually complex scenes remain common (Saradopoulos et al., 2023; Hong et al., 2021). In most systems, 10–15% of cases still require manual validation (Preti et al., 2021), and training datasets are often biased toward a few species, limiting scalability when the objective is to detect multiple species (Roy et al., 2024).
Optoelectronic, electrical impedance and infrared sensors offer an alternative non-visual detection pathway, especially suitable for night-active insects or confined environments. For example, Flórián et al. (2023) developed a sensor-equipped funnel trap with a blow-off system to prevent multiple counts, achieving 84–92% detection accuracy when tested on several moth species, including Agrotis segetum, Autographa gamma, Helicoverpa armigera, Cameraria ohridella, Grapholita funebrana, and Grapholita molesta. Welsh et al. (2022) combined optoelectronic wingbeat detection with machine learning to classify lepidopteran species, in multiple species target sampling, reporting >70% detection reliability. CapTrap® represents a commercial example of this approach, relying on motion-based infrared detection rather than imaging (Georgiev et al., 2025). These systems often excel in real-time performance yet overcounting due to re-entry and species calibration are noted challenges (Potamitis et al., 2017; Preti et al., 2021). Some setups, like the one of Rydhmer et al. (2022), utilize dual-wavelength near-infrared sensors and FPGA-based processing, but these often incur higher hardware and energy costs. RapidAIM exemplifies behavioural-sensor based detection (movement patterns such as walking dynamics and locomotion trajectories), displaying high autonomy and pre-capture identification. Yet, its limitations include possible overcounting from re-entry and higher hardware costs (Hamza et al., 2026). Crucially, because no images are captured in these advanced systems, validation of automated counts is not possible, making error tracking and species confirmation difficult.
Originally developed by the Slovenian company EFOS, the Trapview system is an automated monitoring tool primarily deployed for agricultural pests, such as the American grapevine leafhopper (Scaphoideus titanus) the main vector of phytoplasmas associated with flavescence dorée in vineyards (Ortis et al., 2025). By providing real-time, camera-based data on pest populations, it allows producers a quick reaction.
In this study, we evaluate the application of automated traps to detect and monitor the pine processionary moth. This is the first study, at the extent of our knowledge, that has analysed the application of this technology, and has been expanded beyond agriculture, to monitor major forest defoliators such as the pine processionary moth. We compare the efficiency of automated and conventional traps across different habitats in four countries under varying population densities. We further aim to analyse the ability of trap catches as predictor of nest density, the probability of detection at low densities allowing early detection systems, and the daily flight activity in relation to meteorological variables.
Materials and methods
Study regions and trap locations
We selected sites where traps are traditionally used for surveillance, covering both forest and urban habitats. The study was conducted in four countries (
Table 1).
Table 1. List of the sites where surveillance devices were deployed.
|
Country |
Site coordinates (centroid of all traps) |
Elevation of the centroid (m) | Setting | Tree |
Number of traps | Deployment period (day/month) |
|---|
| forest/urban | species* | auto/conv | |
|---|
| France | 47.833670 N, 2.450634 E | 146 | Forest | PS/PN | 6/4 | 27/05 to 17/10 |
| 47.846235 N, 1.923284 E | 106 | Urban | PN | 6/5 | 28/05 to 17/10 |
| Italy | 46.630154 N, 10.805001 E | 951 | Forest | PN, PS | 10/9 | 16/06 to 04/09 |
| Portugal | 38.835777 N, −8.849344 W | 26 | Forest | PPi | 5/5 | 21/07 to 01/10 |
| 38.713961 N, −9.188228 W | 114 | Urban | PP | 5/5 | 21/07 to 01/10 |
| Slovenia | 45.599402 N, 13.937283 E | 494 | Forest | PN | 5/5 | 26/06 to 03/10 |
| 45.602344 N, 13.941606 E | 491 | Urban | PN | 5/5 | 26/06 to 03/10 |
France – The study area is located in the metropolitan area of Orléans which displays a mix of densely urbanized areas to forest or agricultural lands on its periphery. Host trees are found as street or isolated trees, groves or small stands scattered over the city (Rossi et al., 2016). Orléans is bordered on the northeast by the Orléans Forest, the biggest state-owned forest in France, and on the south by the Sologne forest. The forested areas of the region are composed of coniferous or mixed stands and broadleaved stands. Pinus nigra and P. sylvestris are the most frequent hosts in Orléans region. Our study area corresponds to the northern distribution of the insect in the Paris Basin, where it has continuously progressed northward since the 1990s, at an average speed of 5 km per year (Battisti et al., 2005). The Orléans region is located in the southern Paris basin and has been definitively colonized since 35 years. A total of twelve automated traps were deployed, with six located in urban sites within Orléans city and six in the Orléans forest. Additionally, nine conventional traps were set up at the same locations as the automated traps, including five in urban areas and four in forest sites (
Table 1).
Italy – The Venosta/Vinschgau valley, located in the mountains of south Tyrol at the intersection of Italy, Austria, and Switzerland, is characterized by an east-west orientation with contrasting north and south-facing slopes (Battisti et al., 2005). The study area is located in the current upper altitudinal distribution in the southern-central Alps, reaching 1500 m on south-facing slopes and 1200 m on north-facing slopes following recent winter warming. Infested stands are largely located on south-facing slopes and consist of mixed forests of native Scots pine (Pinus sylvestris) and introduced black pine (Pinus nigra). A total of ten automated traps were deployed in forest sites. In addition, we installed nine conventional traps in proximity to the automated trap sites.
Portugal – Two sampling sites were selected, one in an urban area in the city of Lisbon, and the other in a forest area about 50 km northeast. The forest sampling site is located within a property belonging to the Companhia das Lezírias. This pine forest covers approximately 1000 hectares and consists predominantly of maritime pine (Pinus pinaster), managed for timber production. The selected sampling plot is situated in the interior of the pine forest, away from edges and boundaries, representing the average conditions of the productive stand. Within this plot, the traps were arranged in two parallel lines spaced 50 m apart. Along these lines, automated traps and conventional traps were placed alternating and intercalated with each other. The urban site is located in Tapada da Ajuda, in the university campus, the main conifer tree species in this area are umbrella pines (Pinus pinea) together with many other conifer and broadleaf trees. A total of 20 traps were deployed, 10 in the urban area and 10 in the forest. In each site, five automated traps and five conventional traps were set up.
Slovenia – The study was conducted in and around the village of Hrpelje, located near Kozina in the south-western part of Slovenia, within the sub-Mediterranean biogeographical region. Hrpelje is a suburban area situated at the forest edge, where urban landscapes include numerous Austrian pine trees (P. nigra) planted in gardens and along roads. The surrounding environment consists of coniferous to mixed forest stands, with P. nigra being the dominant pine species. The pine processionary moth is present in the western part of Slovenia, where this study area lies near the edge of its distribution range. To assess trap performance across habitat types, a total of 20 traps were deployed. Five automated traps were installed in the urban area and five in the forest, complemented by five conventional traps in each habitat.
Trap types and deployment
For automated monitoring, we used Trapview FUNNEL SC traps (
Figure 1), which are specifically designed for larger moths. The trap entrance is the same as with conventional bucket/unitrap. When entering the trap, moths fall into the trap body, where they get stuck to the sticky surface. Main sensors of the automated trap are high resolution cameras (each 8Mpix), which are responsible for image captures (three images were captured at fixed time intervals during the night (at 23:00, 02:00, and 05:00 In France, Italy, and Slovenia, and at 00:00, 03:00, and 06:00 in Portugal, accounting for time differences). Images of captured moths, temperature and humidity data and the state of the device are then sent via cellular network to the cloud, where they are stored and processed before shown to the user through a web application. The trap has a self-cleaning feature which means the exposed sticky surface to which insects are caught is part of a sticky tape which rolls over daily to avoid surface saturation. This glued surface is provided as a roll that enables automatically daily change of the sticky paper over a 30-day period. Electronics are powered by the combination of solar panel and battery, while temperature and humidity sensors housed outside the trap collect data every five minutes. The traps were mounted on poles at about 2 m from the ground.
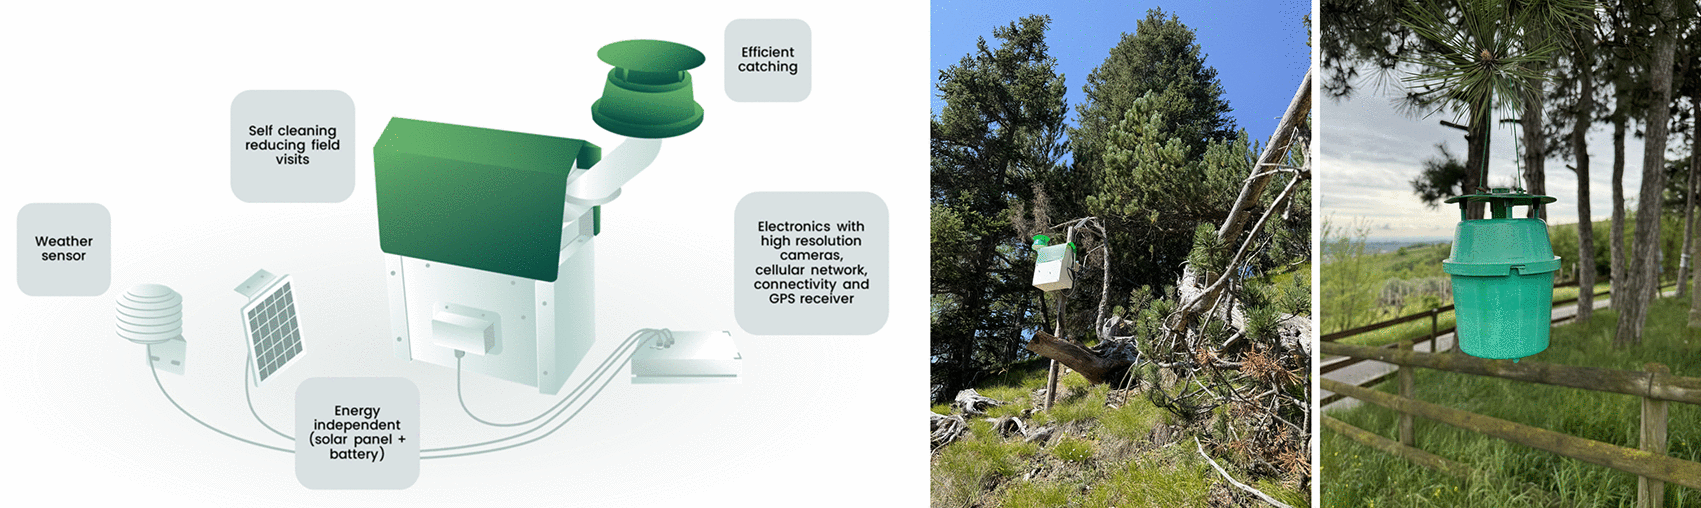
Figure 1. Schematic representation of the automated trap (left), the automated trap (centre) and a conventional funnel trap (right) deployed on the ground.
For conventional monitoring, we used standard bucket/unitrap traps for large moths (
Figure 1), with catches recorded manually by counting the males in the collector under the funnel on a weekly basis. The traps were mounted on poles at the same height as the automated traps.
Both types of traps were installed about one to two weeks prior to the expected onset of the flight period in each region, with an approximate distance of 500 m between traps. All traps were baited with the long-life dispensers (10 mg) of sexual pheromone provided by Pherobank®, which covers the entire flight period (unpublished results from previous year trials).
Image assessment and accuracy validation
Identification of the target insects was implemented via deep learning, specifically based on the Faster R-CNN algorithm. For the training of pine processionary moth recognition model, over 1,600 manually annotated images were used. Model performance was evaluated using mean Average Precision (mAP), a common measure that is used as a single number that summarizes how well the model detects the objects in which values closer to 1 indicate higher detection performance. The initial evaluation was based on 117 images collected since 1st July 2025 from limited number of traps installed in the beginning of the flight season. As trap deployment was not complete during the initial assessment, manual validation was conducted in the present study using images from all automated traps deployed in Portugal during the entire flight period.
The performance of the automated traps was evaluated using a confusion matrix approach based on manual validation of approximately 2,220 images per period. Two distinct levels of moth activity were considered; low and high catch thresholds, resulting in a total of 4,440 validated images. The same 10 traps were evaluated in both periods, and 3 images were examined per trap and per day. AI predictions were compared with manual visual classifications at the corresponding evaluated image positions. True positives (TP) corresponded to AI detections confirmed by human eye visual counting, while true negatives (TN) were evaluated positions that did not contain moths, but could contain another insect, a leaf, or other debris and AI correctly did not classify as pine processionary. False positives (FP) occurred when the AI incorrectly identified a moth, due to the misclassification of non-target moth species. False negatives (FN) corresponded to moths not detected by the AI but seen by human eye. Separate confusion matrices were produced for low and high activity periods and reported in supplementary material (Table S1). Based on these classifications, performance metrics were calculated, including precision (TP/(TP + FP)), which reflects how often positive detections are correct; recall or sensitivity (TP/(TP + FN)), indicating the proportion of actual moths correctly detected; accuracy ((TP + TN)/N), representing overall correctness; and the F1-score (2× (Precision × Recall) / (Precision + Recall)), which balances precision and recall.
The effectiveness of the automated traps in retaining moths on the sticky paper was assessed in Italy by comparing detection on consecutive images. Movement was expected to be less at low catches, when the sticky surface was largely exposed, resulting in direct contact between moths and the adhesive, and higher at high catches, when trapped moths largely covered the sticky surface allowing newly arriving moths to land over them. The relationship between total trap catch and movement rate (%) was assessed using simple linear regression. Total catch was considered a proxy for trap saturation, as higher catch may reduce the exposed sticky surface available to retain newly arriving moths.
Trap catch as an indicator of infestation level
Local infestation levels were quantified through a standardized assessment of larval nest density across each study region in the winter following trap deployment. At every trapping site, a visual survey was conducted on the nearest 30 trees surrounding each trap to record the number of nests, using binoculars when nests were high in the canopy and difficult to spot. This protocol provided a localized estimate of infestation, allowing a comparative analysis between adult male catch and actual larval presence in the field. To facilitate comparison with the French dataset, where infestation was assessed at the hectare scale, nest counts were standardized to a 1 ha area.
For each trap location, a circular buffer with a radius of 56.4 m (corresponding to approximately 1 ha) was generated in QGIS using Google Earth satellite imagery as background layer. Within each buffer, forest cover was delineated and measured to estimate the proportion of forest cover. In addition, all visible trees within the buffer were counted from satellite imagery to estimate tree density. The proportion of pine trees within the forested area was obtained from local stand information. Nest density per hectare was then estimated as:
where:
N30 = number of nests counted on the 30 surveyed trees.
Pforest = proportion of forest cover within the 1 ha buffer.
Ppines = proportion of pine trees within the forested area.
TreeD = tree density (trees ha−1).
In Portugal and Slovenia nest occurrence was extremely low, with most sampling spots recording zero nests in both forest and urban habitats. This lack of variation resulted in highly zero-inflated datasets and prevented the assessment of meaningful relationships between trap catch and infestation level in these countries.
Assessment of non-target organisms and predation
Non-target captures were assessed in Italy and Portugal only, representing contrasting population levels, high and low, respectively. In Italy, insects retained on the sticky papers of four traps representing different catch density, from very low to very high, were counted and identified at a group level. Hymenopteran parasitoids were examined using a binocular microscope. In Portugal, non-target captures were assessed by counting the individuals from the bulk catch in conventional traps during weekly inspections, and individuals were identified and assigned to major taxonomic groups.
Predation in automated traps was assessed using images from both countries. The image records were examined for evidence of predator activity on captured moths. Predation was inferred when predators were observed on the sticky surface together with signs of feeding or partial removal of moths, such as the presence of detached wings, antennae, or other moth remains.
Statistics
Differences in moth catch between automated and conventional traps were analysed using generalized linear models (GLMs). Because count data showed overdispersion, negative binomial models with a log-link function were performed. The response variable was the number of moths captured, while trap type, habitat, and country were included as explanatory variables. Country-specific analyses were subsequently performed to compare traps within each habitat. Estimated marginal means were obtained using the emmeans package, and pairwise comparisons between trap types were expressed as rate ratios with associated z-ratios and p-values.
The timing of first moth detection was determined for each trap using daily records. For each automated and conventional trap, the first detection date was defined as the first Julian day on which at least one individual was caught. To compare detection timing between trap types, paired t-tests were performed separately for each country within each habitat. Differences were expressed as mean differences in Julian days between automated and conventional traps. To explore geographic variation in detection timing, analyses were conducted using automated traps only. First detection dates were compared among countries using a one-way analysis of variance (ANOVA), pooling data across habitats. To evaluate habitats effects, first detection dates were compared between forest and urban environments within each country using independent two-sample t-tests.
To evaluate the probability of detection of automated and conventional traps at low population density, a binary variable was created for each trap based on captures recorded during the first four weeks of the flight activity following the first detection date, as a proxy of low density. Traps that captured at least one moth were assigned to a value of 1, whereas traps with no captures were assigned to a value of 0. For each country and habitat, the proportion of traps with successful detections were compared between automated and conventional traps using Fisher’s exact test. This test was chosen because some contingency tables contained small sample sizes and low expected frequencies. Separate analyses were performed for each habitat within each country and for pooled data at the country level.
To evaluate the effect of temperature and humidity on automated trap catch, we calculated nightly average of these variables over the interval from 21:00 to 06:00, corresponding to the main flight window. For each trap and date, daily catch values were then averaged across traps within each country and habitat to obtain standardized daily catch per trap. To focus the analysis on the time when moths were more active, we used a core period defined by the 20th and 80th percentiles of the distribution date within each country and habitat. Finally, linear regressions were performed separately for each country and habitat.
To test the relationships between catch and local infestation level, linear regression analyses were used. Nest density (number per ha) was used as the response variable and total trap catch as the explanatory variable. Because the number of traps within each country and trap type was relatively limited, data from France and Italy were pooled to increase the sample size. Separate regressions were then performed for conventional and automated traps. The strength of the relationships was assessed using the coefficient of determination (R2), and the statistical significance was evaluated using the p-value associated with the regression slope.
Results
Automated traps recorded consistently higher mean catch than conventional traps at all sites and across different population densities (
Figure 2). In Italy (forest habitat only), automated traps captured 7.2 times more moths than conventional traps (automated/conventional ratio = 0.138, p < 0.001, negative binomial model). In French forest the ratio was similar (0.115, p < 0.001) while in urban settings the catch was higher and the ratio 11.9-fold higher than in the forest (ratio = 0.0084, p < 0.001). In Portugal, the catch was low in forest and very low in urban settings, with a 3.5-fold (ratio = 0.287, p < 0.001) and 5.4-fold (ratio = 0.184, p < 0.001) increase in catches for automated traps, respectively. In Slovenia, catch was very low and more similar between trap types (forest ratio = 0.764, urban ratio = 0.851; p > 0.05).
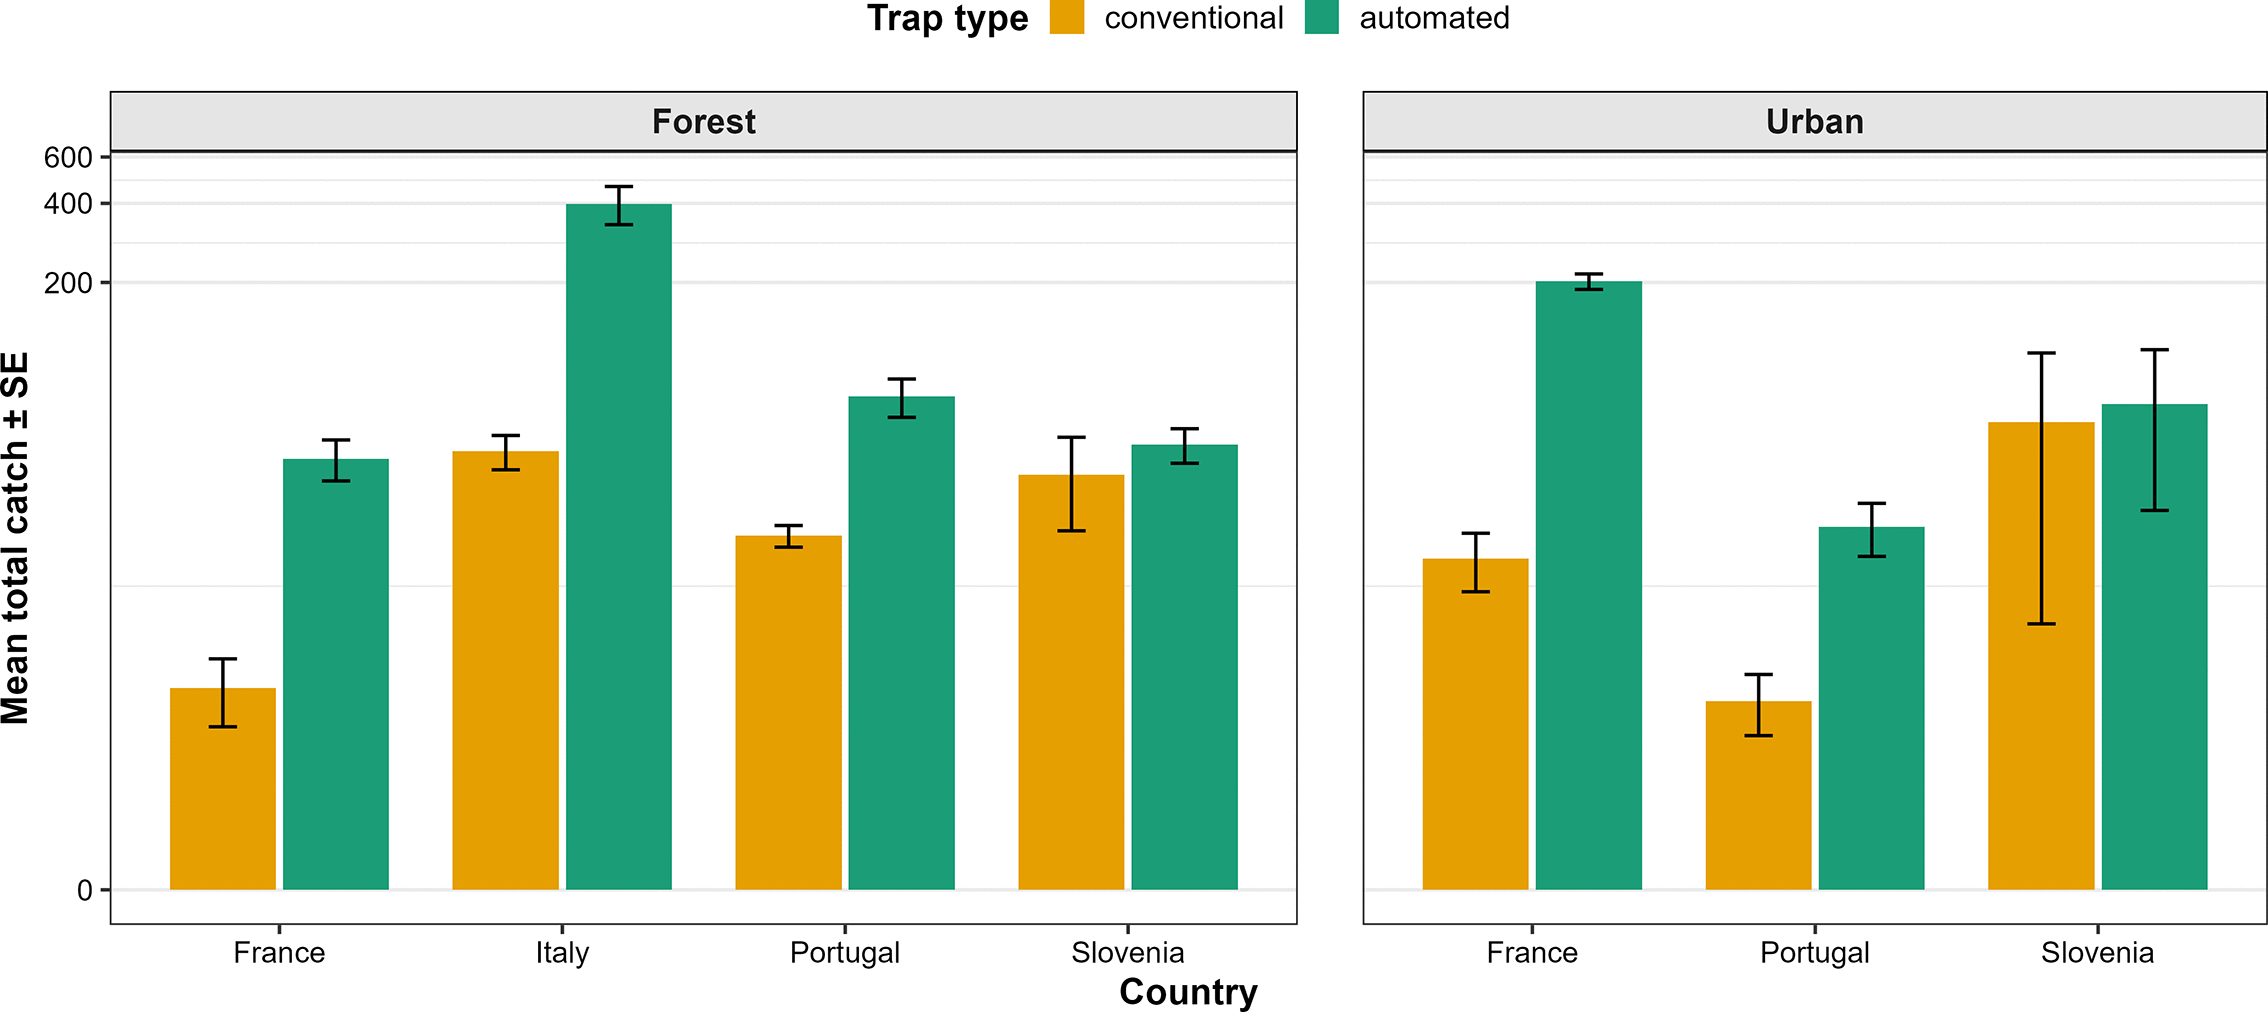
Figure 2. Mean total catch (±SE) recorded by automated and conventional traps across habitats and countries.
For visualization purposes, the y-axis was displayed using a natural logarithmic scale to improve the readability of differences among trap types and countries.
The AI model achieved a very high detection performance, with a mean Average Precision (mAP) of 0.98, indicating high accuracy in identifying pine processionary moths. Automated traps demonstrated high performance across both low and high catch periods. During the low-density period, the system achieved perfect performance, with precision, recall, accuracy, and F1-score all equal to 1, indicating the absence of both false positives and false negatives. As expected, the lower number of catches facilitated image interpretation and resulted in error-free detection. During the high-density period, performance remained very high, with a precision of 0.985, recall of 0.988, accuracy of 0.975, and an F1-score of 0.987. The few false positives recorded (n = 6) were mainly associated with wing scales imprints or occasional misclassification of non-target species, whereas false negatives (n = 5) corresponded to a small number of visible moths that were not detected by the system.
Moth movement on the sticky paper varied substantially among traps, ranging from 1.0% to 53.5% (mean = 21.6%). No clear relationship was observed between total catch and movement rate. It should be noted, however, that rates were always evaluated at high trap catch densities typical of the Italian site, ranging from 225 to 830 moths.
As expected, flight patterns varied by country, with activity occurring later in warmer areas (
Figure 3). First detection dates differed between automated and conventional traps depending on country and habitat. In forest habitats, automated consistently detected moth activity earlier than conventional traps. These differences were statistically significant in France (mean difference = −10.3 days, p = 0.037), Italy (−7.8 days, p = 0.0075), and Portugal (−5.2 days, p = 0.039). On the other hand, no significant differences were observed in Slovenia (−1.25 days, p = 0.726). In urban habitats, differences between trap types were smaller and not statistically significant across countries (France: −1.5 days, p = 0.137; Portugal: −6.8 days, p = 0.216; Slovenia: −4.8 days, p = 0.478). Overall, these results indicate that automated traps provide earlier detection especially in forest environments. First detection dates varied markedly among countries (ANOVA, p < 0.001) with Italy being the earliest (Julian day average = 173), followed by France (day 178), then Slovenia (day 192) and Portugal, which showed the latest detections (day 216). The habitat influenced first detection only in France, with moths appearing earlier in urban areas (mean Julian day = 176) than in forests (mean Julian day = 180) (p = 0.028). The tendency was the same in Portugal and Slovenia, but differences were not significant. When the first four weeks of moth catch were considered, as a proxy of low population density, automated detected moth in a greater percentage than conventional traps (
Table 2). When data from all countries were pooled, automated showed a two-fold higher detection rates than conventional traps, with significant results in both urban and forest habitats.
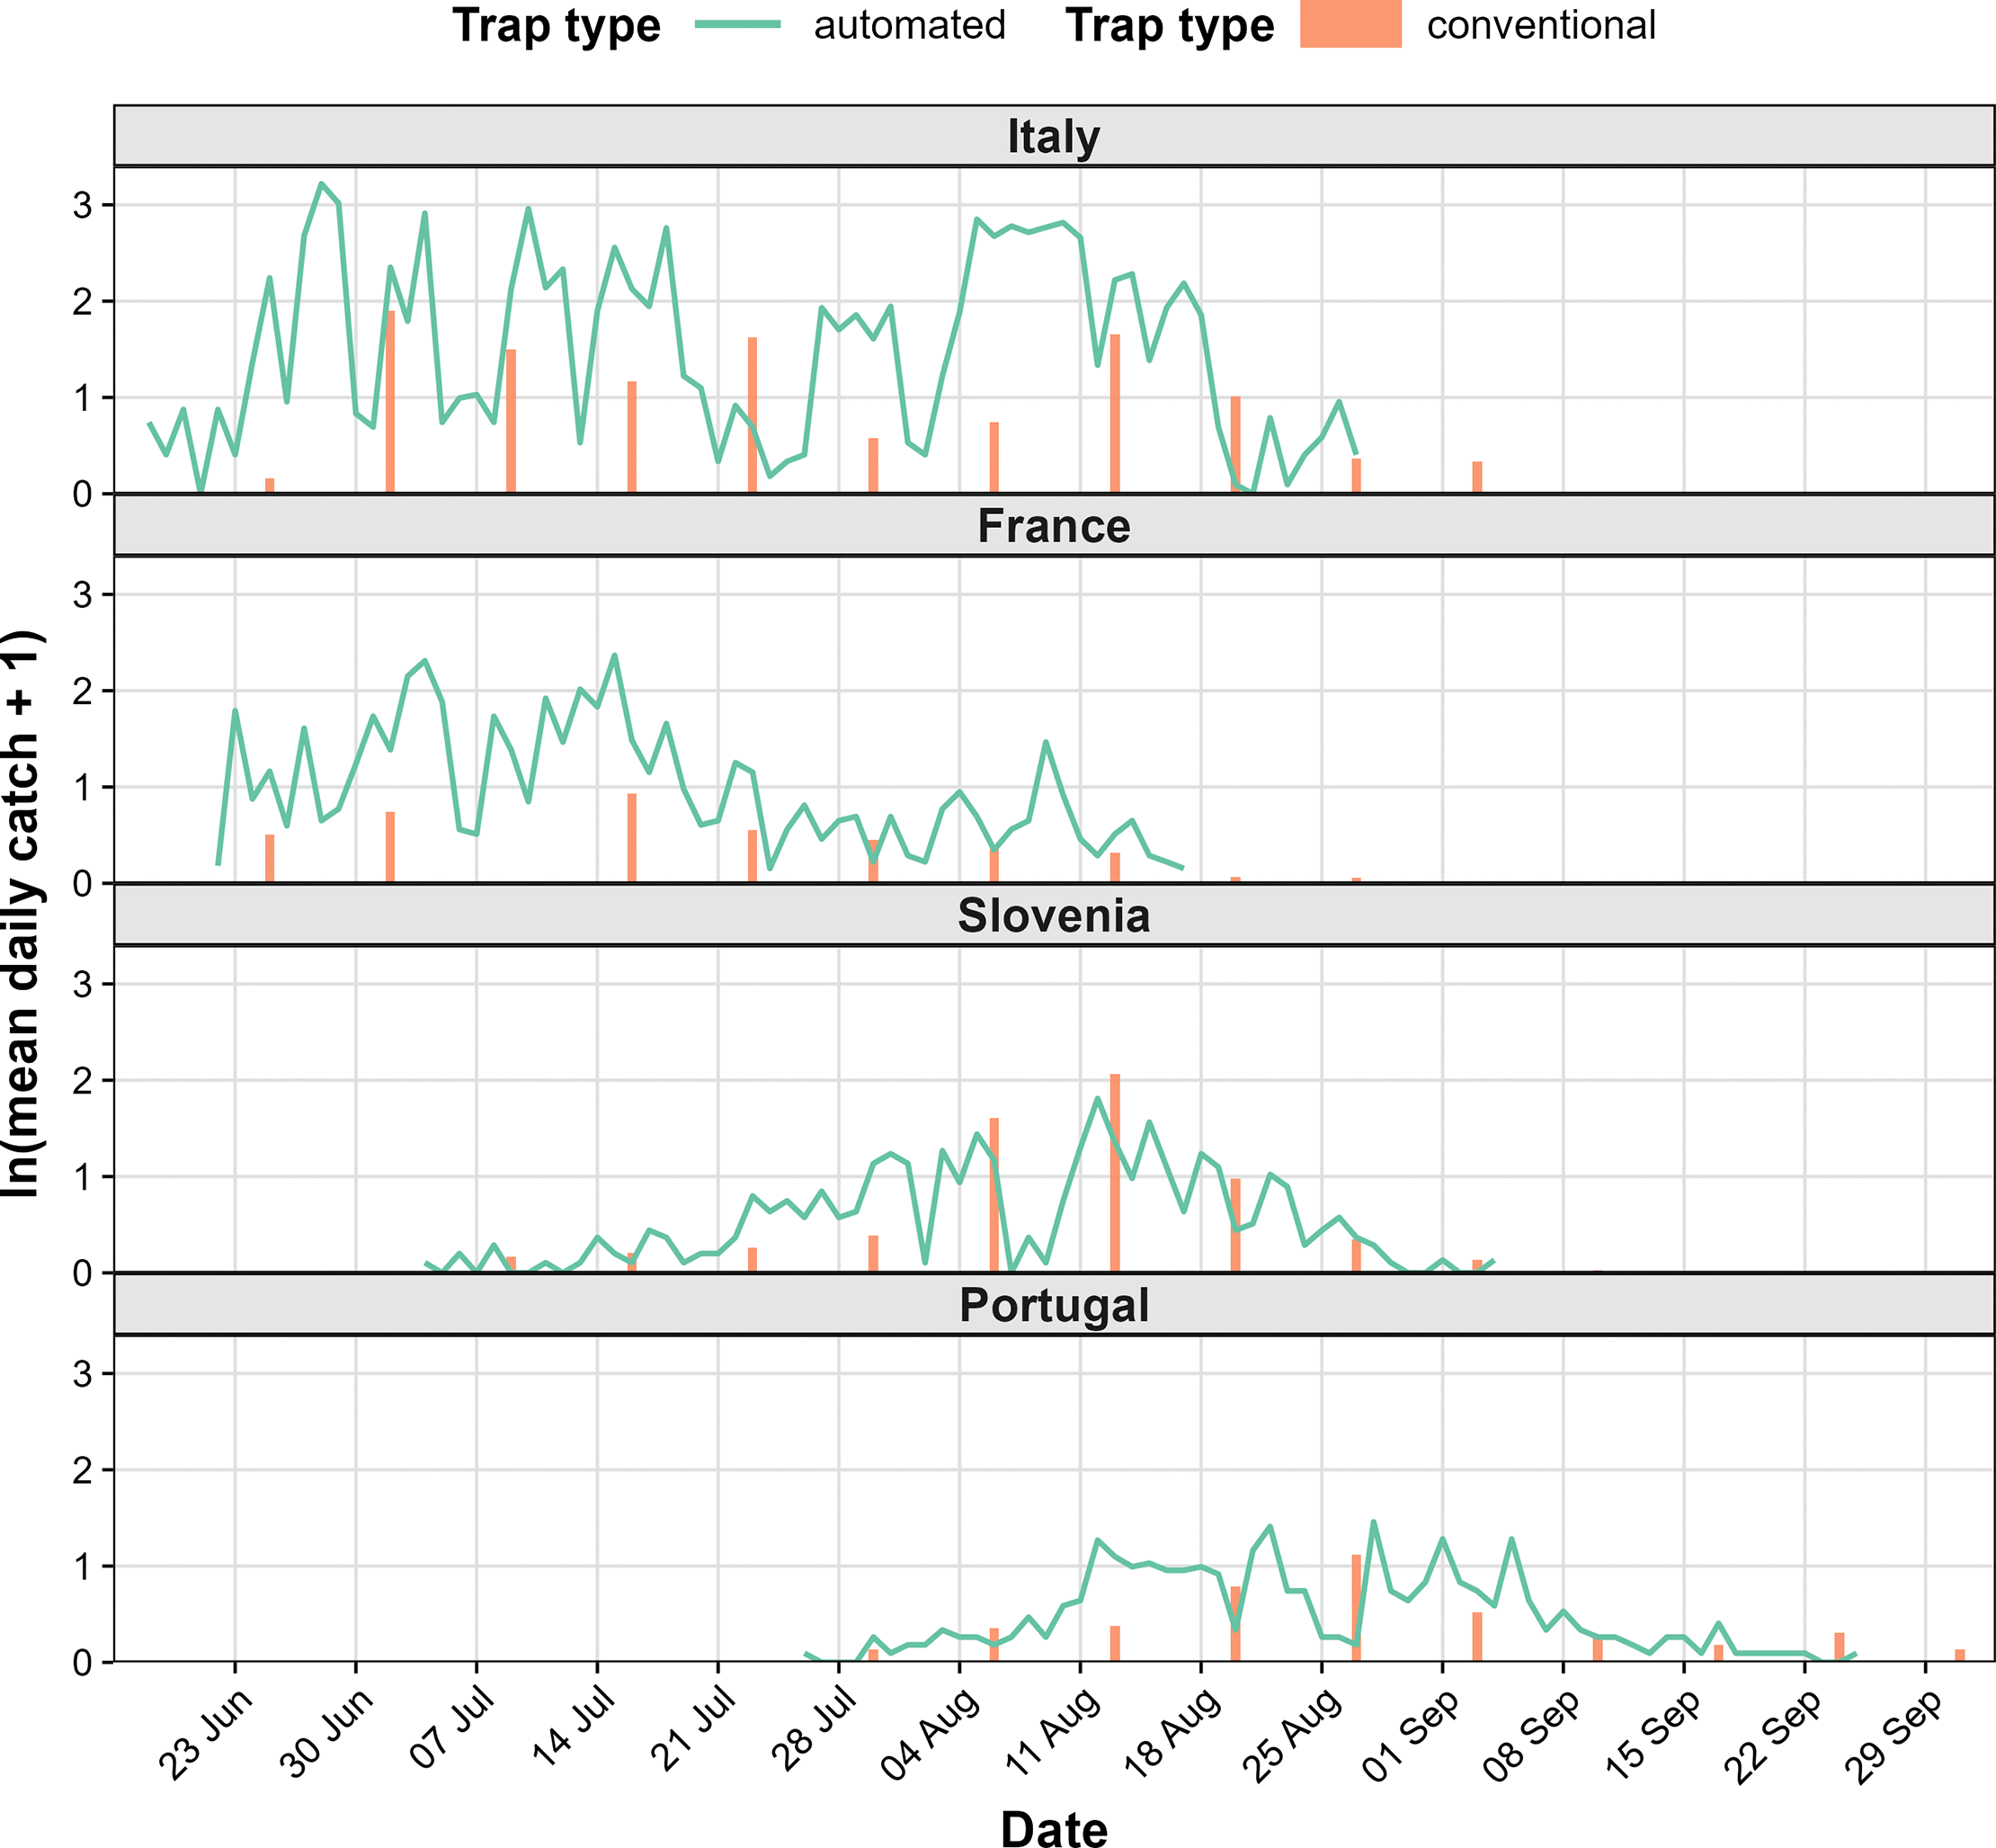
Figure 3. Temporal dynamics of daily moth catch recorded by automated and conventional traps in Italy, France, Slovenia, and Portugal, ordered by the time of first catch.
Daily catch was standardized using ln(x + 1).
Table 2. Proportion of positive traps (%) detecting pine processionary moth using automated and conventional traps across countries and habitats.
Fisher’s exact tests were used to compare detection rates between trap types.
| Habitat | Automated trap % | Conventional trap % |
Fisher’s exact test p value |
|---|
| Italy | Forest | 85.0 | 25.0 | <0.001 |
| France | Urban | 100 | 75.0 | 0.022 |
| Forest | 95.8 | 45.8 | <0.001 |
| All | 97.9 | 60.4 | <0.001 |
| Portugal | Urban | 70.0 | 40.0 | 0.111 |
| Forest | 50.0 | 30.0 | 0.333 |
| All | 60.0 | 35.0 | 0.043 |
| Slovenia | Urban | 80.0 | 26.7 | 0.009 |
| Forest | 37.5 | 12.5 | 0.220 |
| All | 58.1 | 19.4 | 0.004 |
| All countries | Urban | 84.7 | 50.8 | <0.001 |
| Forest | 73.0 | 29.0 | <0.001 |
| All | 77.4 | 37.1 | <0.001 |
Temperature generally acted as a key driver of moth catch, with clear significant positive relationships observed in Italy (p < 0.001), France (urban: p = 0.031; forest: p = 0.0018), and Slovenia forest sites (p = 0.0012), where warmer nights lead to increased catches (
Figure 4). Yet, this effect is strongly habitat dependent. In Portugal, contrasting patterns were observed between habitats: moth catch decreased significantly with increasing temperature in forest sites (p = 0.0042), whereas a significant positive relationship was found in urban areas (p = 0.0051). In Slovenia, temperature significantly increased moth catch in forests (p = 0.0012) but had no detectable effect in urban habitats (p = 0.90). In contrast, relative humidity was generally negatively associated with moth catch. Significant negative relationships were observed in France (forest: p = p < 0.001; urban: p = p < 0.001), Italy (p = 0.0021), Slovenia forest sites (p = p < 0.001), and Portugal urban sites (p = 0.006) (
Figure 5), indicating reduced catch under more humid conditions. No significant relationships with humidity were detected in Portugal forest sites (p = 0.32), and the difference was marginal in Slovenia urban sites (p = 0.055) (
Figure 5).
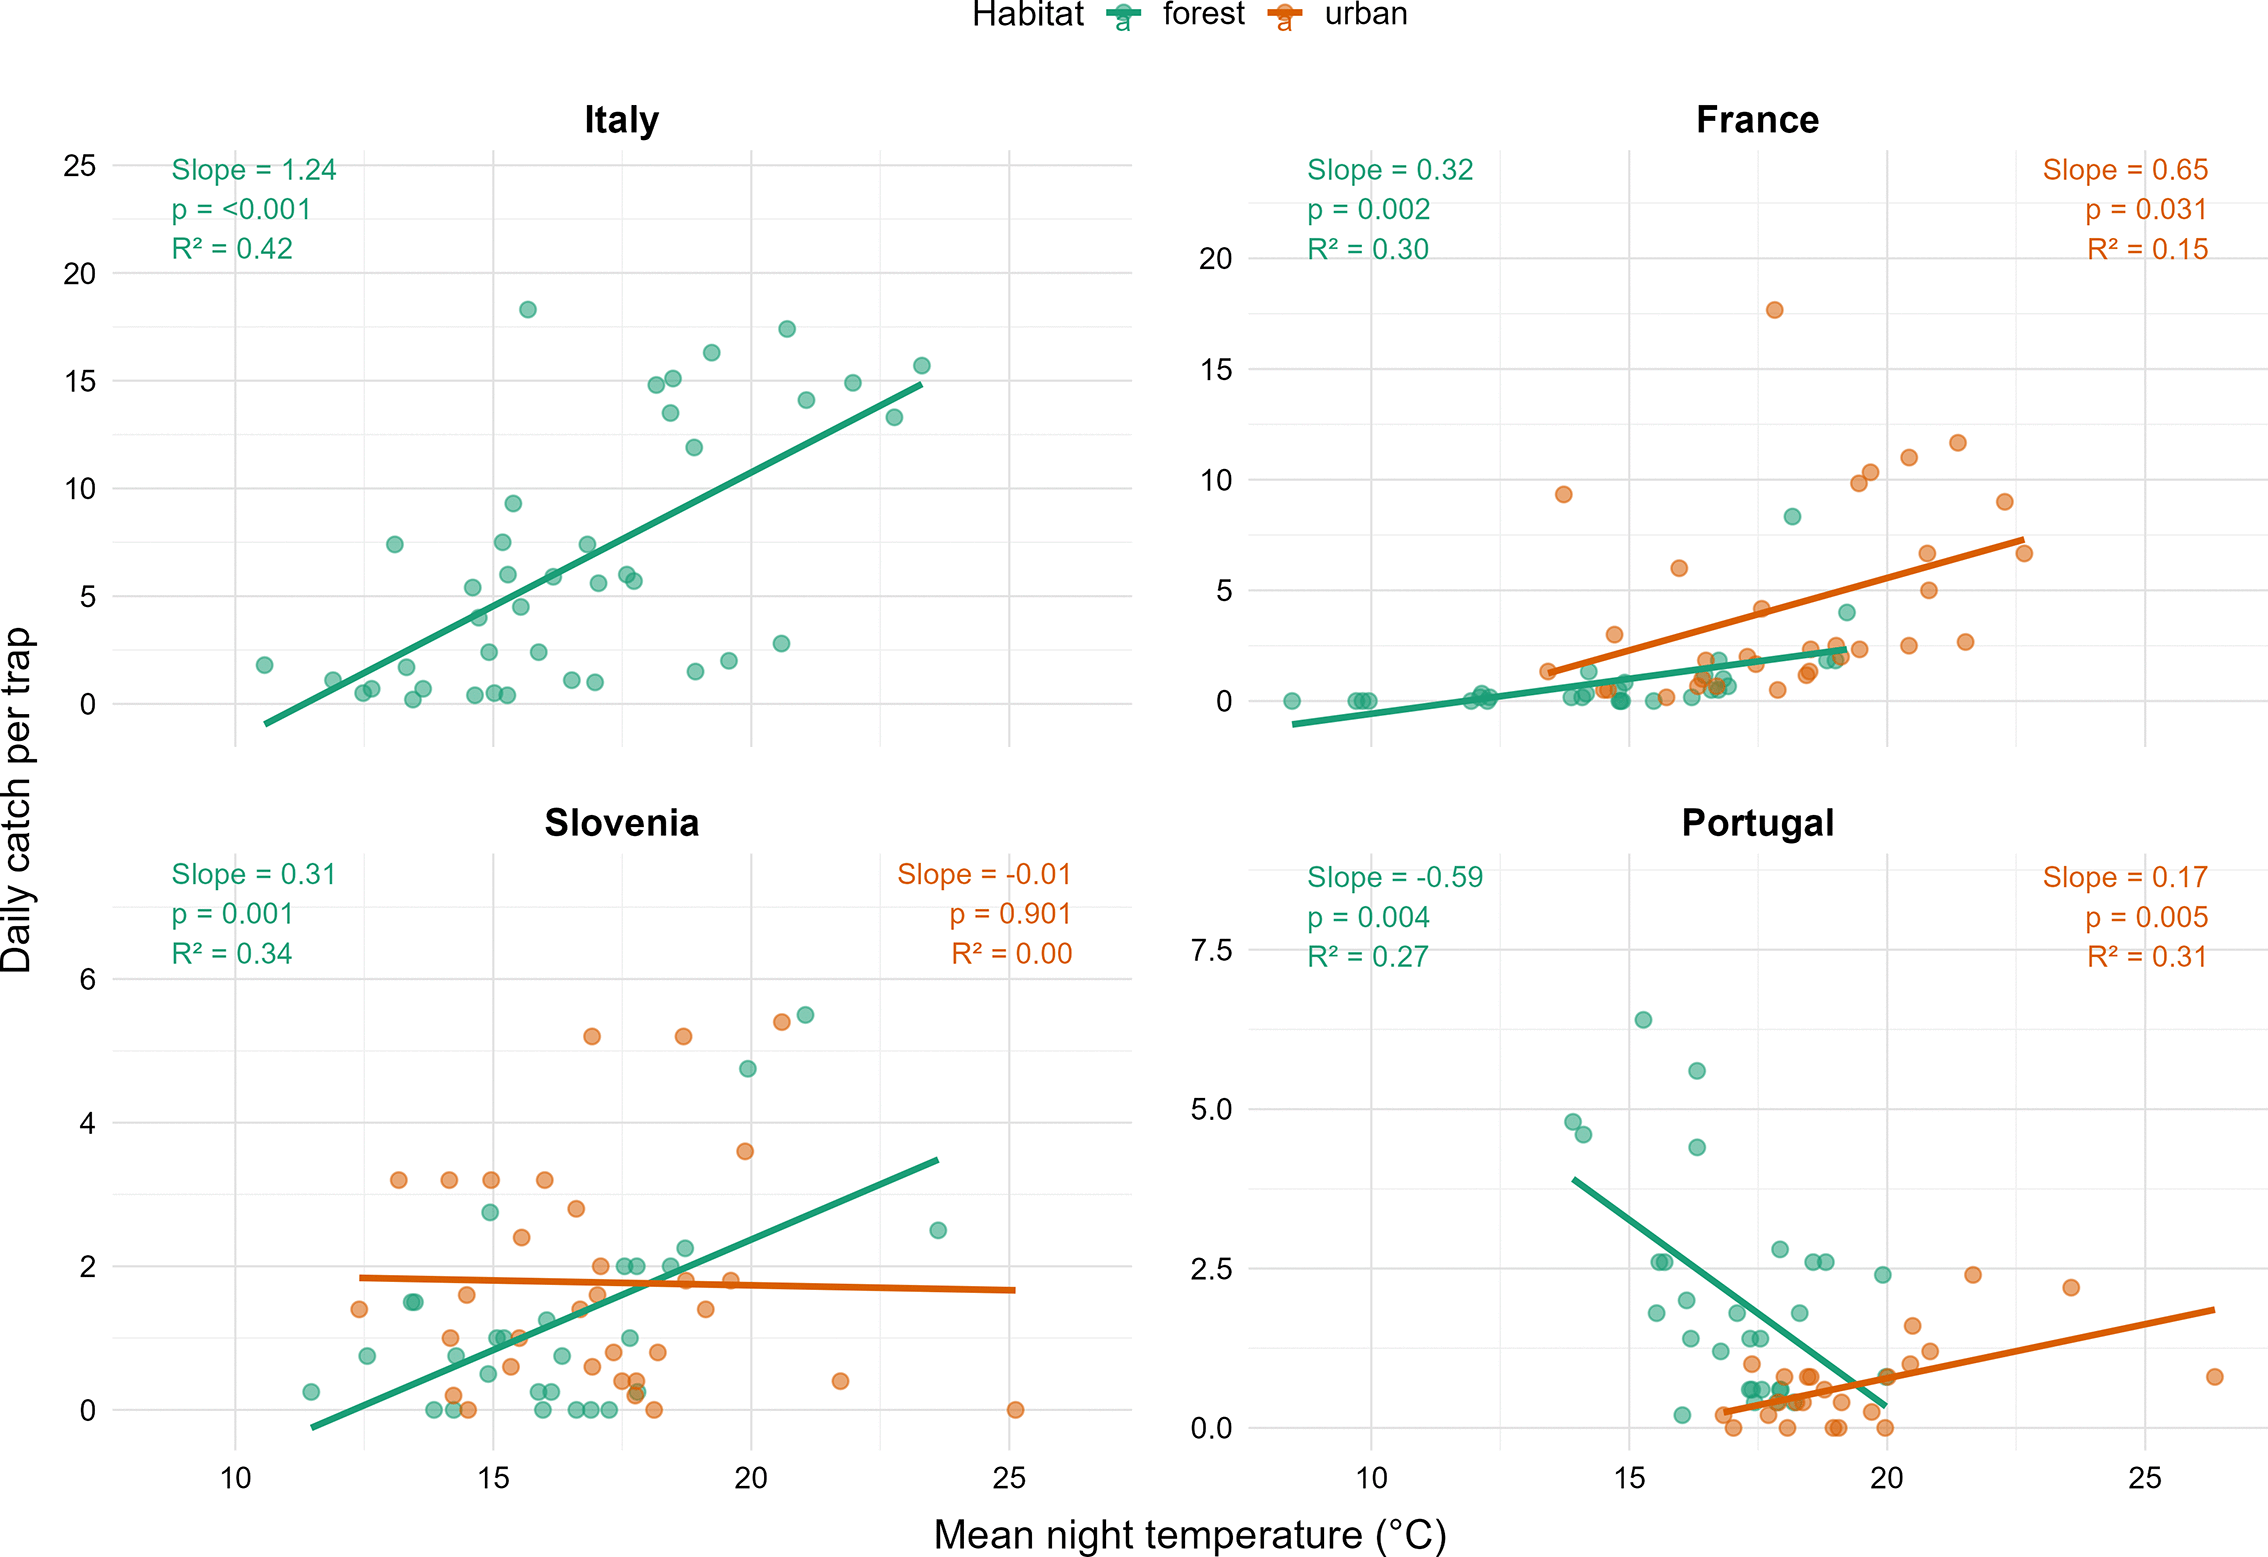
Figure 4. Relationships between mean night temperature and trap catch in automated traps during the central flight period (20–80% quantile).
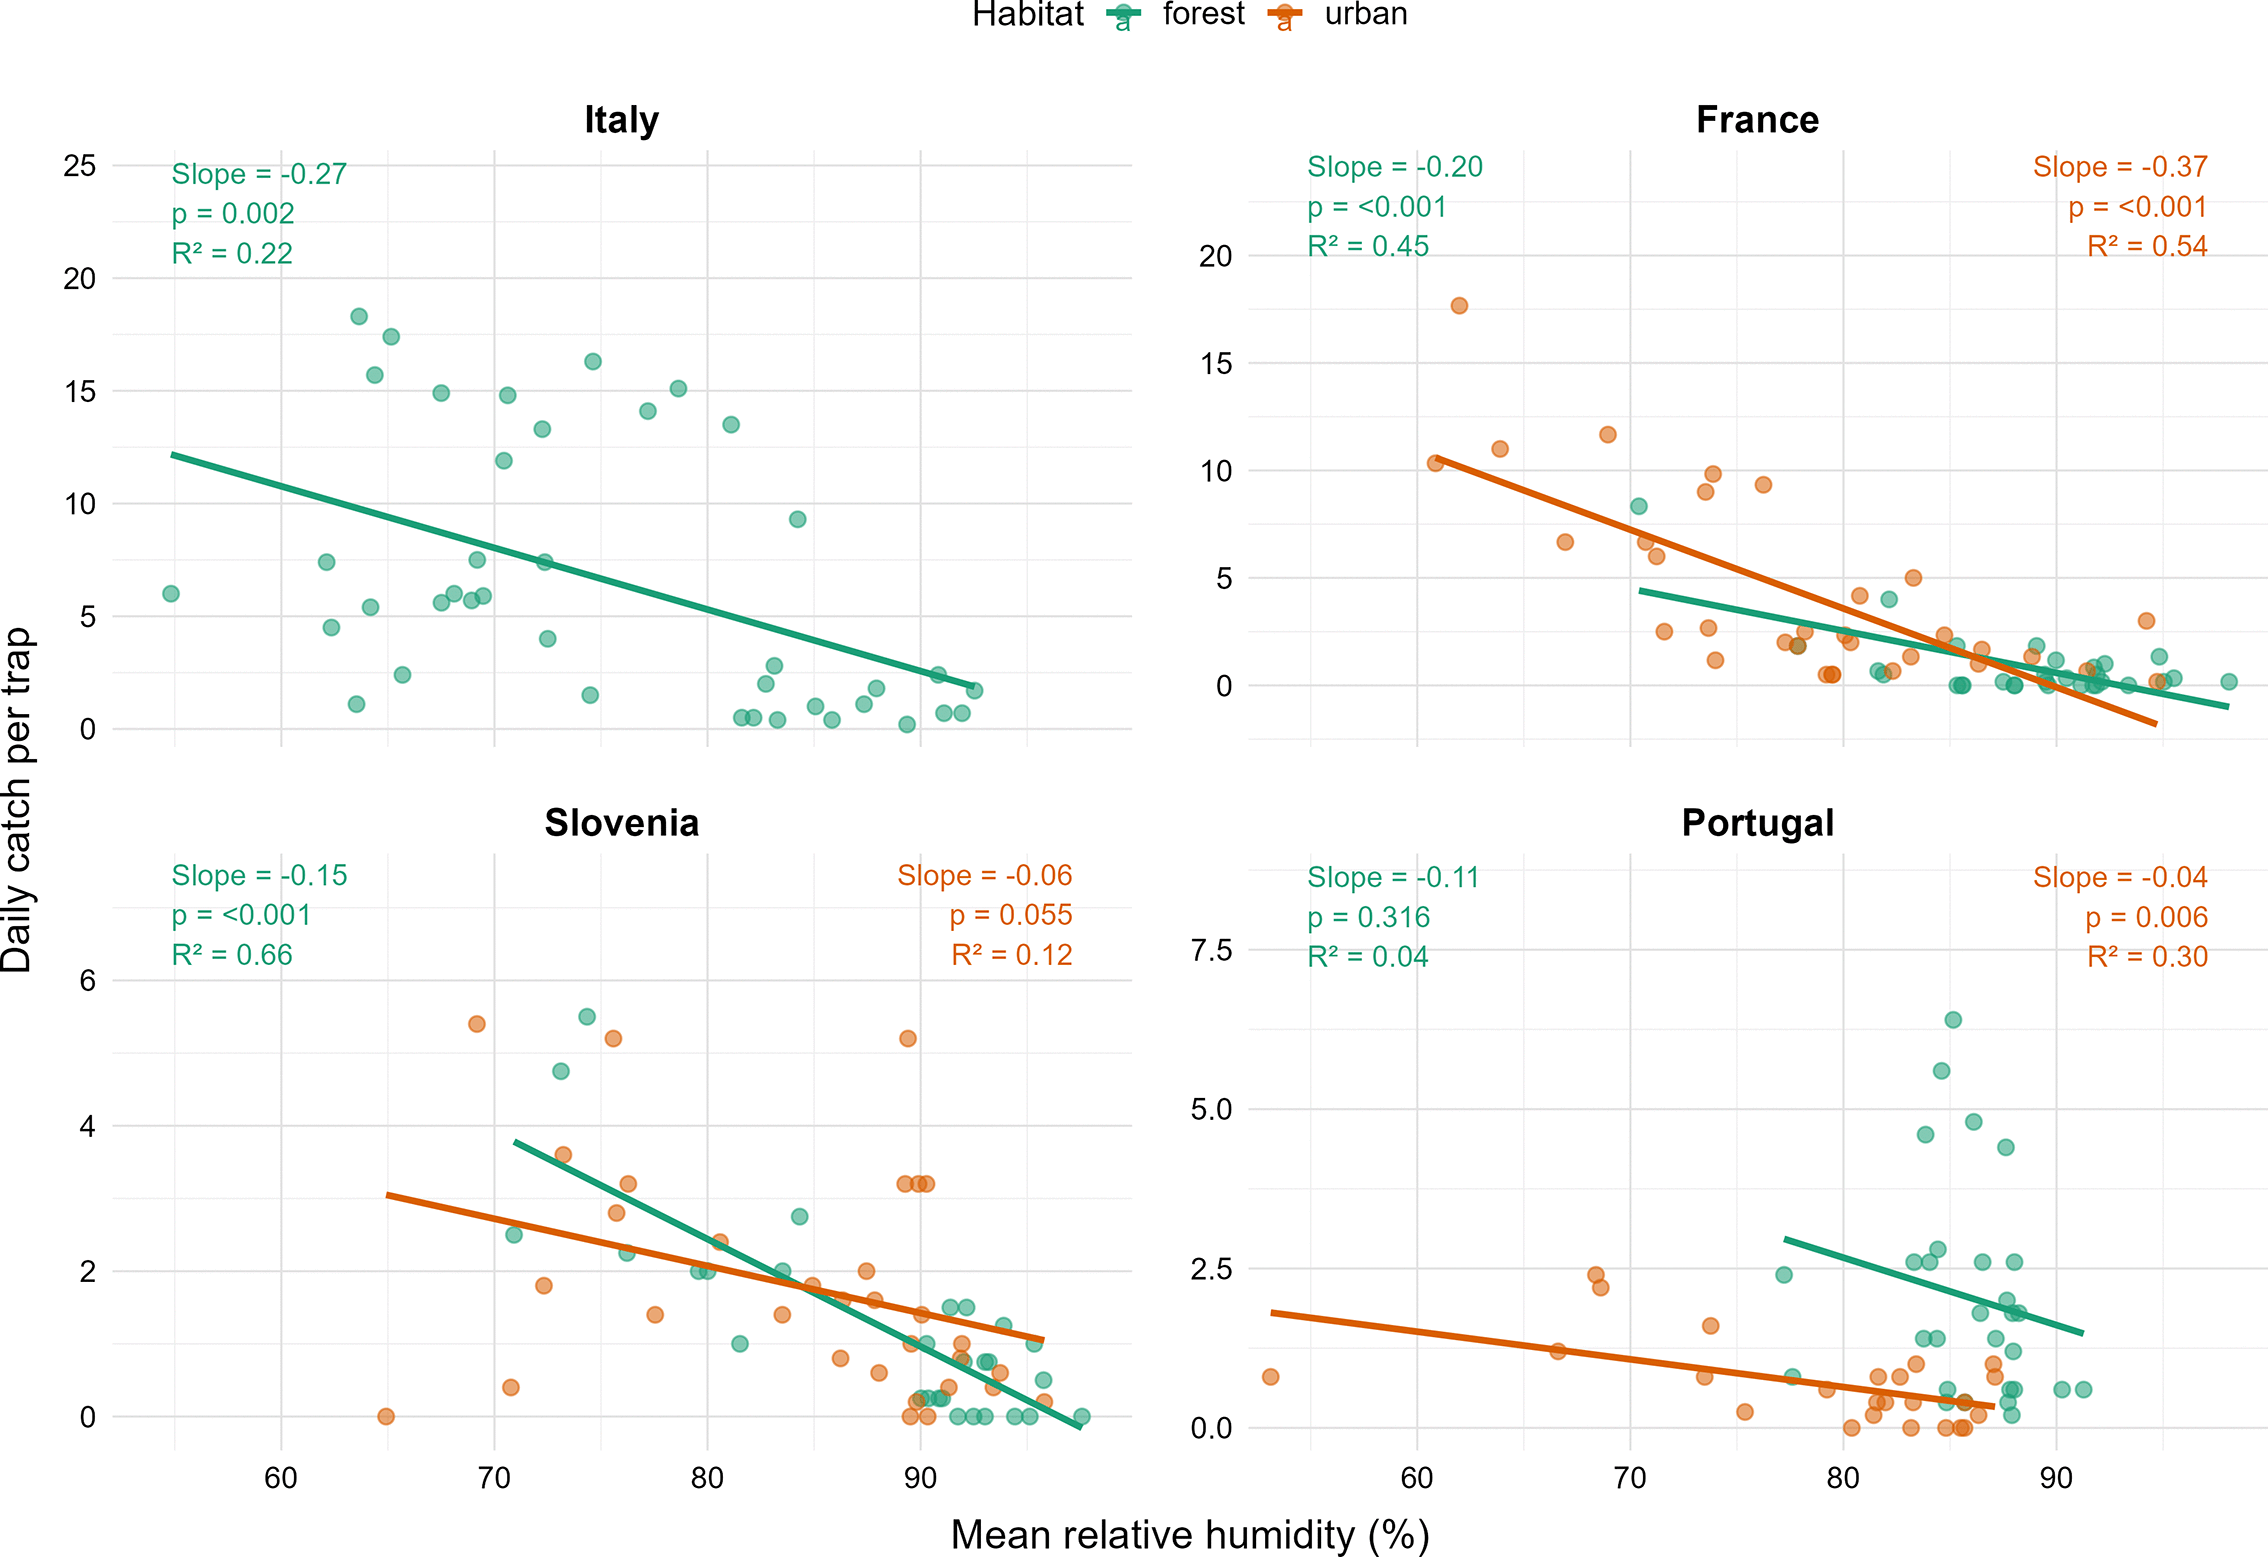
Figure 5. Relationships between relative humidity and trap catch during the central flight period (20–80% quantile).
Linear regression analyses revealed positive relationships between total trap catch and nest density (nests ha−1) for both automated (R2 = 0.48, P < 0.001) and conventional traps (R2 = 0.45, P = 0.003) when data from France and Italy were pooled (
Figures 6).
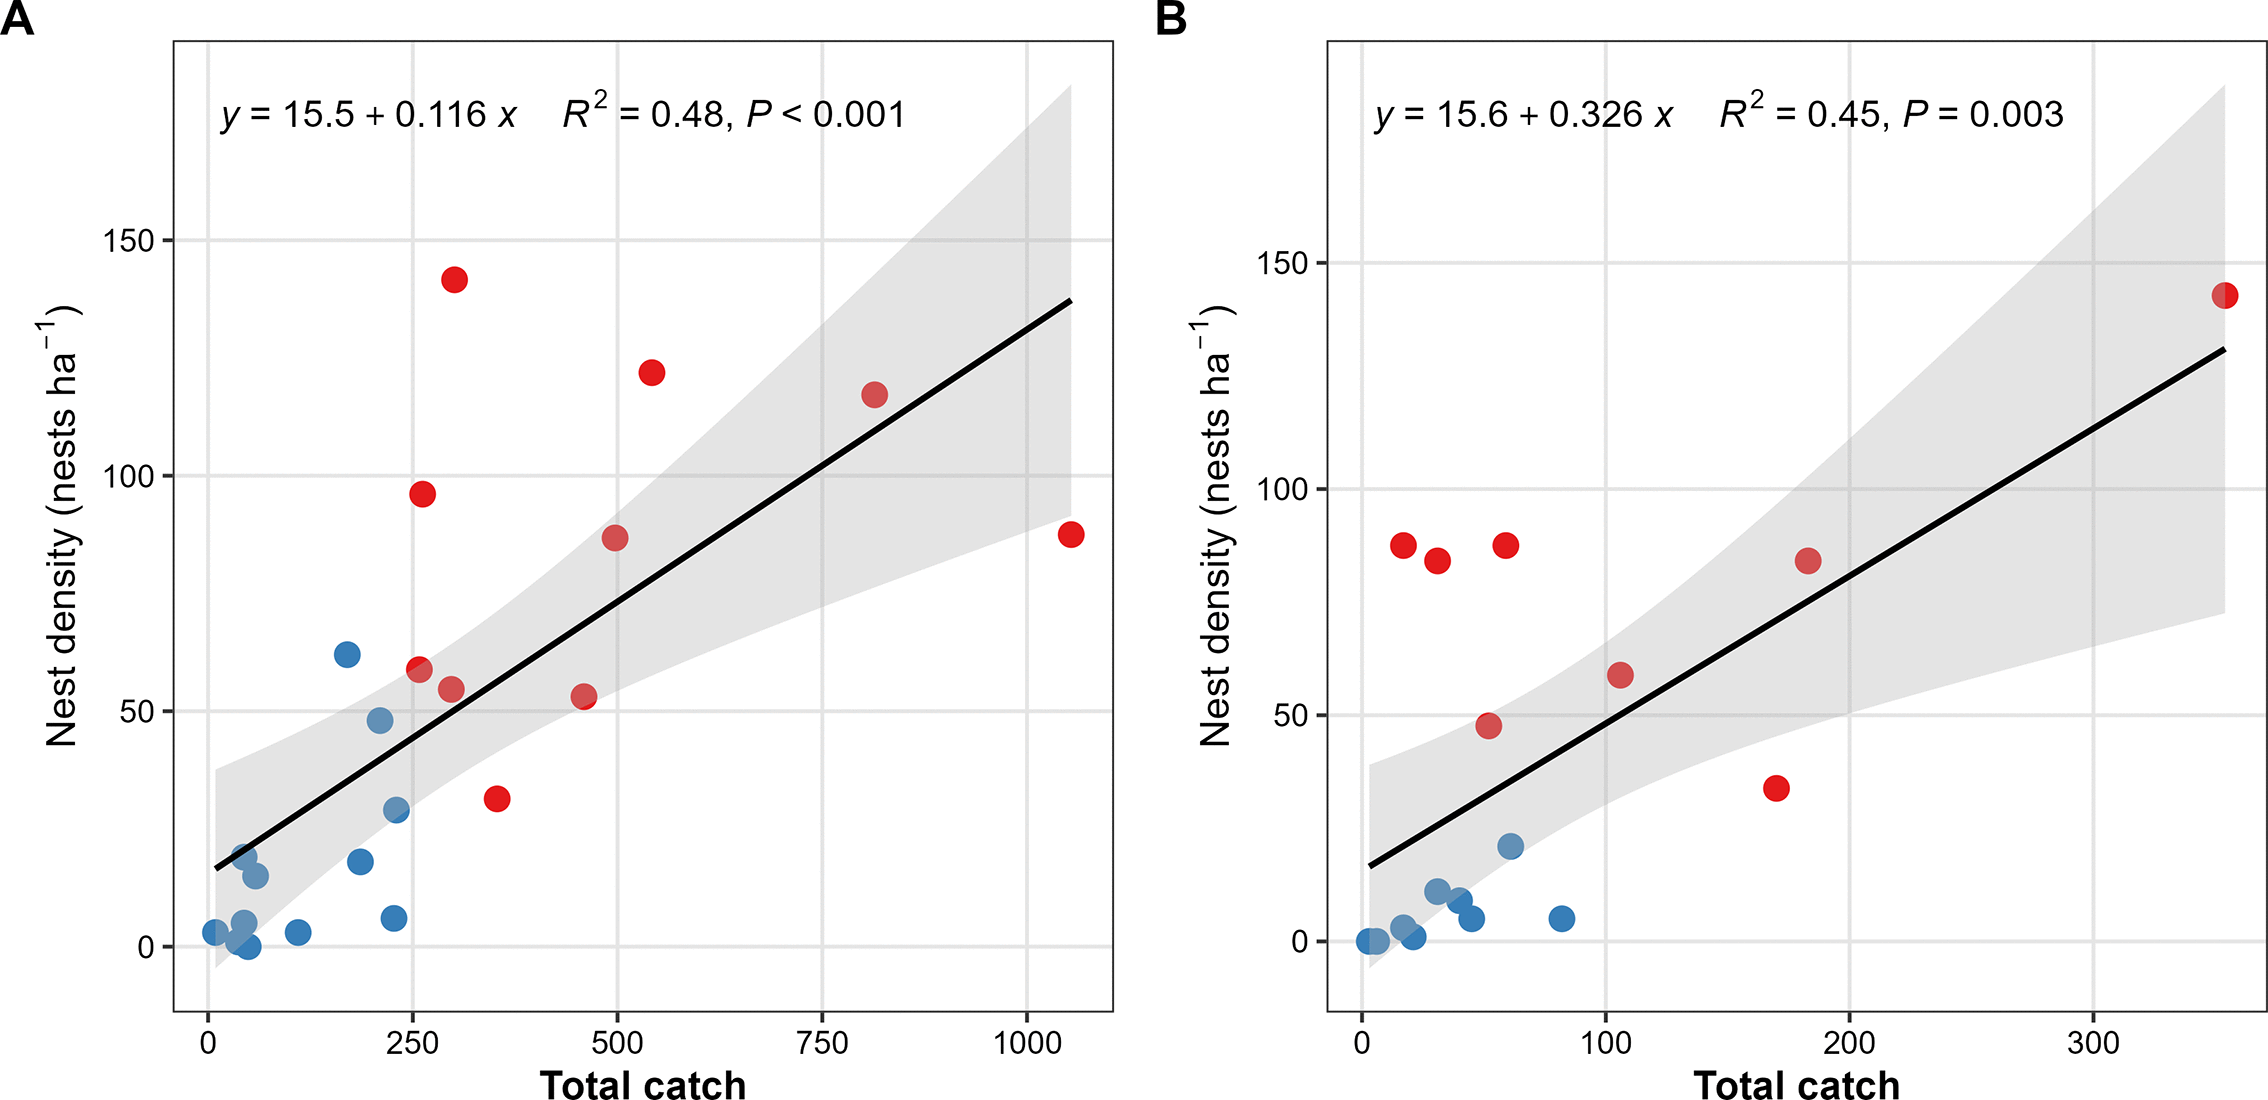
Figure 6. Relationships between total trap catch and nest density for automated (A) and conventional (B) traps.
Data from France (blue dots) and Italy (red dots) were pooled for each trap type.
Non-target catch in automated traps in Italy were generally low, ranging from 36 to 145 individuals per trap during the whole flight period (1.9–4.7 individuals per day). Notably, the highest number of non-target captures was recorded at the site with the highest moth catches, whereas the lowest number of non-target captures occurred at the site with the lowest moth catch. Diptera was the dominant non-target group at all sites, representing approximately 58–79% of captures. Leafhoppers and parasitoids were the second most abundant groups depending on the site, whereas ants, bees, beetles, grasshoppers, small moths, and spiders occurred only sporadically. Only rare cases of predation were observed (3 moths were predated by grasshoppers). Non-target captures recorded in conventional traps in Portugal were dominated by Diptera (77.9%) in forest habitats and by Hymenoptera, particularly the Asian hornet Vespa velutina (51.2%), in urban habitats. Several other arthropod groups were also recorded, although generally at low frequencies (forest: beetles, true bugs, moths, spiders; urban: beetles, dragonflies, true bugs). Predation could be reliably assessed only on images of automated traps, and occasionally during the checks of conventional traps. For automated traps in Portugal, only a few cases of predation were observed. Ants were observed on captured moths in two forest traps, predating three individuals in one trap and two in another. A wasp was also observed on a sticky surface, but no evidence of predation was detected in this case.
Discussion
Our results demonstrated that automated traps consistently captured more moths than conventional traps throughout most of the sites, with the exception of Slovenian ones where the trend was similar, although not significant. This can be explained by local variability and low population density rather than reduced performance of the automated trap. Detecting differences between monitoring methods becomes increasingly difficult when target populations are very low because trap catches are dominated by stochastic variation and the probability of capture is inherently low (Venette et al., 2002; Miller, 2020). Moreover, forest insect populations are often spatially heterogeneous, with variation in stand structure and local microclimatic conditions contributing to considerable differences among neighbouring traps (Petrovskaya et al. 2018). Under such conditions, variability among sampling sites may mask plausible differences in trap performance, particularly when the number of monitored sites is limited. Similar density-dependent effects have recently been demonstrated by Taylor and Tobin (2025), who showed that the relative performance of trapping systems varies with pest density and that distinguishing trap efficiency becomes increasingly difficult at low population levels.
The greater trapping performance of automated traps most likely resulted from the combined effects of its trap design and automated imaging system. Unlike conventional traps, where captured insects remain in the collector for a week or more, automated traps record moth catch daily and automatically renews the sticky surface. Consequently, insects are recorded before deterioration by scavengers, predation or escape can occur, whereas conventional traps may underestimate catches because specimens remain exposed to these processes between inspections (Howse et al., 2013). Similar advantages of automated monitoring have been reported for agricultural pests, where smart traps provide real-time information, improve temporal resolution and substantially reduce the labour associated with repeated field inspections (Ortis et al., 2025; Preti et al., 2021). Our study demonstrated that these advantages also apply to forest Lepidoptera monitored over broad geographical scales.
Besides improving surveillance performance, automated traps appear to be more ecologically selective for non-target organisms and predators. The moths caught every night are wrapped up in the sticky paper roll inside the trap and are becoming dry and inaccessible, while in conventional traps are just accumulating in the bucket, getting wet with rain and releasing odours that are attracting predators and scavengers. This ultimately affect the count of the individuals when the operator is checking the bucket once per week, resulting in the large underestimation of the catch shown by the comparison between automated and conventional traps.
Reliable automated species identification is essential for the operational deployment of AI-based monitoring systems. As ecological surveys and remote sensing platforms generate ever-larger volumes of imagery, audio recordings and videos, manual identification has become a serious bottleneck for biodiversity research and conservation practice (Christin, Hervet, et Lecomte, 2019). Our manual validation revealed excellent performance of the Faster R-CNN recognition algorithm, with consistently high precision, recall, F1-score and overall accuracy under both low- and high-density conditions. Unlike the initial validation conducted by TrapView company, which was based on a limited number of images collected during the early installation phase, our evaluation covered the complete Portuguese flight season using all deployed traps, providing a comprehensive assessment under realistic field conditions. The high accuracy achieved in our study is consistent with recent advances in AI-based image recognition for insect monitoring. Similar camera-based systems have reported F1-scores of 0.93 for moth classification (Bjerge et al., 2021), counting accuracies of 97.9% for Matsucoccus thunbergianae using Faster R-CNN (Hong et al., 2021), and classification accuracies between 82 and 99% for vineyard pests using deep-learning models (SDD ResNet50, Faster R-CNN ResNet101, etc.) (Gonçalves et al., 2022). Recent reviews further indicate that image-based deep-learning systems commonly achieve accuracy exceeding 90% for Lepidopteran pests under field conditions (Passias et al., 2024; Cardim Ferreira Lima et al., 2020; Roy et al., 2024). Most classification errors occurred during peaks of moth abundance and were associated with overlapping individuals, accumulation of wing prints on the sticky paper, or the very few non-target moths captured by the traps that shared similar morphological characteristics. Similar limitations have been reported in other camera-based monitoring systems, where image occlusion and morphological similarity between species remain the principal sources of misclassification (Bjerge et al., 2021; Roy et al., 2024; Saradopoulos et al., 2023). Nevertheless, these errors remained infrequent and had little influence on overall monitoring performance, indicating that only minimal manual verification is required. Furthermore, the permanent archive of trap images allows doubtful detections to be rapidly verified while simultaneously providing additional annotated data for the continuous improvement of the recognition model.
One of the most important outcomes of this study was the substantially higher probability of detecting moth activity during the beginning of the flight season. Across most countries, automated traps detected adult moths more frequently than conventional traps during periods of low flight activity, when only a few individuals were present. Likewise, first detections generally occurred several days earlier in automated than in conventional traps. These improvements are particularly important because surveillance programmes often aim to detect the onset of adult emergence rather than periods of peak abundance. Early detection is especially relevant for species whose geographical distribution continues to expand towards higher latitudes and elevations in response to climate warming, as for pine processionary moth (Battisti et al., 2005; Robinet et al., 2007). Newly established populations typically occur at low densities, making them difficult to detect using traditional surveillance methods. Failure to detect these populations early may delay management interventions and allow infestations to become established. The greater sensitivity of automated traps therefore represents an important advantage for monitoring programmes operating near the expanding range of species, where rapid detection is essential for delimiting newly colonized areas and tracking distributional changes over time.
Improved temporal resolution is another major advantage of automated monitoring. Weekly inspections, which remain standard practice in conventional trapping methods, inevitably delay access to field data and limit the precision with which flight phenology can be characterized. Automated traps overcome this limitation by providing daily observations throughout the flight season, supporting more accurate characterization of emergence patterns and population dynamics. Similar gains have recently been demonstrated for eastern spruce budworm (Choristoneura fumiferana), where automated pheromone trap networks have enabled the detection of immigration events and substantially improved the temporal resolution of dispersal studies (Dargent et al., 2023). Comparable benefits have been reported for agricultural pests, where daily image transmission has been shown to overcome the delays and labour costs associated with weekly manual inspections, allowing pest management decisions to be based on real-time pest activity rather than retrospective data (Preti et al., 2021). Beyond supporting forest pest management, automated monitoring networks capable of continuously transmitting standardized observations across broad geographical areas could also contribute to long-term ecological studies investigating shifts in phenology, dispersal and species distributions under future climate change scenarios, and decision-making tools by coupling automated trapping and phenology modelling.
Understanding the environmental factors regulating adult flight activity is essential for improving surveillance programmes and predicting periods of peak moth activity (Jonason et al., 2014). A further advantage of automated traps is that they enable the collection of meteorological data in real time, synchronously with trap catch. Temperature and relative humidity have long been recognized as major determinants of nocturnal flight in Lepidoptera, influencing both flight initiation and dispersal behaviour (Battisti et al., 2006; Greenbank, Schaefer, et Rainey, 1980). Consistent with previous studies, our results showed that temperature generally promoted pine processionary moth activity, although the magnitude and even the direction of this relationship varied among countries and habitats. This pattern agrees with the well-established dependence of nocturnal moth activity on sufficiently warm temperatures to sustain flight muscle activity, a process achieved through preflight shivering of the major flight muscles (Crespo, Vickers, et Goller, 2014). Increased temperatures reduce energetic constraints associated with flight and generally enhance dispersal capacity, explaining the higher numbers of moths captured during warmer nights (Crespo et al., 2014). However, Portugal showed contrasting responses between habitats. While urban populations exhibited the expected positive relationship between temperature and moth activity, forest populations showed a significant negative relationship. This result probably reflects differences in local microclimatic conditions rather than contrasting physiological responses. During the Portuguese summer, forest temperatures frequently remained within or above the thermal optimum for flight, meaning that further increases in temperature may have reduced activity because of increased thermal stress or lower nocturnal humidity. Forest stands also create distinct microclimates through canopy cover, reduced wind speed and altered heat exchange, which may influence flight behaviour differently from open urban environments (Wenda et al., 2025). These results emphasize that habitat-specific microclimates should be considered when interpreting climatic effects on insect phenology. Relative humidity generally showed the opposite pattern, with higher humidity associated with reduced moth activity in most countries and habitats, suggesting that humid atmospheric conditions reduce adult flight performance. High humidity is frequently associated with reduced atmospheric stability, dew formation and increased probability of precipitation, all of which may limit nocturnal flight activity (Fetnassi et al., 2022). Nevertheless, humidity effects were weaker than temperature effects and were not significant in Portugal forest sites, while only a marginal relationship was observed in Slovenian urban habitats. These differences further illustrate that the influence of weather variables depends on local environmental conditions and probably reflects interactions between temperature, humidity, vegetation structure and local topography. Integrating these environmental measurements with yearly trapping data may ultimately improve predictive phenological models and contribute to forecasting adult emergence and subsequent larval development.
Both trapping systems showed remarkably similar positive significant relationships between total catch and nest density, despite the large differences in the absolute number of captured moths. In a large-scale validation using sticky traps in France, Italy and Portugal, Jactel et al. (2006) also found significant positive correlations between mean daily male catches and winter nest density across all study regions. Similar findings were reported for the closely related oak processionary moth, which revealed a consistent linear relationship between square-root transformed adult males per trap and cube-root transformed numbers of larval nests (Straw et al., 2019).
Both traps rely on the same synthetic sex pheromone and therefore sample the same population of dispersing males, consequently, it is expected that both trapping systems would respond similarly to changes in population density, even if their capture efficiency differs. In their study Athanassiou et al. (2017) found positive and significant correlations among captures of T. pityocampa in pairs of different trap devices, and confirmed that most designs tracked the same population fluctuations. In our study, the substantially higher catches of the automated trap therefore reflect more efficient sampling of the available male population rather than greater predictive ability. Trap catches explained approximately half of the variation in nest density (R2 = 0.45–0.48), indicating that factors acting after adult flight may also contribute substantially to the final level of infestation. Adult abundance represents only the starting point of a complex sequence of demographic processes occurring between summer flight and winter nest assessment. Embryonic mortality, predation, parasitism, climatic conditions during egg development, larval survival and host tree quality all influence the number of nests ultimately observed. Consequently, these intervening demographic processes introduce additional variability in nest density and larval phenology beyond that explained by adult abundance alone. Such processes are widely recognised as important drivers of forest insect population dynamics (e.g., Jactel et al., 2006).
Estimating nest density is inherently difficult and prone to bias, particularly in mature pine stands where nests may be partially concealed within irregular tree crowns, introducing unavoidable observer error. These challenges were especially evident in Portugal and Slovenia, where a high proportion of sites had no detectable nests despite adult moth captures, precluding a meaningful assessment of the relationship between trap catches and nest density in these countries. Overall, the consistent positive and significant relationships suggest that captures in automated traps broadly reflected local infestation trends and provide reliable evidence that automated trap monitoring can capture spatial variation in infestation levels. Further validation across a larger number of sites and infestation gradients, particularly in low-density populations and at the expanding edge of the species’ distribution, is needed to further evaluate the robustness and operational applicability of automated monitoring systems.
The advantages demonstrated by automated traps extend beyond improvements in trapping performance and have important implications for operational forest surveillance. Traditional monitoring programmes require regular visits to every trap location to retrieve catches, replace lures when necessary and manually count insects. For regional and national surveillance networks covering hundreds or thousands of monitoring sites, these repeated field inspections represent one of the largest components of monitoring costs. Camera-based automated traps substantially reduce this logistical burden by providing continuous remote access to trapping information while simultaneously increasing temporal resolution. This capability is particularly valuable for forest ecosystems, where monitoring sites are often located in remote or inaccessible areas. Automated surveillance allows managers to rapidly identify areas where moth activity has begun, optimize inspection schedules and concentrate field efforts only where intervention is required. Furthermore, because all observations are stored electronically, automated systems facilitate the development of large, standardized databases that can support long-term analyses of population dynamics, phenology and climate-driven distribution changes. Such datasets will become increasingly valuable as forest pests continue responding to environmental change throughout Europe. Although automated monitoring systems require substantially greater initial investment than conventional traps, the higher costs may be offset by substantial reductions in labour, travel expenses and inspection frequency, particularly in extensive monitoring programmes covering large geographical regions (Preti et al., 2021; Ortis et al., 2025). Future studies are therefore needed to quantify the long-term costs and benefits of automated monitoring under different surveillance scenarios to determine the conditions under which AI-based camera traps become more cost-effective than conventional approaches.
Conclusions
This study provides the first comprehensive evaluation of AI-based camera traps for monitoring the pine processionary moth across multiple European countries, habitats and population densities. Compared with conventional traps, automated traps consistently captured more moths, detected adult activity earlier, increased the probability of detection during the critical early stages of the flight season and maintained excellent automated identification accuracy. In addition, the system reduced non-target captures compared with conventional traps and continuously transmitted monitoring information without requiring regular field inspections. Overall, these findings demonstrate that AI-based camera traps represent a major advance in forest pest surveillance. Their combination of high detection sensitivity, reliable automated identification, remote data transmission and ecological monitoring provides significant advantages over conventional trapping methods and offers new opportunities for large-scale surveillance programmes. As climate change continues to alter the distribution and phenology of this and other forest pests, automated monitoring systems have the potential to become key components of future forest health monitoring networks, supporting earlier detection, more informed management decisions and improved understanding of pest population dynamics in a changing climate.
Ethics and consent
Ethical approval and consent were not required for this work.
Data availability
Underlying data
Zenodo: Large testing of AI-based camera traps on a forest defoliating pest in Europe. Version 1 (V1) [Dataset]. FORSAID. https://doi.org/10.5281/zenodo.22735263 (Bourougaaoui et al., 2026).
The project contains the following underlying data:
-
compiled_data_all_countries.xlsx (compiled daily trap catches and nightly temperature and relative humidity data used in the statistical analyses).
-
Nest_density_per_ha_France_Italy.xlsx (winter nest density per hectare associated with the sampling sites and trap types in France and Italy).
-
raw_data_flight_France.zip (raw flight-monitoring data from individual traps in France, including daily datasets obtained by summing catches from the three automated images captured each day).
-
raw_data_flight_Italy.zip (raw flight-monitoring data from individual traps in Italy, including daily datasets obtained by summing catches from the three automated images captured each day).
-
raw_data_flight_Portugal.zip (raw flight-monitoring data from individual traps in Portugal, including daily datasets obtained by summing catches from the three automated images captured each day).
-
raw_data_flight_Slovenia.zip (raw flight-monitoring data from individual traps in Slovenia, including daily datasets obtained by summing catches from the three automated images captured each day).
-
raw_hourly_climate_data_France.zip (raw hourly temperature and relative humidity data recorded by automated traps in France).
-
raw_hourly_data_Italy.zip (raw hourly temperature and relative humidity data recorded by automated traps in Italy).
-
raw_hourly_climate_data_Portugal.zip (raw hourly temperature and relative humidity data recorded by automated traps in Portugal).
-
raw_hourly_climate_data_Slovenia.zip (raw hourly temperature and relative humidity data recorded by automated traps in Slovenia).
Acknowledgements
The authors acknowledge the contribution by entomologists and foresters who provided substantial help for carrying out the field work, namely the Forest Service of Schlanders/Silandro in Italy, Charles Genève, Benoît Nusillard, Aurore Mignan, Miguel Landum for their assistance in the fieldwork.
References
- Albanese A, Nardello M, Brunelli D:
Automated pest detection with DNN on the edge for precision agriculture.
IEEE J. Emerg. Sel. Top. Circuits Syst.
2021; 11(3): 458–467. Publisher Full Text
- Athanassiou CG, Kavallieratos NG, Pardo D, et al.:
Evaluation of pheromone trap devices for the capture of Thaumetopoea pityocampa (Lepidoptera: Thaumetopoeidae) in Southern Europe.
J. Econ. Entomol.
2017; 110(3): 1087–1095. PubMed Abstract
| Publisher Full Text
- Battisti A:
Field studies on the behaviour of two egg parasitoids of the pine processionary moth Thaumetopoea pityocampa.
Entomophaga.
1989; 34(1): 29–38. Publisher Full Text
- Battisti A, Stastny M, Netherer S, et al.:
Expansion of geographic range in the pine processionary moth caused by increased winter temperatures.
Ecol. Appl.
2005; 15(6): 2084–2096. Publisher Full Text
- Battisti A, Stastny M, Buffo E, et al.:
A rapid altitudinal range expansion in the pine processionary moth produced by the 2003 climatic anomaly.
Glob. Chang. Biol.
2006; 12(4): 662–671. Publisher Full Text
- Battisti A, Avcı M, Avtzis DN, et al.:
Natural history of the processionary moths (Thaumetopoea spp.): New insights in relation to climate change.Roques A, editor.
Processionary moths and climate change: An update.
Springer;
2015; pp. 15–79. Publisher Full Text
- Battisti A, Larsson S, Roques A:
Processionary moths and associated urtication risk: Global change–driven effects.
Annu. Rev. Entomol.
2017; 62: 323–342. Publisher Full Text
- Bjerge K, Nielsen JB, Sepstrup MV, et al.:
An automated light trap to monitor moths (Lepidoptera) using computer vision-based tracking and deep learning.
Sensors.
2021; 21(2): 343. PubMed Abstract
| Publisher Full Text
| Free Full Text
- Bourougaaoui A, Ben Jamâa ML, Robinet C:
Has North Africa turned too warm for a Mediterranean forest pest because of climate change?
Clim. Chang.
2021; 165(3): 46. Publisher Full Text
- Bourougaaoui A, de Groot M , Deveza T, et al.:
Large testing of AI-based camera traps on a forest defoliating pest in Europe. [Dataset].
Zenodo.
2026. Publisher Full Text
- Brunelli D, Polonelli T, Benini L:
Ultra-low energy pest detection for smart agriculture.
2020 IEEE Sensors.
IEEE;
2020; pp. 1–4. Publisher Full Text
- Cardim Ferreira Lima M, Damascena de Almeida Leandro ME, Valero C, et al.:
Automatic detection and monitoring of insect pests—A review.
Agriculture.
2020; 10(5): 161. Publisher Full Text
- Carus S:
Effects of defoliation caused by the processionary moth on growth of Crimean pines in western Turkey.
Phytoparasitica.
2009; 37(2): 105–114. Publisher Full Text
- Christin S, Hervet É, Lecomte N:
Applications for deep learning in ecology.
Methods Ecol. Evol.
2019; 10(10): 1632–1644. Publisher Full Text
- Crespo JG, Vickers NJ, Goller F:
Male moths optimally balance take-off thoracic temperature and warm-up duration to reach a pheromone source quickly.
Anim. Behav.
2014; 98: 79–85. PubMed Abstract
| Publisher Full Text
| Free Full Text
- Dargent F, Candau J-N, Studens K, et al.:
Characterizing eastern spruce budworm’s large-scale dispersal events through flight behavior and stable isotope analyses.
Front. Ecol. Evol.
2023; 11: 1060982. Publisher Full Text
- Elkinton JS, Cardé RT:
The use of pheromone traps to monitor distribution and population trends of the gypsy moth.Mitchell ER, editor.
Management of insect pests with semiochemicals: Concepts and practice.
Springer;
1981; pp. 41–55. Publisher Full Text
- EPPO:
EPPO Standards PM 7/37: Thaumetopoea pityocampa. Bulletin OEPP/EPPO Bulletin.2004; 34: 295–297. Publisher Full Text
- Fetnassi N, Ude K, Kull A, et al.:
Weather sensitivity of sugar bait trapping of nocturnal moths: A case study from Northern Europe.
Insects.
2022; 13(12): 1087. Publisher Full Text
- Flórián N, Jósvai JK, Tóth Z, et al.:
Automatic detection of moths (Lepidoptera) with a funnel trap prototype.
Insects.
2023; 14(4): 381. PubMed Abstract
| Publisher Full Text
| Free Full Text
- Georgiev G, Georgieva M, Zaemdzhikova G, et al.:
Flight characteristics of the summer and winter phenological form of the pine processionary moth (Thaumetopoea pityocampa) according to data from automatic pheromone traps near Asenovgrad in Bulgaria.
Silva Balcanica.
2025; 26(1): 13–22. Publisher Full Text
- Gonçalves J, Silva E, Faria P, et al.:
Edge-compatible deep learning models for detection of pest outbreaks in viticulture.
Agronomy.
2022; 12(12): 3052. Publisher Full Text
- Greenbank DO, Schaefer GW, Rainey RC:
Spruce budworm (Lepidoptera: Tortricidae) moth flight and dispersal: New understanding from canopy observations, radar, and aircraft.
Memoirs of the Entomological Society of Canada.
1980; 112(S110): 1–49. Publisher Full Text
- Hamza PF, Abbas A, Ketting P, et al.:
Biosecurity responses to fall armyworm (Spodoptera frugiperda) in Ghana and Australia: Comparative analysis and practical implications.
NeoBiota.
2026; 107: 155–174. Publisher Full Text
- Hong S-J, Nam I, Kim S-Y, et al.:
Automatic pest counting from pheromone trap images using deep learning object detectors for Matsucoccus thunbergianae monitoring.
Insects.
2021; 12(4): 342. PubMed Abstract
| Publisher Full Text
| Free Full Text
- Howse P, Stevens JM, Jones OT:
Insect pheromones and their use in pest management.
Springer Science & Business Media;
2013.
- Huchon H, Démolin G:
La biologie de la processionnaire du pin: Dispersion potentielle, dispersion actuelle.
Rev. For. Fr.
1970; 22: 220–234. Publisher Full Text
- Jactel H, Menassieu P, Vétillard F, et al.:
Population monitoring of the pine processionary moth (Lepidoptera: Thaumetopoeidae) with pheromone-baited traps.
For. Ecol. Manag.
2006; 235(1): 96–106. Publisher Full Text
- Jonason D, Franzén M, Ranius T:
Surveying moths using light traps: Effects of weather and time of year.
PLoS One.
2014; 9(3): e92453. PubMed Abstract
| Publisher Full Text
| Free Full Text
- Kammar V, Rani AT, Kumar KP, et al.:
Light trap: A dynamic tool for data analysis, documenting, and monitoring insect populations and diversity.Chakravarthy AK, editor.
Innovative pest management approaches for the 21st century: Harnessing automated unmanned technologies.
Springer;
2020; pp. 137–163. Publisher Full Text
- Kerdelhué C, Zane L, Simonato M, et al.:
Quaternary history and contemporary patterns in a currently expanding species.
BMC Evol. Biol.
2009; 9(1): 220. Publisher Full Text
- Miller JR:
Sharpening the precision of pest management decisions: assessing variability inherent in catch number and absolute density estimates derived from pheromone-baited traps monitoring insects moving randomly.
J. Econ. Entomol.
2020; 113(5): 2052–2060. Publisher Full Text
- Moneo I, Battisti A, Dufour B, et al.:
Medical and veterinary impact of the urticating processionary larvae.Roques A, editor.
Processionary moths and climate change: An update.
Springer;
2015; pp. 359–410. Publisher Full Text
- Novak M, Doležal P, Budík O, et al.:
Intelligent inspection probe for monitoring bark beetle activities using embedded IoT real-time object detection.
Eng. Sci. Technol. Int. J.
2024; 51: 101637. Publisher Full Text
- Ortis G, Duso C, Mori N:
New tools to monitor Scaphoideus titanus, the main vector of phytoplasmas associated with Flavescence dorée in vineyards.
Entomol. Exp. Appl.
2025; 173(4): 330–335. Publisher Full Text
- Passias A, Tsakalos K-A, Rigogiannis N, et al.:
Insect pest trap development and DL-based pest detection: A comprehensive review.
IEEE Trans. AgriFood Electron.
2024; 2(2): 323–334. Publisher Full Text
- Petrovskaya NB, Forbes E, Petrovskii SV, et al.:
Towards the development of a more accurate monitoring procedure for invertebrate populations, in the presence of an unknown spatial pattern of population distribution in the field.
Insects.
2018; 9(1): 29. PubMed Abstract
| Publisher Full Text
| Free Full Text
- Potamitis I, Eliopoulos P, Rigakis I:
Automated remote insect surveillance at a global scale and the Internet of Things.
Robotics.
2017; 6(3): 19. Publisher Full Text
- Preti M, Verheggen F, Angeli S:
Insect pest monitoring with camera-equipped traps: Strengths and limitations.
J. Pest. Sci.
2021; 94(2): 203–217. Publisher Full Text
- Ray RK, Chakravarty S, Dash S, et al.:
Precision pest management in agriculture using Inception V3 and EfficientNet B4: A deep learning approach for crop protection.
Inf. Process. Agric.
2026; 13(1): 142–161. Publisher Full Text
- Roberts NS, Ndayiragije JC, Özek T, et al.:
Visual modelling can optimise sticky trap design for simultaneous monitoring of multiple species of insect pests.
Sci. Rep.
2025; 15(1): 17280. PubMed Abstract
| Publisher Full Text
| Free Full Text
- Robinet C, Baier P, Pennerstorfer J, et al.:
Modelling the effects of climate change on the potential feeding activity of Thaumetopoea pityocampa (Den. & Schiff.) (Lepidoptera: Notodontidae) in France.
Glob. Ecol. Biogeogr.
2007; 16(4): 460–471. Publisher Full Text
- Roques A, Rousselet J, Avcı M, et al.:
Climate warming and past and present distribution of the processionary moths (Thaumetopoea spp.) in Europe, Asia Minor and North Africa.Roques A, editor.
Processionary moths and climate change: An update.
Springer;
2015; pp. 81–161. Publisher Full Text
- Rosenzweig C, Casassa G, Karoly DJ, et al.:
Assessment of observed changes and responses in natural and managed systems.Parry ML, Canziani OF, Palutikof JP, et al., editors.
Climate change 2007: Impacts, adaptation and vulnerability—Contribution of Working Group II to the Fourth Assessment Report of the Intergovernmental Panel on Climate Change.
Cambridge University Press;
2007; pp. 79–131.
- Rossi JP, Imbault V, Lamant T, et al.:
A citywide survey of the pine processionary moth Thaumetopoea pityocampa spatial distribution in Orléans (France).
Urban For. Urban Green.
2016; 20: 71–80. Publisher Full Text
- Roy DB, Alison J, August TA, et al.:
Towards a standardized framework for AI-assisted, image-based monitoring of nocturnal insects.
Philos. Trans. R. Soc. B: Biol. Sci.
2024; 379(1904): 20230108. PubMed Abstract
| Publisher Full Text
| Free Full Text
- Rydhmer K, Bick E, Still L, et al.:
Automating insect monitoring using unsupervised near-infrared sensors.
Sci. Rep.
2022; 12(1): 2603. PubMed Abstract
| Publisher Full Text
| Free Full Text
- Saradopoulos I, Potamitis I, Konstantaras AI, et al.:
Image-based insect counting embedded in e-traps that learn without manual image annotation and self-dispose captured insects.
Inform.
2023; 14(5): 267. Publisher Full Text
- Sbay H, Zas R:
Geographic variation in growth, survival, and susceptibility to the processionary moth (Thaumetopoea pityocampa Dennis & Schiff.) of Pinus halepensis Mill. and P. brutia Ten.: Results from common gardens in Morocco.
Ann. For. Sci.
2018; 75(3): 69. Publisher Full Text
- Sittinger M, Uhler J, Pink M, et al.:
Insect detect: An open-source DIY camera trap for automated insect monitoring.
PLoS One.
2024; 19(4): e0295474. Publisher Full Text
- Straw NA, Hoppit A, Branson J:
The relationship between pheromone trap catch and local population density of the oak processionary moth Thaumetopoea processionea (Lepidoptera: Thaumetopoeidae).
Agric. For. Entomol.
2019; 21(4): 424–430. Publisher Full Text
- Sütő J:
Embedded system-based sticky paper trap with deep learning-based insect-counting algorithm.
Electronics.
2021; 10(15): 1754. Publisher Full Text
- Taylor RAJ, Tobin PC:
Spatial distribution, sampling efficiency and Taylor’s power law: 3. Density-dependent efficiency in emerald ash borer sampling schemes.
Agric. For. Entomol.
2025; 27(3): 476–486. Publisher Full Text
- Venette RC, Moon RD, Hutchison WD:
Strategies and statistics of sampling for rare individuals.
Annu. Rev. Entomol.
2002; 47: 143–174. Publisher Full Text
- Welsh TJ, Bentall D, Kwon C, et al.:
Automated surveillance of lepidopteran pests with smart optoelectronic sensor traps.
Sustainability.
2022; 14(15): 9577. Publisher Full Text
- Wenda C, Luk C-L, Benedick S, et al.:
Butterflies respond to habitat disturbance in tropical forests through activity shifts.
J. Anim. Ecol.
2025; 94(7): 1361–1371. PubMed Abstract
| Publisher Full Text







